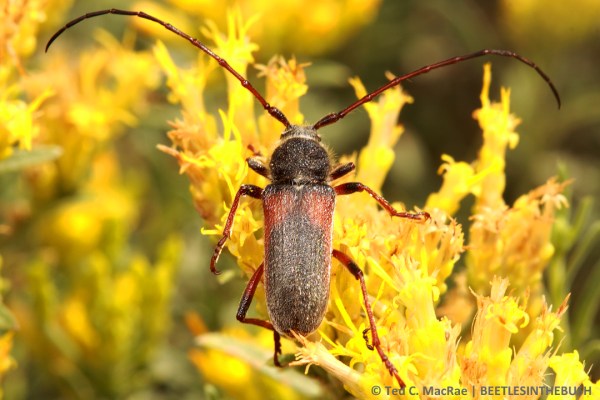
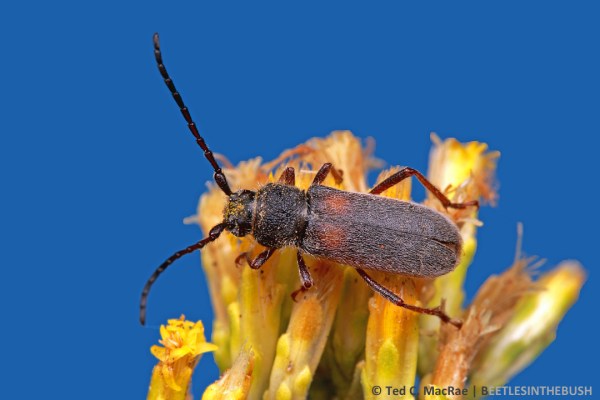
A Crossidius hirtipes subspecies blend zone…

…or, “There’s something fishy going on here!”

After a day in the vicinity of Yearington, Nevada  looking for (and eventually finding) a population of Crossidius hirtipes longhorned beetles assignable to subspecies “rubrescens“, field mate Jeff Huether and I dropped a little further south to look for two additional subspecies—C. h. immaculipennis and C. h. macswaini. Like C. h. rubrescens, populations assignable to these two subspecies are also restricted to a small area in west-central Nevada. Chemsak & Linsley (1959) described C. h. immaculipennis from specimens collected 10 miles north of Smith (Lyon Co.) and two years later (Linsley & Chemsak 1961) described C. h. macswaini from 19 miles SE of Wellington (Douglas Co.). We were still under the smoke plum from the now 9-day old Rim Fire in the nearby Sierra Nevada, which came and went during much of the day (top photo) and eventually settled in to create some amazing sunset landscapes (bottom photo).

19 mi S of Wellington, Toiyabe National Forest, Nevada.

Rim Fire smoke moves in and out of the area | 19 mi S of Wellington, Toiyabe National Forest, Nevada.

As had happened the day before with C. h. rubrescens, success did not come quickly or easily. We first searched for the type locality of C. h. immaculipennis, but many parts of the area have been converted to agriculture, and in the precise area 10 miles north of Smith we found only vast fields of dark green, irrigated alfalfa and not the rabbitbrush chaparral habitat required by these beetles. We did a little searching in surrounding areas and eventually found one rather nice-looking patch of ground with healthy stands of Chrysothamnus viscidiflorus in full bloom. Mindful of the previous day’s experience with finding the beetles often ensconced down within the inflorescences—especially as cooler temperatures set in, we took care to carefully inspect the blossoms in case the cool morning temperatures were inhibiting the beetles from coming back up for the day. Alas, we saw no beetles despite spending a considerable amount of time searching.

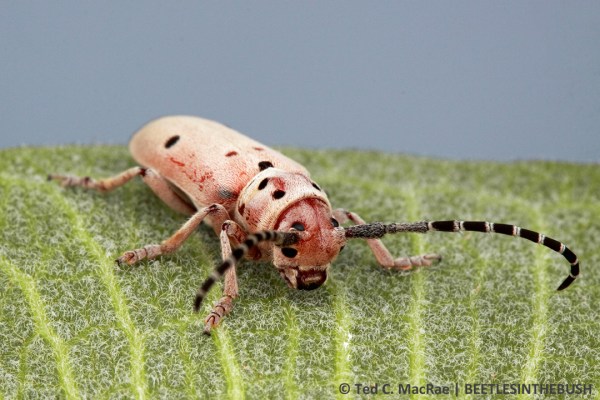
Crossidius hirtipes immaculipennis (male) | 6.3 mi W of Wellington, Nevada.

Crossidius hirtipes immaculipennis (male) | 6.3 mi W of Wellington, Nevada.

Rather than beat a dead horse, we decided to drive a short distance south and west to the town of Wellington, where a fellow cerambycid collector had found the subspecies a few years earlier. He had provided us with some detailed notes on the specific localities where he found the beetles, and these proved to be of great help as we passed through endless, seemingly acceptable chaparral habitat trying to decide exactly where we should stop and invest more time to look for the beetle. We stopped at one of the sites indicated in the notes and immediately found a beetle on one of the first plants we checked, and eventually after a gap in finding any more we found an area where good numbers of the plants were supporting decent numbers of the beetles. Chemsak & Linsley (1959) distinguished C. h. immaculipennis by its reddish legs, pale color, and complete lack of elytral markings in the male, exemplified by the male shown in the photo above.

Crossidius hirtipes macswainei? (female) | 6.3 mi W of Wellington, Nevada.

Crossidius hirtipes macswainei? (female) | 6.3 mi W of Wellington, Nevada.

As we searched the plants and found more and more individuals, I noticed an occasional adult that seemed to be a little more yellowish than reddish and with distinct sutural maculae. I didn’t think much about it then, chalking it up to individual variability, but after returning home and having a chance to look at the specimens more closely I was surprised to determine that these few beetles actually are a better fit for the second subspecies we planned to search for that day—C. h. macswainei. We had found both subspecies at the same site and didn’t even realize it. Okay, I know what you’re thinking… subspecies must exhibit allopatric geographic distributions (cannot occur together at the same place and time). It is, thus, tempting to declare that the two “subspecies” are actually not distinct, but rather represent distinctive extremes of individual variation in a single interbreeding population. However, one must also consider the possibility that the two subspecies represent reproductively isolated populations and, thus, qualify as distinct species. I’m not qualified to make that judgement, but I will note that most of the individuals encountered were assignable to C. h. immaculipennis  and the rest to C. h. macswainei, but that no “intergrades” were found.

Crossidius hirtipes macswainei (male) | 19 mi S of Wellington, Nevada.

Crossidius hirtipes rhodopus? (male) | 19 mi S of Wellington, Nevada.

After collecting adequate series from W of Wellington, we traveled further south of town to the type locality of C. h. macswainei (not knowing we already had it!). The holotype and most of the paratypes were collected 19 miles S of Wellington (Linsley & Chemsak 1961), but a number of paratypes had also been collected 14 miles south of town, so we stopped there first in an unsuccessful bid to find the subspecies before moving on to the type locality a few miles further south. Within a few minutes of arriving, I found the individual shown in the photo immediately above, presumed that I had found the subspecies we were looking for, and popped it into a vial alive as a photo backup if we did not find any other individuals with which I could attempt field photographs. Ironically, that is exactly what happened—despite Jeff and I scouring every plant we could find in about a 1-mile stretch along each side of the road, we never found another beetle. Later that evening I took the above individual out of its vial for photographs, but it never really “perked up” to look fully natural, resulting in “bum” antennae that give away the staged nature of the photograph. Again, it was not until I got back home and could look at the specimen closely before I realized that it did not at all fit the description of C. h. macswainei, but instead seemed to be a good match for the subspecies C. h. rhodopus, known from only a short distance further south but—until now, at least—apparently restricted to the Mono Basin in east-central California (see this post for more details about this subspecies). Jeff has since reported to me that some of the beetles he collected at the “C. h. rubrescens” locality (see this post) also are a match for C. h. macswainei, adding yet another wrinkle to those that resulted from this day’s collecting. Such inconsistencies with the published literature may tempt some to scrap all of Linsley & Chemsak’s subspecies, but considering that those two authors examined more than 12,000 specimens during the course of their studies such a reaction would be both premature and presumptuous. What is needed is more study—more specimens from more localities, hopefully augmented with DNA sequence analysis. For the latter goal we did our part, dropping a specimen or two from every locality in which we found beetles into ethanol for just such purpose. Until such studies are done, I prefer to withhold judgement about whether C. hirtipes is comprised of one highly polytopic population, several subspecifically distinct populations, or perhaps even multiple distinct species.
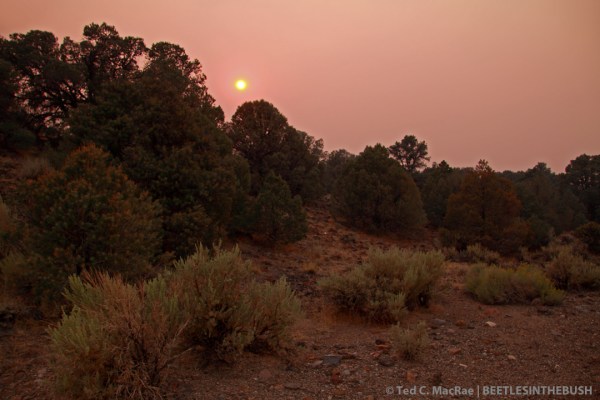
14 mi SE of Wellington, Toiyabe National Forest, Nevada.

Evening haze creates a spectacular sunset | 14 mi SE of Wellington, Toiyabe National Forest, Nevada.

Even though we found only a single beetle at the second locality, our persistence in searching until the day ran out was rewarded by a most spectacular sunset caused by thick haze from the nearby Rim Fire in California. It would also be our last day in Nevada before dropping south into California and spending the next several days in successful bids for C. coralinus monoensis, C. c. caeruleipennis, C. h. nubilus, and C. h. rhodopus.

REFERENCE:

Chemsak, J. A. & E. G. Linsley. 1959. Some new species and subspecies of Crossidius from western North America. Journal of the Kansas Entomological Society 32(4):176–183.

Linsley, E. G. & J. A. Chemsak. 1961. A distributional and taxonomic study of the genus Crossidius (Coleoptera, Cerambycidae). Miscellaneous Publications of the Entomological Society of America 3(2):25–64 + 3 color plates.

Copyright © Ted C. MacRae 2014
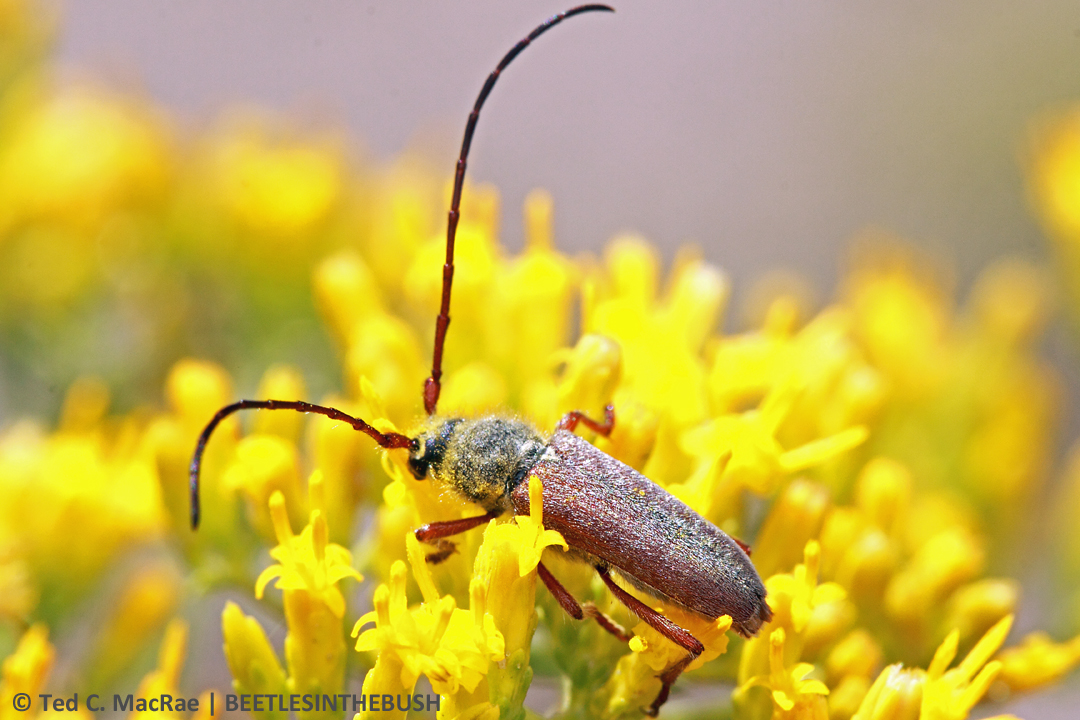
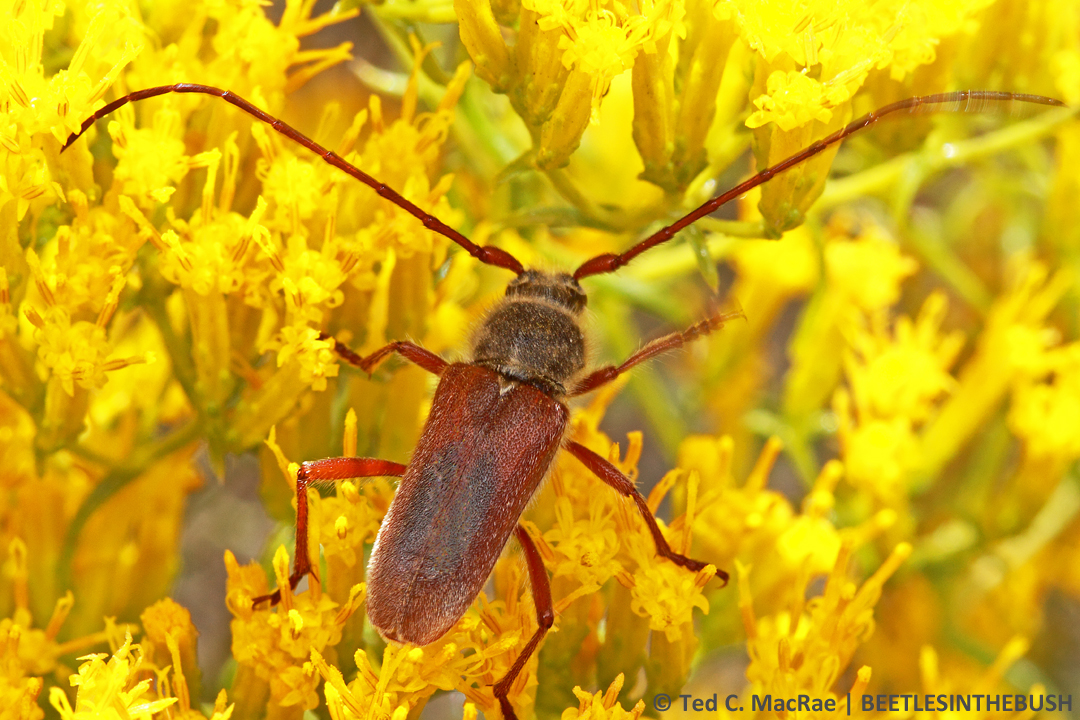
Crossidius hirtipes rhodopus in Adobe Valley, California

Crossidius hirtipes rhodopus | Adobe Valley, Mono Co., California

Crossidius hirtipes rhodopus Linsley, 1955 | Adobe Valley, Mono Co., California

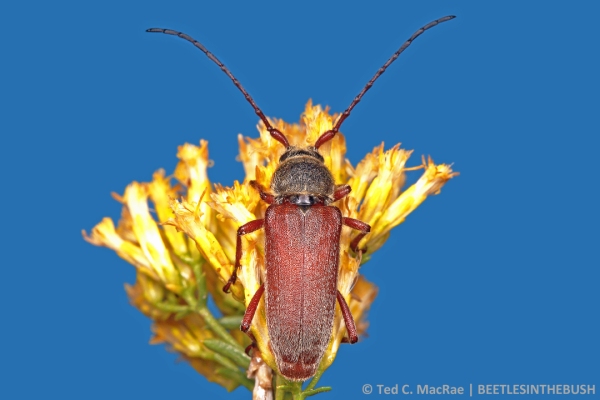
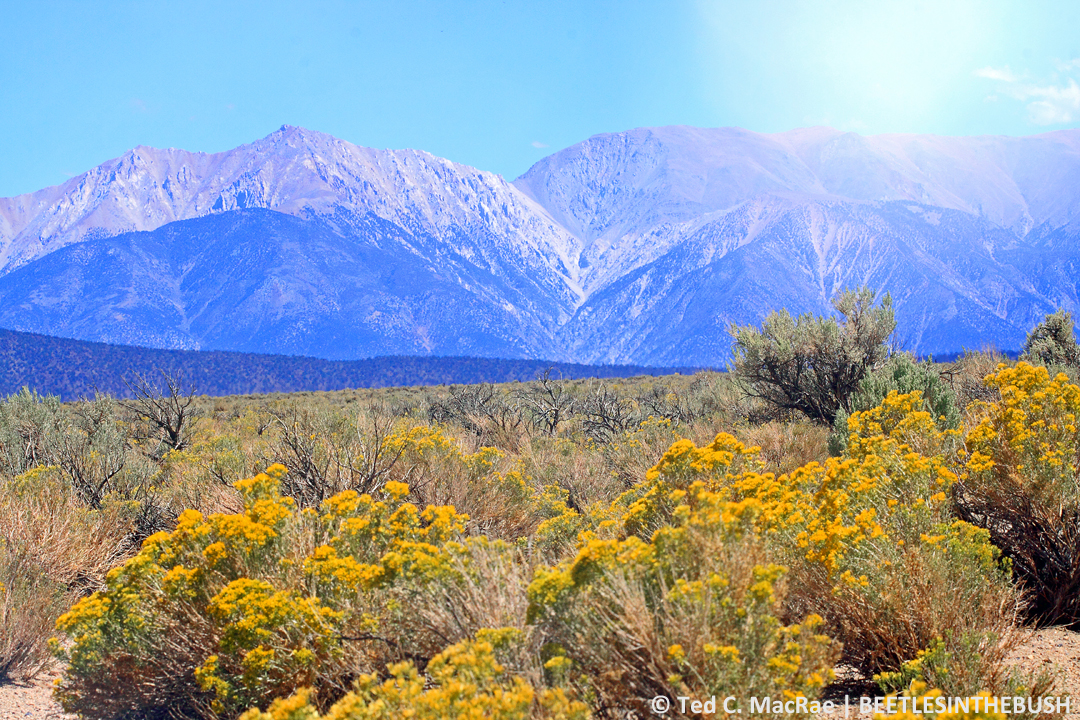
On Day 7 of last August’s Great Basin Collecting Trip, we left Bishop and headed back north to the Mono Basin to look for Crossidius hirtipes rhodopus, a distinctive reddish subspecies known only from the Mono Basin. I’d seen this beetle before—almost 20 years ago during one of several trips to the type locality of Nanularia monoensis (described by my late friend Chuck Bellamy in his 1987 revision of the genus), so we drove south of Mono Lake on Hwy 120 through Adobe Valley on our way to the Benton Range where I last saw them. Of course, C. h. rhodopus occurs more broadly in the Mono Basin than just the Benton Range, and as we drove through the valley we saw robust stands of the beetle’s host plant, yellow rabbitbrush (Chrysothamnus viscidiflorus), in full bloom stretching across the floor of the valley to the towering White Mountains in the distance. Impatience can sometimes be a virtue, and in this case our decision to stop and check the plants rather than waiting until we got to the Benton Range paid off—not only were the beetles out in force, allowing us to photograph and collect to our heart’s content, but we saw only a few beetles on but a single flowering plant during our subsequent visit to the Benton Range. Apparently the rains that had caused such a profusion of bloom in the Adobe Valley had not graced the Benton Range, resulting in the driest conditions I have seen during my several visits there.

This subspecies is one of the more darkly colored subspecies

This subspecies is one of the more darkly colored subspecies

Crossidius h. rhodopus is among the most distinctive of all the C. hirtipes subspecies due to its dark reddish-brown coloration. It closely resembles C. h. nubilus, which we had seen the day before at its only known locality further south at Westgaard Pass between the White and Inyo Mountains, but it is not as dark as that subspecies and lacks the extensive clouding of black on the apical portions of the elytra. The red-brown legs and brown antennae becoming darker at the tip further characterize C. h. rhodopus, originally described as a full species (Linsley 1955) but later regarded as a subspecies of the widely distributed and highly polytopic C. hirtipes LeConte, 1854 (Linsley & Chemsak 1961).

Yellow rabbitbrush (Chrysothamnus viscidiflorus) abounds in the valley, as the White Mountains loom in the background.

Yellow rabbitbrush (Chrysothamnus viscidiflorus) abounds below the magnificent White Mountains.

Those who are unfamiliar with the Mono Basin are missing one of California’s greatest natural treasures. A closed, internal-drainage basin bordered to the west by the massive Sierra Nevada Mountains (with Yosemite National Park lying just over the peaks), to the east by the Cowtrack Mountain, to the north by the Bodie Hills, and to the South by the north ridge of the Long Valley, the eerily beautiful Mono Lake is its most prominent feature. Do not, however, neglect other areas of the basin, which offer their own uniquely dramatic beauty. Adobe Valley, stretching south of the lake towards the White Mountains and famous for the wild mustang that live there, is one such area.

A handsome male rests on yellow rabbitbrush flowers (studio shot).

A robustly handsome female perches a terminal flower cluster of yellow rabbitbrush (studio shot).

REFERENCES:

Linsley, E. G. 1955. Notes and descriptions of some species of Crossidius. The Pan-Pacific Entomologist 31(2):63–66.

Linsley, E. G. & J. A. Chemsak. 1961. A distributional and taxonomic study of the genus Crossidius (Coleoptera, Cerambycidae). Miscellaneous Publications of the Entomological Society of America 3(2):25–64 + 3 color plates.

© Ted C. MacRae 2014

Beetle Collecting 101: How to rear wood-boring beetles

I’ve been collecting wood-boring beetles for more than three decades now, and if I had to make a list of “essential” methods for collecting them I would include “beating,” “blacklighting,” and “rearing.” Beating is relatively straightforward—take a beating sheet (a square piece of cloth measuring 3–5 ft across and suspended beneath wooden, metal, or plastic cross members), position it beneath a branch of a suspected host plant, and tap the branch with a stick or net handle. Many wood-boring beetles tend to hang out on branches of their host plants, especially recently dead ones, and will fall onto the sheet when the branch is tapped. Be quick—some species (especially jewel beetles in the genus Chrysobothris) can zip away in a flash before you have a chance to grab them (especially in the heat of the day). Others (e.g., some Cerambycidae) may remain motionless and are cryptically colored enough to avoid detection among the pieces of bark and debris that also fall onto the sheet with them. Nevertheless, persistence is the key, and with a little practice one can become quite expert at efficiently collecting wood-boring beetles using this method. Blacklighting is even easier—find the right habitat (preferably on a warm, humid, moonless night), set up a blacklight in front of a white sheet, crack open a brew, and wait for the beetles to come!

Rearing, on the other hand, takes true dedication. One must not only learn potential host plants, but also how to recognize wood with the greatest potential for harboring larvae, retrieve it from the field, cut it up, place it in rearing containers, and monitor the containers for up to several months or even years before hitting pay dirt (maybe!). Despite the considerable amount of effort this can take, the results are well worth it in terms of obtaining a diversity of species (usually in good series), some of which may be difficult to encounter in the field, and identifying unequivocal larval host associations. I have even discovered two new species through rearing (Bellamy 2002, MacRae 2003)! Moreover, checking rearing containers can be a lot of fun—in one afternoon you can collect dozens or even hundreds of specimens from places far and wide, depending on how far you are willing to travel to collect the wood. Because of the effort involved, however, the more you can do to ensure that effort isn’t wasted on uninfested wood and that suitable conditions are provided to encourage continued larval development and adult emergence from infested wood the better. It is with this in mind that I offer these tips for those who might be interested in using rearing as a technique for collecting these beetles.

I should first clarify what I mean by “wood-boring” beetles. In the broadest sense this can include beetles from any number of families in which the larvae are “xylophagous,” i.e., they feed within dead wood. However, I am most interested in jewel beetles (family Buprestidae) and longhorned beetles (family Cerambycidae), and as a result most of the advice that I offer below is tailored to species in these two families. That is not to say that I’ll turn down any checkered beetles (Cleridae), powderpost beetles (Bostrichidae), bark beetles (family Scolytidae), or even flat bark beetles sensu lato (Cucujoidea) that I also happen to encounter in my rearing containers, with the first two groups in particular having appeared in quite good numbers and diversity in my containers over the years. Nevertheless, I can’t claim that my methods have been optimized specifically for collecting species in these other families.

First, you have to find the wood. In my experience, the best time to collect wood for rearing is late winter through early spring. A majority of species across much of North America tend to emerge as adults during mid- to late spring, and collecting wood just before anticipated adult emergence allows the beetles to experience natural thermoperiods and moisture regimes for nearly the duration of their larval and pupal development periods. Evidence of larval infestation is also easier to spot once they’ve had time to develop. That said, there is no “bad” time to collect wood, and almost every time I go into the field I am on the lookout for infested wood regardless of the time of year. The tricky part is knowing where to put your efforts—not all species of trees are equally likely to host wood-boring beetles. In general, oaks (Quercus), hickories (Carya), and hackberries (Celtis) in the eastern U.S. host a good diversity of species, while trees such as maples (Acer), elms (Ulmus), locust (Gleditsia and Robinia), and others host a more limited but still interesting fauna. In the southwestern U.S. mesquite (Prosopis) and acacia (Acacia) are highly favored host plants, while in the mountains oaks are again favored. Everywhere, conifers (Pinus, Abies, Juniperus, Tsuga, etc.) harbor a tremendous diversity of wood-boring beetles. To become good at rearing wood-boring beetles, you have to become a good botanist and learn not only how to identify trees, but dead wood from them based on characters other than their leaves! Study one of the many good references available (e.g., Lingafelter 2007, Nelson et al. 2008) to see what the range of preferred host plants are and then start looking.

I wish it were as simple as finding the desired types of trees and picking up whatever dead wood you can findm but it’s not. You still need to determine whether the wood is actually infested. Any habitat supporting populations of wood-boring beetles is likely to have a lot of dead wood. However, most of the wood you find will not have any beetles in it because it is already “too old.” This is especially true in the desert southwest, where dead wood can persist for very long periods of time due to low moisture availability. Wood-boring beetles begin their lives as eggs laid on the bark of freshly killed or declining wood and spend much of their lives as small larvae that are difficult to detect and leave no obvious outward signs of their presence within or under the bark. By the time external signs of infestation (e.g., exit holes, sloughed bark exposing larval galleries, etc.) become obvious it is often too late—everything has already emerged. Instead, look for branches that are freshly dead that show few or no outward signs of infestation. You can slice into the bark with a knife to look for evidence of larval tunnels—in general those of longhorned beetles will be clean, while those of jewel beetles will be filled with fine sawdust-like frass that the larva packs behind it as it tunnels through the wood. Oftentimes the tunnels and larvae will be just under the bark, but in other cases they may be deeper in the wood. Broken branches hanging from live trees or old, declining trees exhibiting branch dieback seem to be especially attractive to wood-boring beetles, while dead branches laying on the ground underneath a tree are not always productive (unless they have been recently cut).

One way to target specific beetles species is to selectively cut targeted plant species during late winter, allow the cut branches to remain in situ for a full season, and then retrieve them the following winter or early spring. These almost always produce well. Doing this will also give you a chance to learn how to recognize young, infested wood at a time that is perfect for retrieval, which you can then use in searching for wood from other tree species in the area that you may not have had a chance to cut. I have cut and collected branches ranging from small twigs only ¼” diameter to tree trunks 16″ in diameter. Different species prefer different sizes and parts of the plant, but in general I’ve had the best luck with branches measuring 1–3″ diameter.

Once you retrieve the wood, you will need to cut it into lengths that fit into the container of your choice (a small chain saw makes this much easier and quicker). In the field I bundle the wood with twine and use pink flagging tape to record the locality/date identification code using a permanent marker. I then stack the bundles in my vehicle for transport back home. Choice of container is important, because moisture management is the biggest obstacle to rearing from dead wood—too much moisture results in mold, while too little can lead to desiccation. Both conditions can result in mortality of the larvae or unemerged adults. In my rearing setup, I use fiber drums ranging from 10-G to 50-G in size (I accumulated them from the dumpster where I work—mostly fiber drums used as shipping containers for bulk powders). Fiber drums are ideal because they not only breath moisture but are sturdy and may be conveniently stacked. Cardboard boxes also work as long as they are sturdy enough and care is taken to seal over cracks with duct tape. Avoid using plastic containers such as 5-G pickle buckets unless you are willing to cut ventilation holes and hot-glue fine mesh over them. While breathable containers usually mitigate problems with too much moisture, desiccation can still be a problem. To manage this, remove wood from containers sometime later in the summer (after most emergence has subsided), lay it out on a flat surface such as a driveway, and hose it down real good. Once the wood has dried sufficiently it can be placed back in the container; however, make sure the wood is completely dry or this will result in a flush of mold. I generally also wet down wood again in late winter or early spring, since I tend to hold wood batches through two full seasons.

I like to check containers every 7–15 days during spring and summer. Some people cut a hole in the side of the container that leads into a clear jar or vial—the idea being that daylight will attract newly emerged adults and facilitate their collection. I’ve tried this and was disappointed in the results—some of the beetles ended up in the vial, but many also never found their way to the vial and ended up dying in the container, only to be found later when I eventually opened it up. This is especially true for cerambycids, many of which are nocturnal and thus probably not attracted to daylight to begin with. My preference is to open up the container each time so that I can check the condition of the wood and look for evidence of larval activity (freshly ejected frass on the branches and floor of the container). I like to give the container a ‘rap’ on the floor to dislodge adults from the branches on which they are sitting, then dump the container contents onto an elevated surface where I can search over the branches and through the debris carefully so as not to miss any small or dead specimens. I use racks of 4-dram vials with tissue packed inside each and a paper label stuck on top of its polypropylene-lined cap as miniature killing jars. Specimens from a single container are placed in a vial with a few drops of ethyl acetate, and I write the container number and emergence date range on the cap label. Specimens will keep in this manner until they are ready to be mounted weeks or months (or even years) later. If the vial dries out, a few drops of ethyl acetate and a few drops of water followed by sitting overnight is usually enough to relax the specimens fully (the water relaxes the specimens, and the ethyl acetate prevents mold if they need to sit for a while longer).

I store my containers in an unheated garage that is exposed to average outdoor temperatures but probably does not experience the extreme high and low temperatures that are experienced outdoors. In the past I wondered if I needed more heat for wood collected in the desert southwest, but I never came up with a method of exposing the containers to the sun without also having to protect them from the rain. Metal or plastic containers might have eliminated this problem, but then breathability would again become an issue. I would also be concerned about having direct sun shining on the containers and causing excessive heat buildup inside the bucket that could kill the beetles within them. Now, however, considering the success that I’ve had in rearing beetles from wood collected across the desert southwest—from Brownsville, Texas to Jacumba, California, this seems not to be a big issue.

If anybody else has tips for rearing wood-boring beetles that they can offer, I would love to hear from you.

REFERENCES:

Bellamy, C. L. 2002. The Mastogenius Solier, 1849 of North America (Coleoptera: Buprestidae: Polycestinae: Haplostethini). Zootaxa 110:1–12 [abstract].

Lingafelter, S. W. 2007. Illustrated Key to the Longhorned Woodboring Beetles of the Eastern United States. Special Publication No. 3. The Coleopterists Society, North Potomac, Maryland, 206 pp. [description].

MacRae, T. C. 2003. Agrilus (s. str.) betulanigrae MacRae (Coleoptera: Buprestidae: Agrilini), a new species from North America, with comments on subgeneric placement and a key to the otiosus species-group in North America. Zootaxa 380:1–9 [pdf].

Nelson, G. H., G. C. Walters, Jr., R. D. Haines, & C. L. Bellamy.  2008.  A Catalogue and Bibliography of the Buprestoidea of American North of Mexico.  Special Publication No. 4. The Coleopterists Society, North Potomac, Maryland, 274 pp. [description].

Copyright © Ted C. MacRae 2014

The sublimely beautiful Crossidius coralinus caeruleipennis

Crossidius coralinus caeruleipennis | Inyo Co. nr. Bishop, California

Crossidius coralinus caeruleipennis | Owens Valley nr. Bishop, California

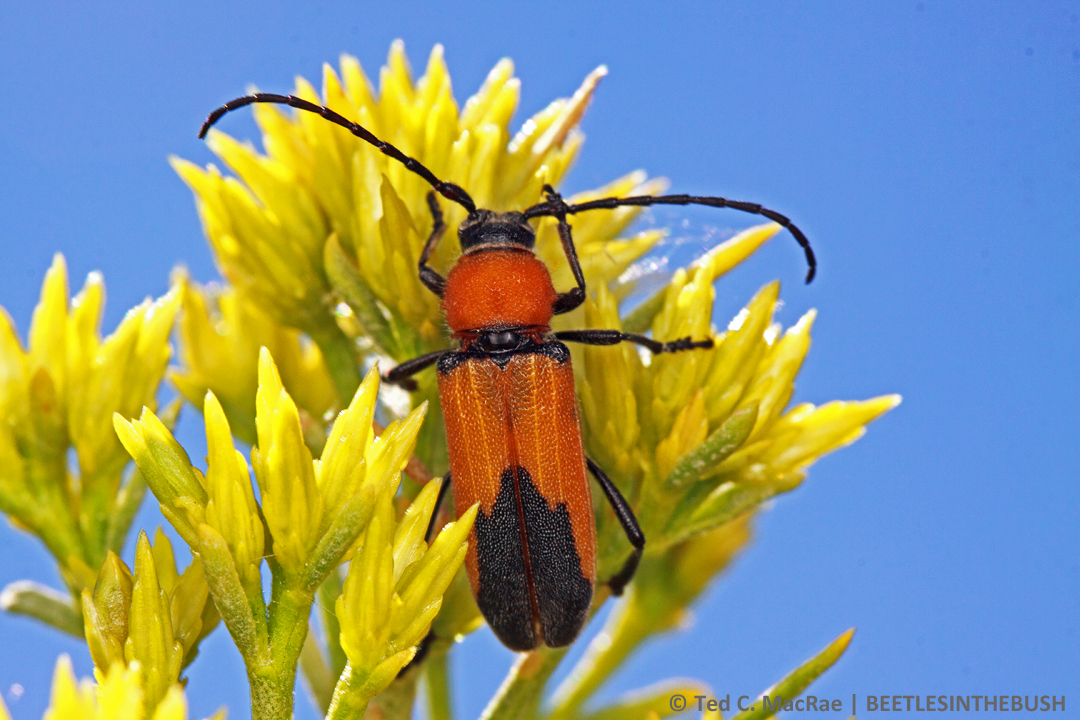
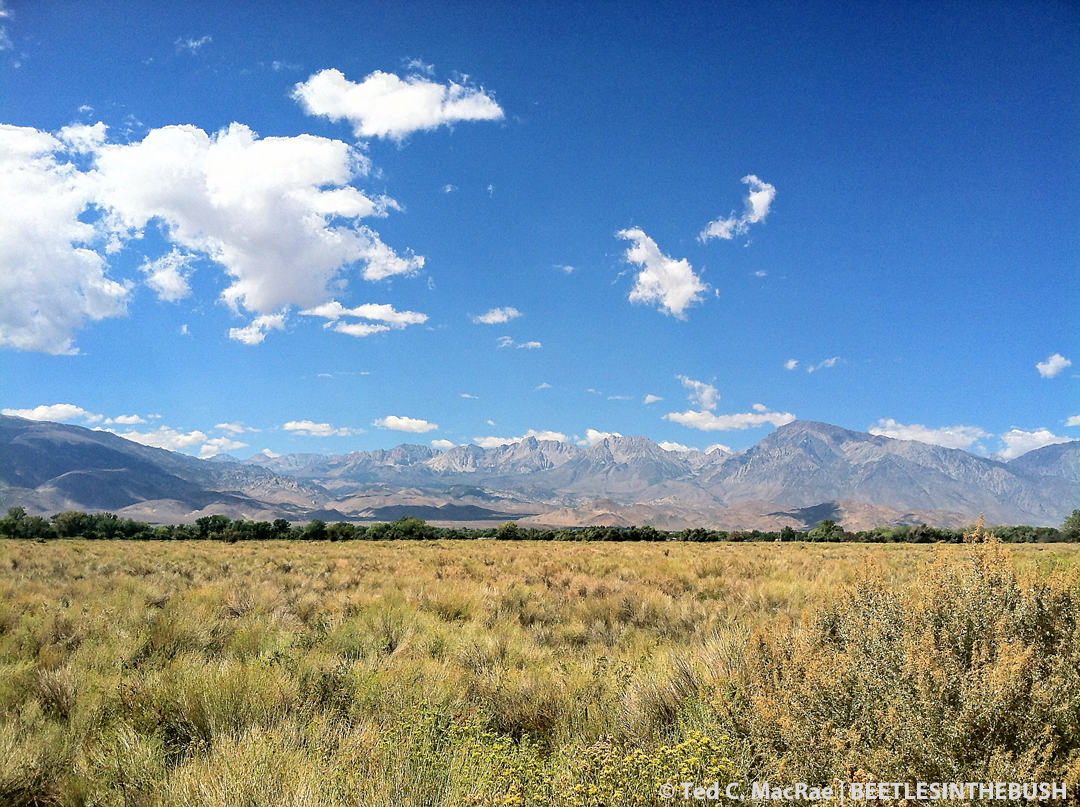
Before driving up into the White Mountains to look for Crossidius hirtipes nubilus and see the grotesquely beautiful trees at Ancient Bristlecone Pine Forest, we made a short two-mile drive north of our hotel in Bishop, California to try our hand with a C. coralinus subspecies that I referred tangentially in my previous post—C. c. caeruleipennis. This has to be among the most beautiful subspecies that I’ve seen yet of what must be considered one of North America’s most attractive species of longhorned beetle. In contrast to the other “orange” subspecies, C. c. monoensis, which we had collected the previous day but that I did not even recognize as C. coralinus because of its color and very small size, I knew exactly what I was looking for on this day as we began to scan the gray rabbitbrush (Ericameria nauseosa) plants that stretched out across the Owens Valley sage grassland as far as the eye could see. At first we were worried that we might be a little late, as most of the plants appeared to be somewhat past peak bloom, but it wasn’t long before we found the first individual sitting atop a flower cluster, and then another, and another...

Males are completely orange.

Males are solid, sublimely orange with strikingly contrasting black legs and antennae.

Crossidius c. caeruleipennis is immediately distinguishable from C. c. temprans (and most of the other C. coralinus ssp. that we collected on the trip further north in Nevada and east in Utah and Colorado) by its bright orange rather than dark red coloration. The subspecies is restricted to the Owens Valley of eastern California and greatly resembles another of the orange subspecies that we collected on the trip, C. c. monoensis. That subspecies is found just a short distance north in the Mono Basin, though at much higher elevations, and is easily distinguished from C. c. caeruleipennis by its smaller average size, by having the black markings of the elytra more expanded apically in females and at least present in males, and by the presence of black bands along the apical and basal margins of the pronotum (Linsley & Chemsak 1961).

Females have a distinct apical blue-black marking on the elytra

Females are distinguished by the apical blue-black marking on the elytra and their shorter antennae.

As it turned out, the beetle was as abundant as any we had seen on the trip to that point. Not that it didn’t require some effort to collect them—they were still rather sparsely distributed among the plants and definitely showed preference for plants that were not as far past peak bloom. However, the habitat was extensive—we could have wandered freely for hours on end without looking at the same plant twice (although that did not stop me from re-checking a few plants that were in peak bloom and seemed to be especially favored). The males were simply gorgeous—a bright, creamy orange that sadly takes on a dull quality in preserved specimens and with long black legs and antennae. The females are no dogs either, less strikingly orange due to the blue-black apical markings on the elytra, but certainly more robust than the males in a subspecies that is already one of the larger of the species. Temperatures climbed rapidly at this relatively southern and lower elevation locality compared to most of the others that we visited during the trip, so the beetles became quite active very quickly after we began to see them. I had only a short window of time in which to attempt field photographs, and while I’m not completely satisfied with the ones that I show here, they were the best that I could manage and still get the blue sky background that I desire for “beetles on flowers” photographs.

Sage grassland and gray rabbitbrush dominate the Owens Valley where C. coralinus caeruleipennis is found.

Gray rabbitbrush dominates the Owens Valley sage grassland where C. coralinus caeruleipennis occurs.

REFERENCE:

Linsley, E. G. & J. A. Chemsak. 1961. A distributional and taxonomic study of the genus Crossidius (Coleoptera, Cerambycidae). Miscellaneous Publications of the Entomological Society of America 3(2):25–64 + 3 color plates.

Copyright © Ted C. MacRae 2014
Clouded beetles amidst spectacular scenery

“Westerly from Westgard Pass is a view equaled in few parts of America. In the middle distance, a dozen miles away and nearly a mile below, lies the fertile Owens Valley, extending at right angles north and south over a hundred miles, and on the farther side, distant a score of miles, tower the snow-clad Sierras, with serrated crests and symmetric domes and peaks outlined against the sky at an approximate height of two and one-half miles vertical above the level of the ocean, and extending north and south far as the eye can see. The vision is rich reward for a journey of a thousand leagues.”—A. L. Westgard, March 1915

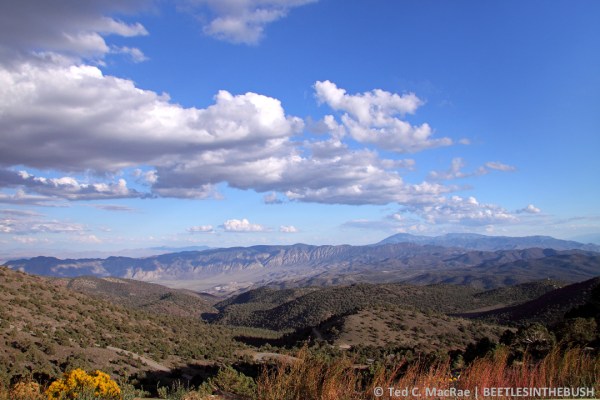
View of Westgard Pass from higher up in the White Mountains near Ancient Bristlecone Pine Forest.

View to Westgard Pass from higher up in the White Mountains near Ancient Bristlecone Pine Forest.

After a morning spent searching for Crossidius coralinus caeruleipennis (perhaps the most sublimely beautiful of the subspecies) in the high desert sage of the wide open Owens Valley floor near Bishop, California, we made the short drive south to Big Pine, turned sharply left, and began the slow, twisting ascent through a narrow gap between the White Mountains to the north and the Inyo Mountains to the south. Eventually reaching an elevation of 7,313 ft,  Westgard Pass serves as access to Earth’s oldest living things! and, in doing so, provides some of the most striking scenery in the entire Basin and Range Province of eastern California.

Westgard Pass, Inyo Co., California.

Chrysothamnus viscidiflorus (small plants with yellow flowers) host Crossidius hirtipes nubilus adults.

Field mate Jeff Huether and I no doubt wanted to see the grotesquely beautiful trees growing in Ancient Bristlecone Pine Forest and were happy to enjoy the magnificent scenery along the way, but our trek to Westgard Pass had also a strictly entomological purpose—to search for Crossidius hirtipes nubilus, among the most uniquely colored and geographically restricted of the C. hirtipes subspecies. Approaching the summit, the narrow, rocky gorge opened up to a broad expanse of pinyon/juniper woodland, and nestled among the ubiquitous sage we found the plant we were looking for—yellow rabbitbrush (Chrysothamnus viscidiflorus) in full bloom.

Crossidius hirtipes nubilus (male) on flowers of Chrysothamnus viscidiflorus.

Crossidius hirtipes nubilus (male) on flowers of Chrysothamnus viscidiflorus (field photo).

It took a while, however, before we found the beetles that we were looking for. Robust gray rabbitbrush (Ericameria nauseosa) plants in full bloom conspicuously dominated the roadsides and demanded our initial attentions, but our only reward was the widespread Crossidius ater. Not even a single Crossidius coralinus specimen could be claimed as consolation. Still, we knew the real quarry was further back from the roadsides, on the much smaller and less conspicuous yellow rabbitbrush that serves as an adult host for Crossidius hirtipes and most of its subspecies. Once we turned our attentions to these smaller plants we found the first adult fairly quickly, but precious few were seen considering the many plants that we examined until we finally zeroed in on one area just south of the summit where the beetles seemed to occur with slightly greater frequency. While not numerous, we eventually found enough beetles for us to declare, “Let’s go see the bristlecone pines!”

In addition to their longer antennae, males are distinguished by xxx.

In addition to longer antennae, males are distinguished by less extensive clouding (studio photo).

This subspecies is among the most distinctive of all the C. hirtipes subspecies due to the combination of dark reddish-brown coloration and extreme, dark clouded area of the elytra (Linsley & Chemsak 1961). It most closely resembles C. h. rhodopus, which occurs further north in the Mono Basin, but that subspecies is not as dark and lacks the extensive clouding of black on the apical portions of the elytra.

Females have the elytral markings xxx.

Females have the markings greatly expanded to almost completely cover the elytra (studio photo).

The dark clouding actually represents an expansion of the dark stripe found along the suture of the elytra of many C. hirtipes subspecies, most of which exhibit sexual dimorphism in the degree to which this stripe is developed. In some subspecies the stripe is present in the females but absent in the males, while in others the stripe is present in both but more fully developed in the female. In C. h. nubilus the sutural stripe reaches an extreme state of development, covering much of the apical two-thirds of the elytra in the male and being so greatly expanded in females that almost the entire elytra are covered except for two small subbasal patches revealing the ground color of the elytra.

REFERENCES:

Linsley, E. G. & J. A. Chemsak. 1961. A distributional and taxonomic study of the genus Crossidius (Coleoptera, Cerambycidae). Miscellaneous Publications of the Entomological Society of America 3(2):25–64 + 3 color plates.

Copyright © Ted C. MacRae 2014
Best of BitB 2013

Welcome to the 6th Annual “Best of BitB”, where I pick my favorite photographs from the past year. Like last year, 2013 was another year of heavy travel. For work I did my annual tour of soybean field sites throughout Argentina during late February and early March, then cranked it up for my own field season with frequent travel to sites in Illinois and Tennessee from May to October. In the meantime I spent a week at company meetings in Las Vegas in August, toured field sites across the southeastern U.S. for two weeks in September, visited Argentina again in October to finalize research plans for their upcoming season, and finished off the travel year by attending the Entomological Society of America (ESA) Meetings in Austin, Texas during November. On top of all this, I managed to slip in two of the best insect collecting trips I’ve had in years, with 10 days in northwestern Oklahoma in early June and another 10 days in California, Nevada, Utah, and Colorado during late August, and I got to play “visiting scientist” during short trips to Montana State University in late July and the Illinois Natural History Survey in late October! Of course, during my brief interludes at home I wasn’t sitting still, giving entomology seminars to several local nature societies and hosting two ESA webinars on insect photography. Needless to say, come December I was more than ready to spend some quite time at home (well, except for hiking most weekends) and am happy to report that I’ve successfully become reacquainted with my family and office mates. It’s a peripatetic life—and I wouldn’t have it any other way!

Okay, let’s get down to business. Here are my favorite BitB photographs from 2013. This year was less about learning new techniques as it was about refining the techniques I’ve found most useful for the style I’ve chosen as a photographer, i.e., hand-held, in situ field shots that (hopefully) excel at both natural history and aesthetic beauty. Links to original posts are provided for each photo selection, and I welcome any comments you may have regarding which (if any) is your favorite and why—such feedback will be helpful for me as I continue to hone my craft. If you’re interested, here are my previous years’ picks for 2008, 2009, 2010, 2011, and 2012. Once again, thank you for your readership, and I hope to see you in 2014!


Tremex columba, female ovipositing | Sam A. Baker State Park, Missouri

Tremex columba female drilling for oviposition into hardwood trunk | Sam A. Baker State Park, Missouri

From Ovipositing Pigeon Horntail (posted 6 Jan). I like this photo for the combination of vibrant, contrasting colors between the wasp and moss-covered wood and the visualization it provides of the remarkable depth to which this wasp will insert its ovipositor into solid wood!


Eurhinus cf. adonis on Solidago chilensis | Chaco Province, Argentina

Eurhinus cf. adonis on Solidago chilensis flowers | Chaco Province, Argentina

From Giving me the weevil eye! (posted 28 Apr). While a little soft, the color combination is pleasing and the pose taken by the beetle almost comically inquisitive.


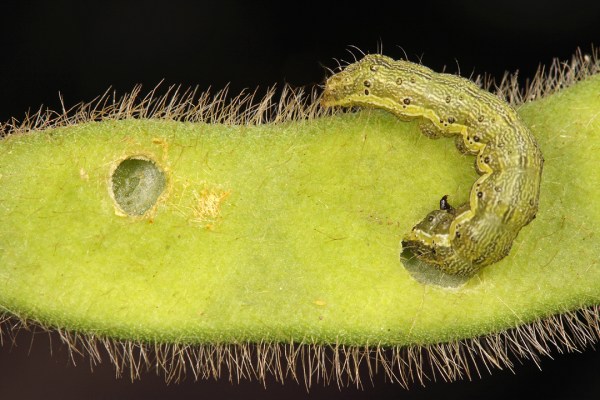
Helicoverpa gelotopeon feeding on soybean pod | Buenos Aires Prov., Argentina

Helicoverpa gelotopeon feeding on soybean pod | Buenos Aires Prov., Argentina

From Bollworms rising! (posted 30 Mar). This is the first photo of an economic pest that has made one of my “Best of BitB” lists. The two holes in the soybean pod, one with the caterpillar and its head still completely inserted, visualizes how the feeding habits of these insects can so dramatically affect yield of the crop.


cf. Eremochrysa punctinervis | Gloss Mountains, Major Co., Oklahoma

cf. Eremochrysa punctinervis | Gloss Mountains, Major Co., Oklahoma

From “Blue-sky” tips and tricks (posted 1 July). Insects with a lot of delicate detail and long, thin appendages are especially difficult to photograph against the sky due to wind movement. See how I dealt with the antennae of this delicate lacewing without resorting to the standard black background typical of full-flash macrophotography.


Cicindela scutellaris lecontei x s. unicolor

Cicindela scutellaris lecontei x s. unicolor intergrade | Holly Ridge Natural Area, Stoddard Co., Missouri

From The Festive Tiger Beetle in Southeast Missouri (posted 25 Oct). I like this photo a lot more now than I did when I first took it. Its shadowy feel and the beetle “peering” from behind a leaf edge give a sense of this beetle’s attempts to hide and then checking to see if the “coast is clear”


Batyle suturalis on paperflower (Psilostrophe villosa) | Alabaster Caverns State Park, Woodward Co., Oklahoma

Batyle suturalis on Psilostrophe villosa flowers | Alabaster Caverns State Park, Woodward Co., Oklahoma

From Tips for photographing shiny beetles on yellow flowers (posted 10 Aug). “Bug on a flower” photos are a dime a dozen, but shiny beetles on yellow flowers with natural sky background can be quite difficult to take. All of the techniques for dealing with the problems posed by such a photo came together nicely in this photo.


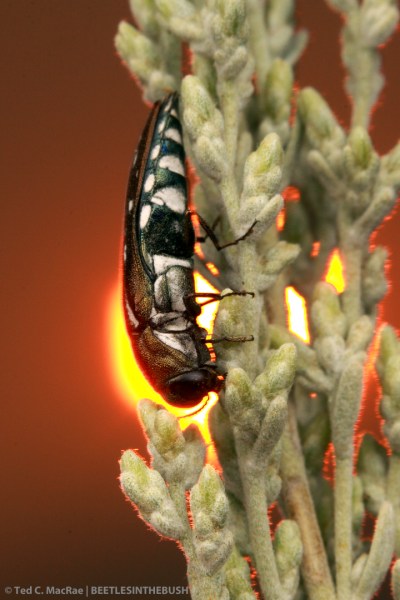
Agrilus walsinghami | Davis Creek Regional Park, Washoe Co., Nevada

Agrilus walsinghami | Davis Creek Regional Park, Washoe Co., Nevada

From Sunset for another great collecting trip (posted 1 Sep). This photo is not without its problems, with a little blurring of the backlit fuzz on the plant, but the placement of the sun behind the subject’s head and resulting color combination make it my favorite in my first attempts at achieving a “sun-in-the-sky” background with a true insect macrophotograph.


A tiny male mates with the ginormous female.

Pyrota bilineata on Chrysothamnus viscidflorus | San Juan Co., Utah

From Midget male meloid mates with mega mama (posted 8 Nov). Another blue-sky-background photograph with good color contrast, its real selling point is the natural history depicted. with some of the most extreme size dimorphism among mating insects that I’ve ever seen.


Phymata sp.

Phymata sp. on Croton eleagnifolium foliage | Austin, Texas

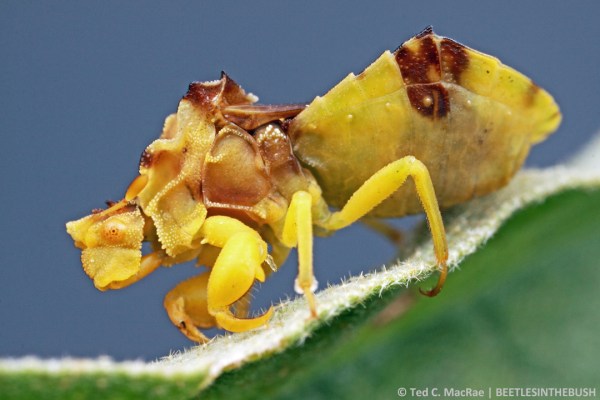
From ESA Insect Macrophotography Workshop (posted 13 Nov). The oddly sculpted and chiseled body parts of ambush bugs makes them look like they were assembled from robots. Contrasting the body against a blue sky gives a more unconventional view of these odd beasts than the typical top-down-while-sitting-on-a-flower view.


Fourth attempt - holding detached pad up against sky for cleaner background.

Moneilema armata on Opuntia macrorhiza | Alabaster Caverns State Park, Woodward Co., Oklahoma

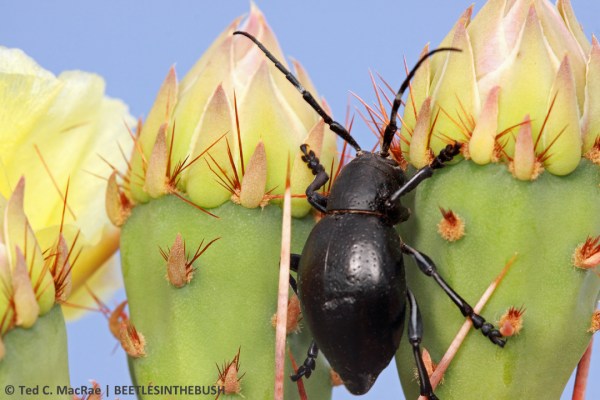
From Q: How do you photograph cactus beetles? (posted 24 Nov). Photographing cactus beetles requires patience, persistence, long forceps, and strong forearms. Natural sky provides a much more pleasing background than a clutter of cactus pads and jutting spines.


I hope you’ve enjoyed this 2013 version of “Best of BitB” and look forward to seeing everyone in 2014.

Copyright © Ted C. MacRae 2013

Hairy milkweed beetle

Across the Great Plains of North America, sand dune fields dot the landscape along rivers flowing east out of the Rocky Mountains. Formed by repeated periods of drought and the action of prevailing south/southwest winds on alluvium exposed by uplifting over the past several million years, many of these dunes boast unique assemblages of plants and animals adapted to their harsh, xeric conditions. Some are no longer active, while others remain active to this day. Among the latter is Beaver Dunes in the panhandle of northwestern Oklahoma.

Beaver Dunes, Oklahoma

Beaver Dunes State Park, Beaver Co., Oklahoma

As I explored the more vegetated areas around the perimeter of the dunes, I spotted the characteristically hairy, fleshy, opposite leaves of Ascelpias arenaria. Known also as “sand milkweed,” this plant is associated with sand dunes and other dry sandy soil sites throughout the central and southern Great Plains. I always give milkweeds a second look whenever I encounter them due to the association with them by longhorned beetles in the genus Tetraopes. It wasn’t long before I spotted the black antennae and red head of one of these beetles peering over one of the upper leaves from the other side.

Tetraopes pilosus on Asclepias arenaria

Tetraopes pilosus on Asclepias arenaria | Beaver Dunes State Park, Oklahoma

This was no ordinary Tetraopes, however. Its large size, dense covering of white pubescence, and association with sand milkweed told me immediately that this must be T. pilosus (the specific epithet meaning “hairy”). Like its host, this particular milkweed beetle is restricted to Quaternary sandhills in the central and southern Great Plains (Chemsak 1963), and also like its host the dense clothing of white pubescence is presumably an adaptation to prevent moisture loss and overheating in their xeric dune habitats (Farrell & Mitter 1998).

Tetraopes pilosus

Species of Tetraopes have the eyes completely divided by the antennal insertions—thus, “four eyes.”

Tetraopes is a highly specialized lineage distributed from Guatemala to Canada that feed as both larvae and adults exclusively on milkweed (Chemsak 1963). Larval feeding occurs in and around the roots of living plants, a habit exhibited by only a few other genera of Cerambycidae but unique in the subfamily Lamiinae (Linsley 1961). Milkweed plants are protected from most vertebrate and invertebrate herbivores by paralytic toxins, commonly termed cardiac glycosides or cardenolides. However, a few insects, Tetraopes being the most common and diverse, have not only evolved cardenolide insensitivity but also the ability to sequester these toxins for their own defense. Virtually all insects that feed on milkweed and their relatives have evolved aposematic coloration to advertise their unpalatability, and the bright red and black color schemes exhibited by milkweed beetles are no exception.

Species of the genus Tetraopes are characterized by the completely divided eyes.

Adult beetles, like the leaves of their hosts, are clothed in white pubescence.

As  noted by Mittler & Farrel (1998), variation in coloration among the different species of Tetraopes may be correlated with host chemistry. Milkweed species vary in toxicity, with more basal species expressing simpler cardenolides of lower toxicity and derived species possessing more complex and toxic analogs. Most species of Tetraopes are associated with a single species of milkweed, and it has been noted that adults of those affiliated with less toxic milkweeds on average are smaller, have less of their body surface brightly colored, and are quicker to take flight (Chemsak 1963, Farrell & Mitter 1998). Thus, there seems to be a direct correlation between the amount of protection afforded by their host plant and the degree to which the adults advertise their unpalatability and exhibit escape behaviors. Asclepias arenaria and related species are the most derived in the genus and contain the highest concentrations of cardenolides. In fact, they seem to be fed upon only by Tetraopes and monarchs while being generally free from other more oligophagous insect herbivores such as ctenuchine arctiid moths and chrysomelid beetles that feed on less derived species of milkweed (Farrell & Mitter 1998). Accordingly, T. pilosus is among the largest species in the genus and has the majority of its body surface red. Also, consistent with it being more highly protected than others in the genus, I noted virtually no attempted escape behavior as I photographed this lone adult.

Asclepias arenaria

Asclepias arenaria (sand milkweed) growing at the base of a dune.

In addition to metabolic insensitivity to cardenolides, adult Tetraopes also exhibit behavioral adaptations to avoid milkweed defenses (Doussard & Eisner 1987). The milky sap of milkweed is thick with latex that quickly dries to a sticky glue that can incapacitate the mouthparts of chewing insects that feed upon the sap-filled tissues. Adult Tetraopes, however, use their mandibles to cut through the leaf midrib about a quarter of the way back from the tip. This allows much of the sticky latex-filled sap to drain from the more distal tissues, on which the beetle then begins feeding at the tip. Leaves with chewed tips and cut midribs are telltale signs of feeding by adult Tetraopes.

REFERENCES:

Chemsak, J. A. 1963. Taxonomy and bionomics of the genus Tetraopes (Coleoptera: Cerambycidae). University of California Publications in Entomology 30(1):1–90, 9 plates.

Doussard, D. E. & T. Eisner. 1987. Vein-cutting behavior: insect counterploy to the latex defense of plants. Science 237:898–901 [abstract].

Farrell, B. D. & C. Mitter. 1998. The timing of insect/plant diversification: might Tetraopes (Coleoptera: Cerambycidae) and Asclepias (Asclepiadaceae) have co-evolved? Biological Journal of the Linnean Society 63: 553–577 [pdf].

Linsley, E.G. 1961. The Cerambycidae of North America. Part 1. Introduction. University of California Publications in Entomology 18:1–97, 35 plates.

Copyright © Ted C. MacRae 2013

A winter longhorned beetle

According to the calendar it’s still autumn; however, in practical terms winter has settled in across much of the U.S. For those of us who study wood-boring beetles in the families Buprestidae (jewel beetles) and Cerambycidae (longhorned beetles), our time for collecting ended long ago. Adults of most species are active in spring and early summer, although some species don’t really make their appearance until summer is in full swing and a few rather distinctive species in genera such as Crossidius and Megacyllene make their appearance exclusively during fall. There is one longhorned beetle, however, that can actually be encountered in its greatest numbers during the dead of winter—Rhagium inquisitor, or the “ribbed pine borer.”

Rhagium inquisitor | Reynolds Co., Missouri

Rhagium inquisitor overwintering adult | Reynolds Co., Missouri

Rhagium inquisitor is unique among North American cerambycids in several respects. Most species in the family overwinter as mature or immature larvae, the former triggered to pupation by the first warm days of late winter and early spring in preparation for emergence as adults a few weeks later. Rhagium inquisitor, on the other hand, pupates during late summer and fall and then transforms to the adult before winter sets in (Linsley & Chemsak 1972), passing the winter in this stage and emerging during the earliest days of spring. Also unique among North American cerambycids is the place of pupation—directly under the bark. This contrasts with most other species, which either feed and pupate within the sapwood or feed under the bark but then bore into the sapwood for pupation. The species breeds exclusively in the trunks of dead conifers, with pines (Pinus spp.) especially favored, and as a result one can easily encounter the adults by peeling back the bark of dead pines during winter. Pupation takes place within distinctive rings of frass and coarse, fibrous wood shavings, prepared by the larva prior to pupation, so even when adults and larvae are not present the occurrence of this species can be determined by the occurrence of their pupation rings.

Adults overwinter in cells lined with frass and fibrous wood shavings.

Adults overwinter in cells lined with frass and fibrous wood shavings.

Not only are the overwintering and pupation habits of this species unique, but the adults themselves are distinctive from all other North American cerambycids (Yanega 1996) in their appearance—”big-shouldered” build, heavily “ribbed” elytra, and unusually short antennae (that are anything but “longhorned”). Lastly, the species is distributed not only in the boreal forests of North America, but Europe and Asia as well. The species is extremely variable in size and sculpturing, which combined with its Holarctic distribution has led to an unusually high number of synonyms. In fact, much of the North American literature prior to Linsley & Chemsak (1972) concluding that the North American and Eurasian forms represented the same species refers to this species as R. lineatum.

REFERENCES:

Linsely, E. G. & J. A. Chemsak. 1972. Cerambycidae of North America, Part VI, No. 1. Taxonomy and classification of the subfamily Lepturinae. University of California Publications in Entomology 69:viii + 1–138, 2 plates.

Yanega, D. 1996. Field Guide to Northeastern Longhorned Beetles (Coleoptera: Cerambycidae). Illinois Natural History Survey Manual 6: x + 1–174 [preview].

Copyright © Ted C. MacRae 2013