3rd Blogoversary, 7 New Blogs, & AIF #10

Today happens to be BitB’s 3rd blogoversary.  I won’t bore you with an attempt at witty, insightful introspection on what it means to have reached this modest milestone.  BitB is still what it started out as – tales from my life-long, entomocentric, natural history learning experience.  I’ve enjoyed these past three years immensely, learned far more than I would have initially imagined, and deeply appreciate the support and encouragement I’ve received from an admireably erudite readership.

Rather than talk on about myself, however, I’d like to talk about others.  I’m always on the lookout for new blogs – those that seem interesting make the blogroll, and if I find their content compelling enough they make my RSS feed list.  A few rise to the top due to their superior photography, insightful writing, or close alignment with my own interests – these I like to feature from time to time by name in an occasional post such as this one.  Following is the latest crop of new sites (or at least new to me) that have piqued my interest:

Crooked Beak Workshop is written by coleopterist Delbert la Rue, Research Associate at the Entomology Research Museum, University of California, Riverside.  I can forgive his primary interest in Pleocomidae (rain beetles) and other scarabaeoid taxa due to his strong side interests in Cicindelidae (tiger beetles), Buprestidae (jewel beetles), and ecology of sand dune ecosystems.  Posts occur irregularly, but when they do appear they are good old-fashioned hardcore coleopteran taxonomy and desert southwest ecology – what could be better?

Field Notes is a herpetology website by Bryan D. Hughes.  “Spectacular” does not even begin to describe his photographs, focused heavily on the marvelous diversity of venomous snakes and other reptiles in the desert southwest (and the occasional desert arachnid as well).  Bryan hopes his pictures and information will help homeowners who choose to live in areas harboring native wildlife become interested in it rather than kill it due to fear and myth – I hope he succeeds!

Gardening with Binoculars is a fairly new site by my good friend and fellow WGNSS member Anne McCormack.  Anne is a true “naturalist’s naturalist,” with solid knowledge that spans the breadth of Missouri’s flora and fauna – both vertebrate and invertebrate.  In GWB, Anne uses this knowledge and her considerable writing talents to weave informative and entertaining tales of her experiences with wildlife in a small native plant garden.  I can almost hear the campfire crackling in the background!

Natural History Museum Beetle blog is a new blog by Beulah Garner, one of the curators of Coleoptera in the Entomology department at The Natural History Museum in London (I am sooo jealous!).  With only two posts under her belt so far, it might be premature to give the site such quick praise; however, I couldn’t resist – the 2nd post had photos of tiger beetles!  Regardless, working amongst more than 9 million insects (did I mention I’m jealous?) should provide plenty of fodder for future posts.
The Atavism is written by David Winter, a PhD student in evolutionary genetics in New Zealand.  Wide ranging in his interests, it is his  series that has captured my interest (and while “spineless” across much of the blogosphere means squishy marine animals, David’s spinelessness is more to my liking – i.e., arthropod-heavy).  Moreover, in true academic fashion, David usually finds an unusual angle from which to discuss his subjects.

The Prairie Ecologist. Chris Helzer is an ecologist for The Nature Conservancy in Nebraska whose writings demonstrate deep, intimate understanding of the prairie landscape and its myriad biotic interactions, as well as the passion that many of us here in the heartland feel when looking out on its vast expanses.  As if that wasn’t enough, Chris is also one of the rare bloggers who combines his well-crafted writing with truly spectacular photography – he’s the total package!

The Sam Wells Bug Page is written by – you guessed it – Sam Wells.  This is a straight up entomology site, featuring a diversity of insects from that wonderful state called California.  You won’t find these insects anywhere else on the web, and though it is (to my liking) heavy on the beetles, a variety of other insect groups are featured as well.  What’s more, each post almost always contains fabulous photos of that remarkable California landscape.  Each post is a little mini-collecting trip – I get a little homesick for the Sierra Nevada every time I read!


One final note – Heath Blackmon at Coleopterists Corner has posted the tenth edition of An Inordinate Fondness.  This was Heath’s first blog carnival hosting gig (could there have been any more appropriate?), but you wouldn’t know it by looking – 14 coleocontributions artfully presented, each with a teaser photo and just enough text to invite further clicking.  Head on over to AIF #10 and enjoy elytral ecstasy at its finest (and don’t forget to tip the waiter!).

Copyright © Ted C. MacRae 2010

Desmocerus palliatus – elderberry borer

Desmocerus palliatus (elderberry borer), Squaw Creek Natl. Wildlife Refuge, Missouri.

Last June I made two trips to the Loess Hills in northwestern Missouri to survey additional sites for Cylindera celeripes (swift tiger beetle), which my colleague Chris Brown and I had discovered in some of the area’s few remaining loess hilltop prairie remnants the previous year. One of these potential new sites was  Squaw Creek National Wildlife Refuge, where a few tiny slivers of hilltop prairie can still be found on the fingers of loess bluffs that border the refuge’s several thousand acres of restored wetlands that famously host large concentrations of snow geese and bald eagles during the fall and spring migrations.  On the first visit, I had arranged to meet with Corey Kudrna, Refuge Operations Specialist, who was kind enough to take several hours out of his day to personally guide me to each of the site’s loess hilltop prairie remnants. 

As we crossed the highway right-of-way at the base of the bluffs on our way to the one of the remnants, we passed through a large patch of common elderberry, Sambucus nigra ssp. canadensis.  Anytime I see patches of this plant, especially in June, I immediately think of Desmocerus palliatus (elderberry borer) – a spectacularly colored longhorned beetle (family Cerambycidae) that breeds exclusively in the living stems and roots of this plant.  It is not a particularly rare species, but for some reason I have not had much success in finding this species.  In my close to three decades of collecting beetles, I had encountered perhaps a half dozen individuals – never more than two at the same time.  Still, when I get the chance to look at elderberry I look for this beetle, and when I did so this time I was delighted to see one within a few moments of entering the patch.  I was ecstatic when I saw another one almost immediately after the first, and I was stunned when I realized that they were all around me!  Good fortune continued on my subsequent visit two weeks later, when I was able to spend a little more time trying to get a good field photograph.  Wind was a problem, the beetles were easily alarmed, and their tendency to rest in the upper reaches of the plant made it difficult to brace myself and the camera while shooting, making this a rather difficult subject to get a good photograph of.  The photo shown here is literally the last of around two dozen that I took and is the only one that I really like.

Many cerambycid beetles are mimics of other more noxious species, mostly ants and wasps.  However, elderberry borers appear to be the exception in that they are themselves noxious.  The cobalt blue and bright orange coloration of the adults screams aposematic (warning) coloration, and it is reasonable to assume that they accumulate in their bodies for defensive purposes the cyanogenic glucosides produced by elderberry plants (Huxel 2000).  Even their movements are those of a chemically protected model – lumbering and clumsy, without the alert evasiveness usually seen with other flower longhorn species.  Presumably this species participates in a Müllerian mimicry complex involving netwinged beetles (family Lycidae, particularly species in the genus Calopteron) and perhaps Pyromorpha dimidiata (orange-patched smoky moth, family Zygaenidae) as well, and it may serve as a Batesian model for the equally colorful but completely innocuous Lycomorpha pholus (black-and-yellow lichen moth, family Arctiidae).

Photo Details: Canon 50D w/ 100mm macro lens (ISO 100, 1/250 sec, f/10), Canon MT-24EX flash w/ Sto-Fen diffusers.

REFERENCE:

Huxel, G. R.  2000.  The effect of the Argentine ant on the threatened valley elderberry longhorn beetle.  Biological Invasions 2:81–85.

Copyright © Ted C. MacRae 2010

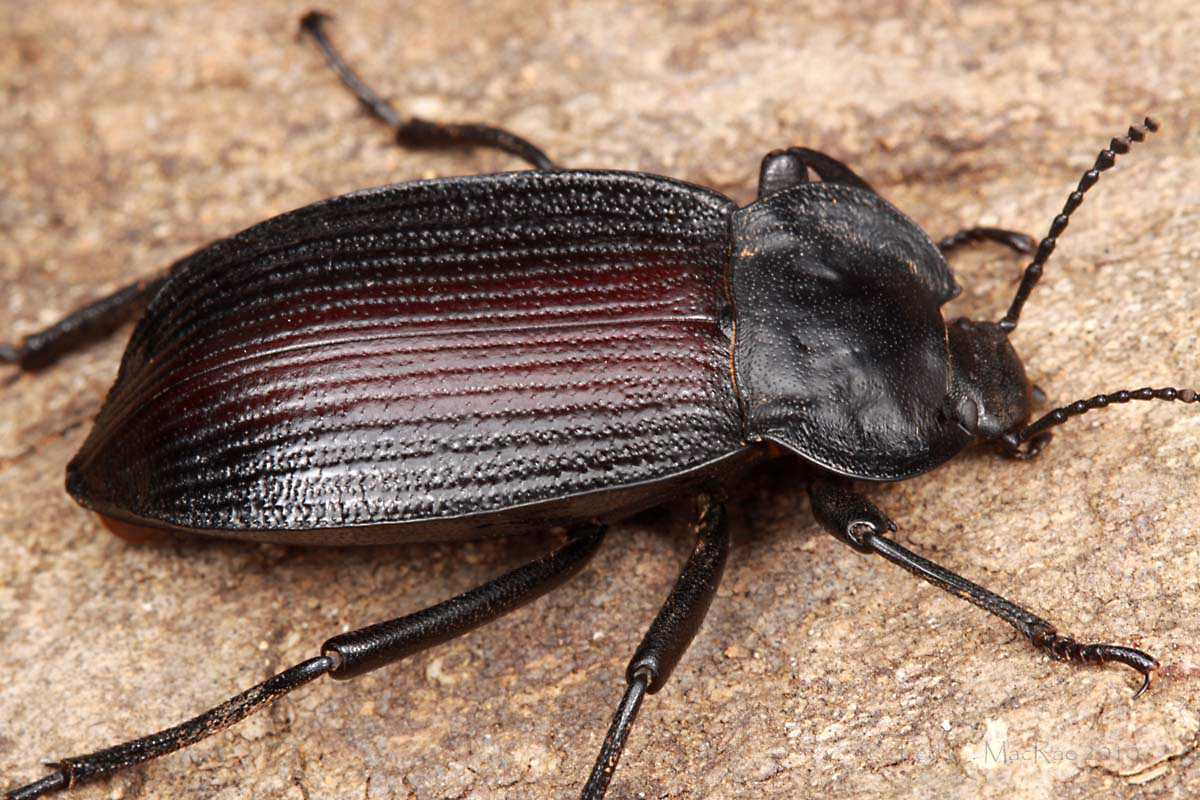
The “best” Eleodes suturalis

Eleodes suturalis - "sutured" clown beetle

Testing with my new diffuser setup¹ continues. I’ve kept this “sutured” clown beetle (Eleodes suturalis) alive since last July as a terrarium-mate with my Great Plains giant tiger beetles (Amblycheila cylindriformis). The first photos I took of it in the terrarium with the old diffusers (Sto-Fen + Puffers) can only be described as “ho-hum.” The next series (with the beetle cleaned up a bit) was taken in a white box with indirect flash and represented a nice improvement over the first shots. Here, the beetle is back in the terrarium on a piece of bark using direct flash and the new diffuser. I think it has the best of both worlds – nicely diffused lighting on a natural substrate (without the need for a white box). Yes, the focus is a bit off in the head area – the beetle was really not very cooperative during the shoot, and I was just interested in seeing how the lighting would look without spending too much time trying to capture the “perfect” shot.

¹ Photos of the diffuser and instructions on how to make it are coming, I promise! I’ve made a few improvements over the prototype by eliminating the tape to hold things together and am just working on the attachment to the MT-24EX flash bracket.

I really hope this diffuser works out for me in the field!

Photo Details: Canon 50D w/ 100mm macro lens (ISO 100, 1/250 sec, f/16), direct Canon MT-24EX flash w/ oversized concave diffuser. Typical post-processing (levels, minor cropping, unsharp mask).

Copyright © Ted C. MacRae 2010

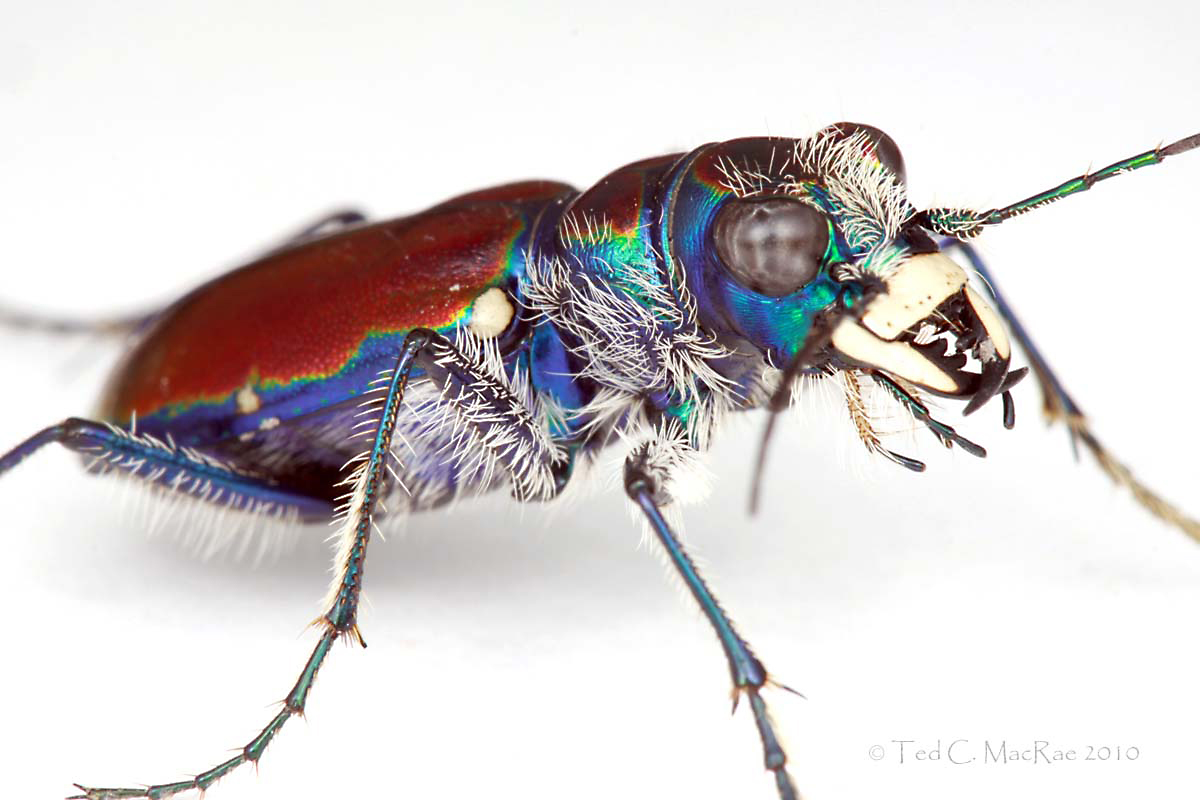
Cicindela pulchra on white

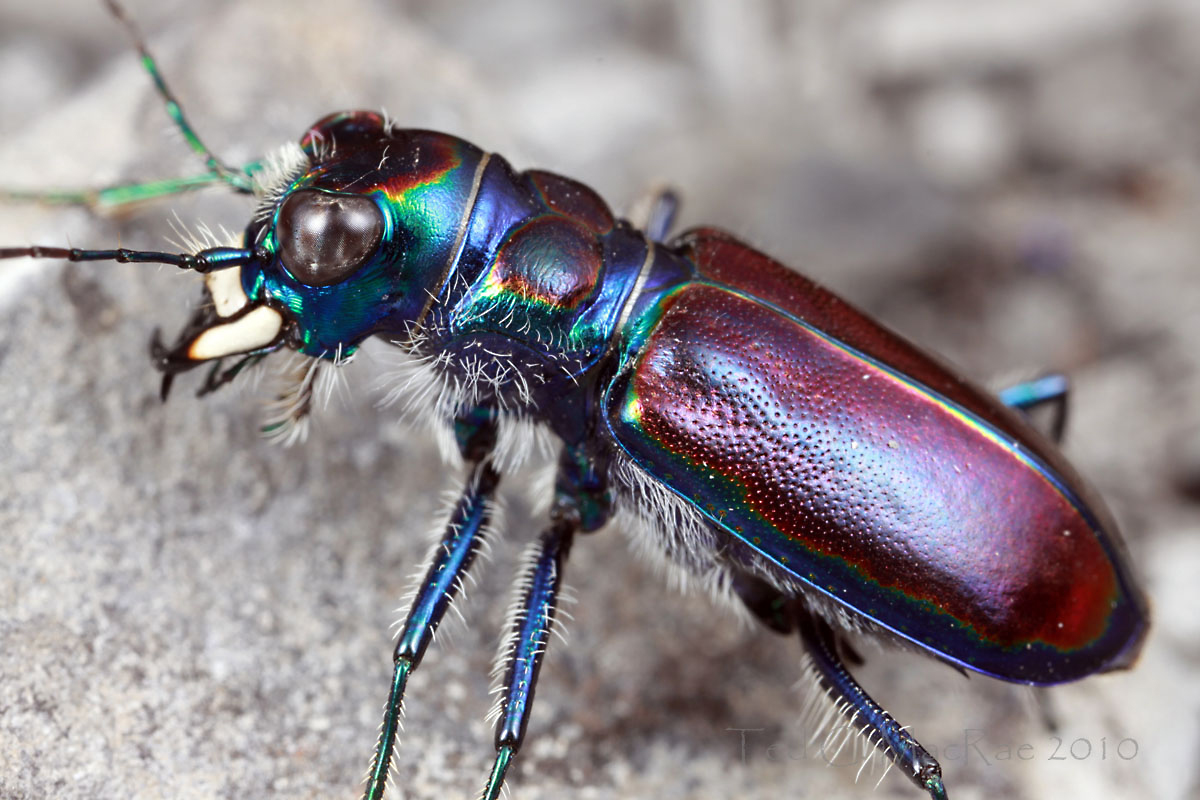
Two more photographs taken with my new diffuser, this time the spectacular Cicindela pulchra (beautiful tiger beetle). Which one do you like better?

Photo Details: Canon 50D w/ 100mm macro lens (ISO 100, 1/250 sec, f/16), Canon MT-24EX flash w/ oversized concave diffuser. Standard post-processing (levels, unsharp mask).

Copyright © Ted C. MacRae 2010

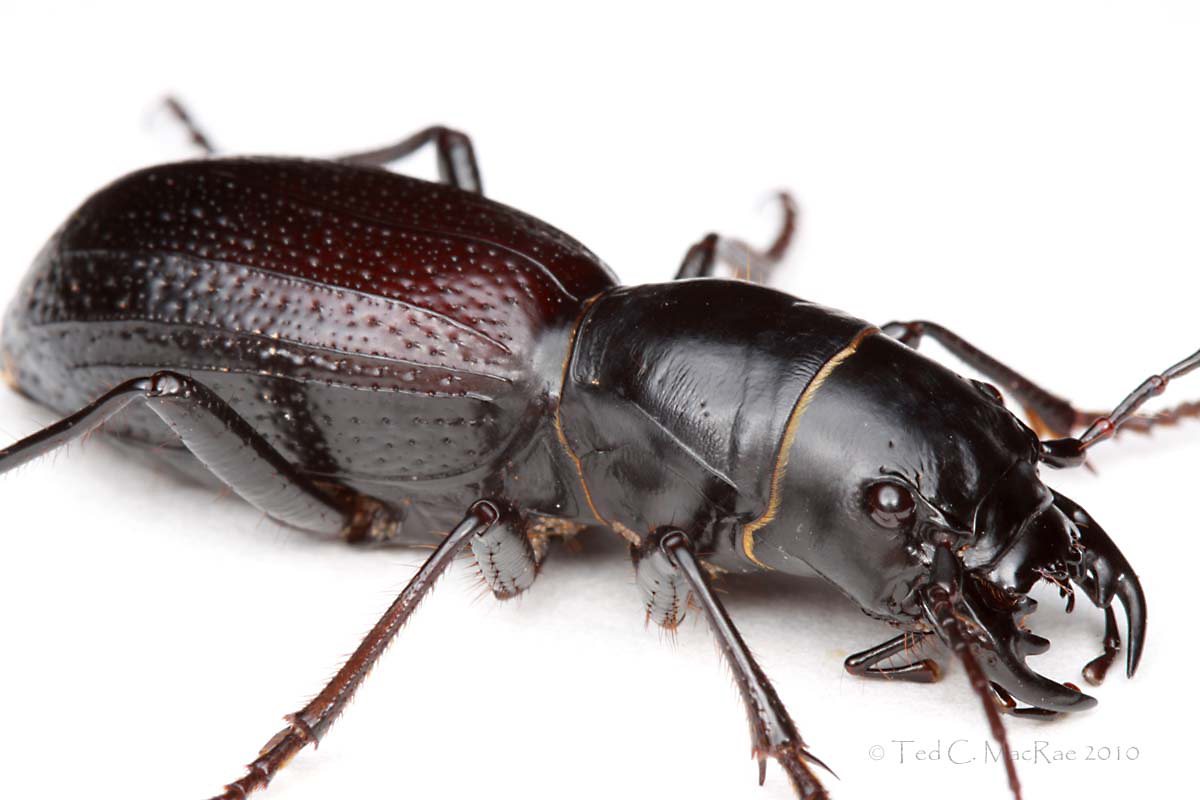
Amblycheila cylindriformis on white

It’s been four months now since I went to the Glass Mountains of northwestern Oklahoma on a hunch to look for Amblycheila cylindriformis (Great Plains giant tiger beetle).  The five adults that I brought back from that night are still alive in a terrarium of native soil, but to this point they have refused to lay eggs.  Despite feeding them regularly with fat Maduca larvae, there is obviously still something they need that I am not providing.  I’ve suspected that perhaps the terrarium that I have them in is too small, and I’ve also noted in the literature that larval burrows are often found clustered near the entrance of mammal burrows.  With this in mind, I combined the native soil from three separate terraria into one larger, deeper terrarium, packed the soil lightly, and used a spoon to create an artificial mammal burrow entrance.  Not long after placing the adults in their new home they began digging at the back of the burrow, eventually creating two separate tunnels leading in opposite directions (and fortunately against the container walls so that I can see inside the tunnels).  I was optimistic at first that finally I had given them what they wanted, but since digging the burrows they’ve just sat in them.  Perhaps they “know” that winter is coming and are just looking to hole up for now, so I suppose I’ll go ahead and place the terrarium in the 10°C incubator with the rest of my larval and adult rearing containers and wait until next spring to see what happens.

In the meantime, I thought I would share these recent photographs of one of them.  I had been wanting to take photographs of this species in a white box, which I have used with a few other species to generate some rather striking photographs (e.g., Gromphadorina portentosa, Buprestis rufipes, Scolopendron heros, Eleodes suturalis). The photographs in this post might look like they were taken in a white box, however, they were not.  I’ve been spending a lot of time lately trying to come up with a diffuser setup that is convenient for field photographs of wild insects in their native habitats.  Kurt’s do-it-yourself concave diffuser and Alex’s tracing paper diffuser work great with the Canon MT-24EX Macro Twin Lite Flash and the Canon MP-E 65mm f/2.8 1-5X Macro Lens, but as I mentioned in a previous post they do not work so well with the Canon EF 100mm f/2.8 Macro USM Lens and its longer working distance… or so I thought!  I’ve come up with a modified version of the concave diffuser that seems to be what I am looking for – it is easy to use, adds virtually no weight to the camera, is completely portable for field use, can be used with both the 65mm and 100mm macro lenses, and – best of all – costs virtually nothing.  The photographs in this post were taken with the first prototype, and now that the basic design and general dimensions seem to work I’ll try to make a more durable version. It’s simply a larger version of the concave diffuser – I found some very thick polypropylene foam that is sturdy enough to hold its shape but flexible enough to curl back and over the top of the flash heads, where the corners are held in place by Velcro. Essentially it forms a large “soft box” type diffuser in front of both flash heads. I cut the bottom inch off of a a 500-mL polypropylene beaker, then cut that in half and cut out all but a quarter inch of the bottom to form a sturdy but transluscent frame to hold the polypropylene foam against the flash head bracket on the front of the lens. Right now the foam is held in place by tape, but hot glue should do a better job, and the diffuser bracket is attached to the flash head bracket with Velcro. The whole rig comes off in a flash and lays mostly flat in the camera bag.

If this diffuser proves successful, it will eliminate the need for the different flash head extender brackets that I was considering.  I really didn’t want to go that route because even the cheapest models are rather costly, and all of them add bulk to the camera and create problems for those who need to switch lenses frequently (such as I do).  Of course, the real test is – does it achieve the desired result?  I’m quite happy with these initial photographs – the lighting is quite even due to the large “apparent” size of the light source, and the annoying double specular highlights that are the hallmark of the MT-24EX are much less apparent (though still slightly discernible).  The closest shots are at 1:1, while those of the entire beetle are between 1:1.5 and 1:2.  They are among the largest beetle species that I have photographed, so the range of magnifications used here pretty much covers the entire range that I typically use with this lens.  Wildflowers often require smaller mags and longer working distances, so it remains to be seen whether this diffuser/lens combination will be useful for them as well. 

All of the photographs in this post were taken with the 100mm macro lens (ISO100, 1/250 sec, F16) and direct MT-24EX macro twin flash using this new diffuser.  The beetle was placed on white filter paper and covered with a clear glass bowl until it settled against the side of it.  Once the beetle was quiet, I gently lifted the bowl and used micro-forceps to gently tug its legs into more appealing positions – surprisingly this did not cause it to become alarmed and try to flee (as long as I didn’t accidentally brush against one of its antennae!).  For the last photograph, I placed the beetle back in its terrarium and used the same techniques to get the beetle in a good position. 

Copyright © Ted C. MacRae 2010
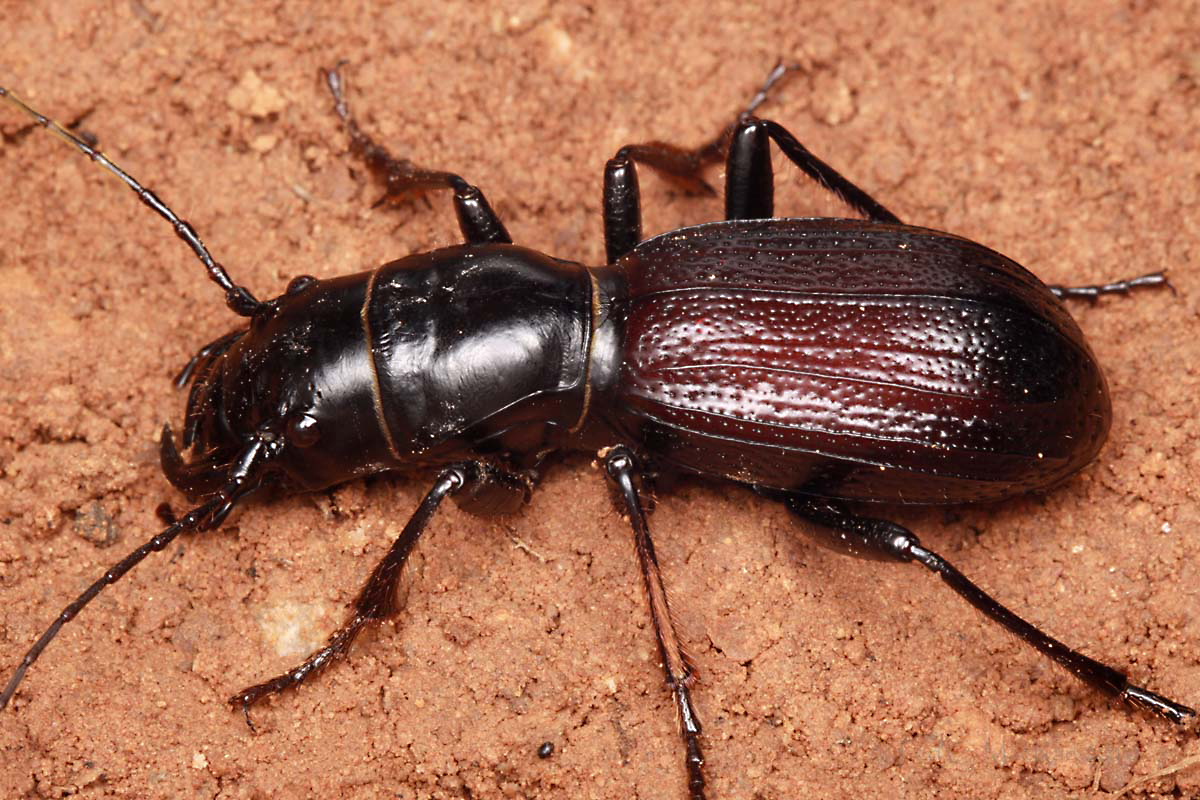
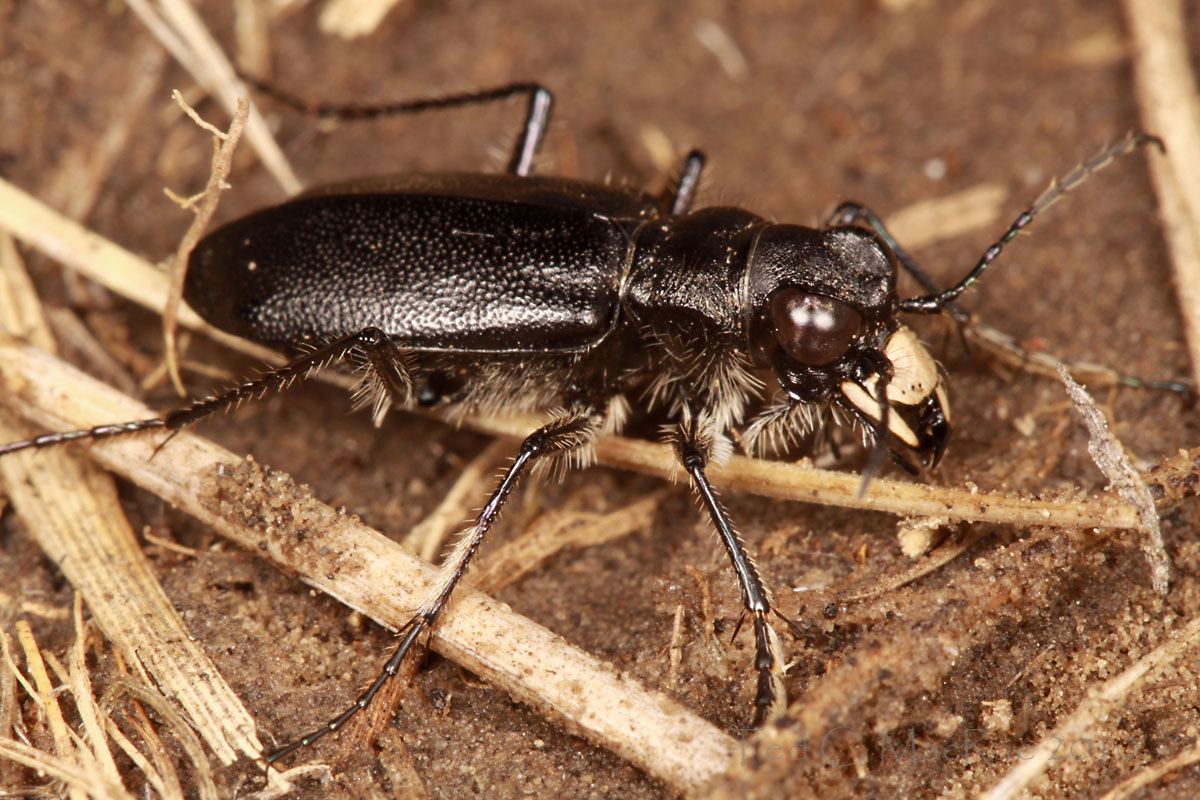
Cicindela nebraskana – Prairie Long-lipped Tiger Beetle

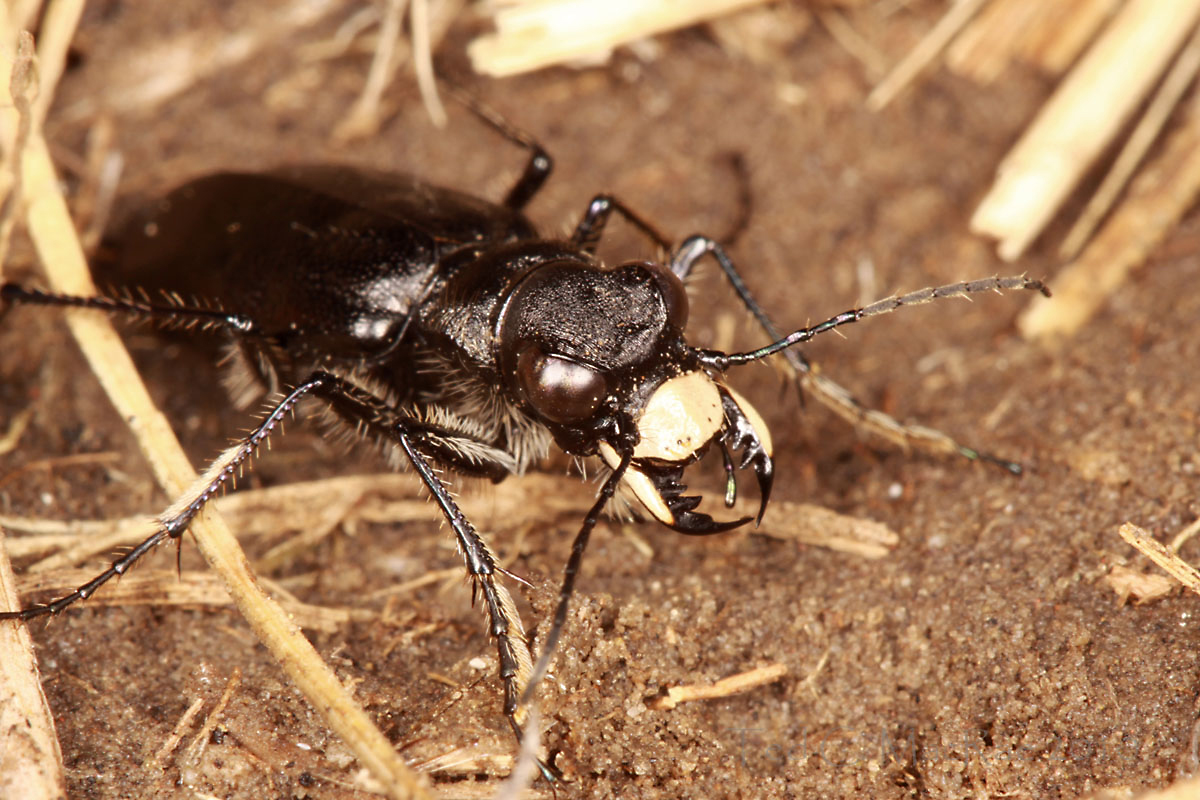
Cicindela nebraskana - the prairie long-lipped tiger beetle

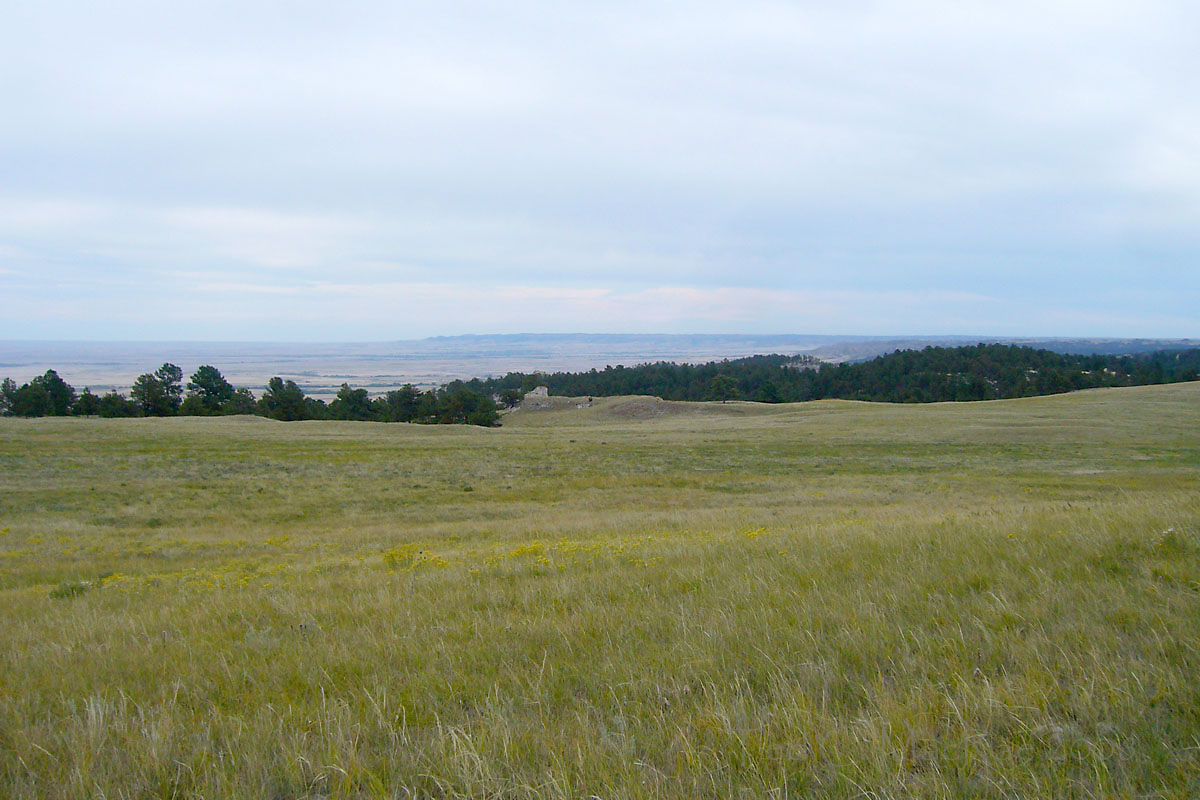
We were only halfway through Day #1 of five days in the field and had already achieved Goal #1 of the trip.  Despite that, it took a few hours before Chris and I were ready to tear ourselves away from our first stop in Fall River Co., South Dakota, where we were treated to the sight of glittering, wine-red adults of Cicindela pulchra bejeweling the charcoal-colored shale slopes.  However, the list of species that we wanted to see over the next several days was long, and eventually our pulchra-fever abated (barely) enough to head south to the Pine Ridge in Sioux Co., Nebraska to look for A-list Species #2 – Cicindela nebraskana.  Sioux Co., Nebraska is the type locality for this species (thus the name), but in reality it is a more western species whose distribution just barely sneaks into the northwestern corner of Nebraska (Pearson et al. 2006, Spomer et al. 2008).  I first saw this species at this very site two years ago, seeing only a handful of individuals and managing one harshly-sunlit, point-and-shoot image of one of them.  To my knowledge, this remains the only known field photograph of this species.

Shortgrass prairie atop the Pine Ridge, Sioux Co., Nebraska (photo taken September 2008).

This time, with a Canon 50D camera and 100mm macro lens in my backpack, I was much better equipped for vastly improved field photographs, but in contrast to the numerous individuals of C. pulchra that we saw earlier in the day, only a single C. nebraskana would turn up after intensive searching by Chris, Matt Brust, and myself in the vast shortgrass prairie sitting at the type locality atop the Pine Ridge.  I didn’t find it – Matt did – and the general rule with rare tigers is to capture the first individual rather than try to photograph it.  If no others are seen, photographing it later in a terrarium of native soil is better than trying to photograph it in the field and risk letting it escape.  Matt gave it to Chris, and at the end of the day when we realized we were not going to see another one, we prepared a terrarium of native soil, taking care to keep the surface as intact as possible so that an accurate replication of the field situation could be created when we photographed it later.

Tiger beetles "hunker down" when fatigued.

Although I prefer actual field photographs, the nice thing about photographing tiger beetles in confinement is… well, they don’t run away!  That’s not to say it is easy.  While they do settle down if left undisturbed for a while, once you start messing with them they quickly become agitated and start running in circles around the terrarium perimeter.  Much finger prodding is necessary to get them away from the edge and into a good spot for photographs, and rarely do they stay put for long.  When they finally do settle down, they tend to “hunker down” in a most unflattering pose (as above) – lacking the appearance of alertness that gives the true field photos their life.

A ferocious pose is struck after judicious prodding of the face and touching of the antennae.

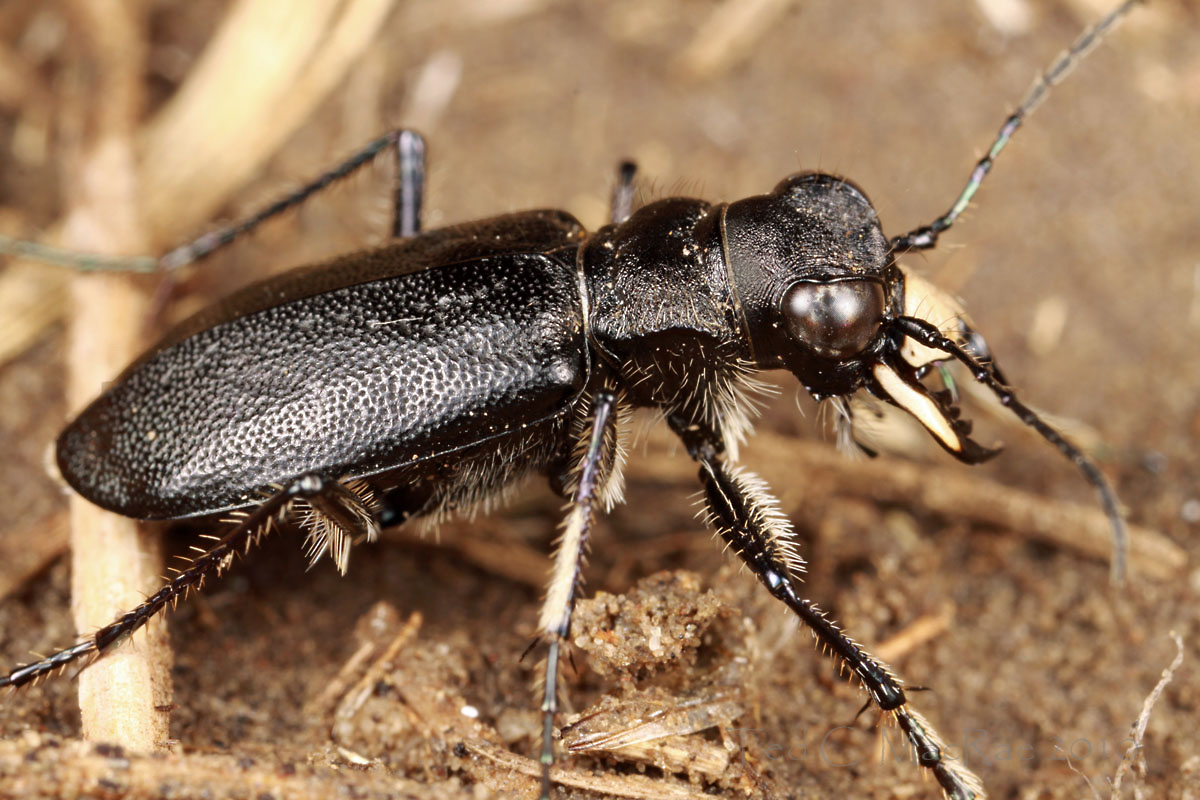
I’m a persistent (syn. stubborn) sort, however, and I’ve learned that I can wear them down and poke and prod them out of their hunker.  Just a light poke at the face will often make them back up and lift their front slightly – poke again and they often open their jaws half-cocked – a light touch on the tip of one antennae and they’ll turn slightly.  With practice and patience, hunkered down beetles can be coaxed into some remarkably aggressive-looking poses.  I like the last of these photos in particular because the oblique, jaws half-cocked pose shows off two nice features of this species – the quite long labrum (upper lip) compared to most other tiger beetle species, and the bright white labrum and mandibles of the males of this species (in females they are partially or completely dark).  The long labrum and jaws give this species a very long-faced appearance that distinguishes it immediately from the black morphs of Cicindela purpurea audubonii that occur with much greater frequency in the same habitats as C. nebraskana.

Photo Details:
1: Canon 50D w/ MP-E 65mm 1-5X macro lens (ISO 100, 1/250 sec, f/13), Canon MT-24EX flash w/ Sto-Fen + GFPuffer diffusers.
2: Panasonic DMC-FX3 (ISO 100, 1/400 sec, f/5.6), natural light.
3-4: Canon 50D w/ 100mm macro lens (ISO 100, 1/250 sec, f/16), Canon MT-24EX flash w/ Sto-Fen + GFPuffer diffusers.
All photos: Typical post-processing (levels, minor cropping, unsharp mask).

REFERENCES:

Pearson, D. L., C. B. Knisley and C. J. Kazilek. 2006. A Field Guide to the Tiger Beetles of the United States and Canada. Oxford University Press, New York, 227 pp.

Spomer, S. M., M. L. Brust, D. C. Backlund and S. Weins.  2008. Tiger Beetles of South Dakota & Nebraska.University of Nebraska, Department of Entomology, Lincoln, 60 pp.

Copyright © Ted C. MacRae 2010
Halloween ID challenge answer – Argiope trifasciata

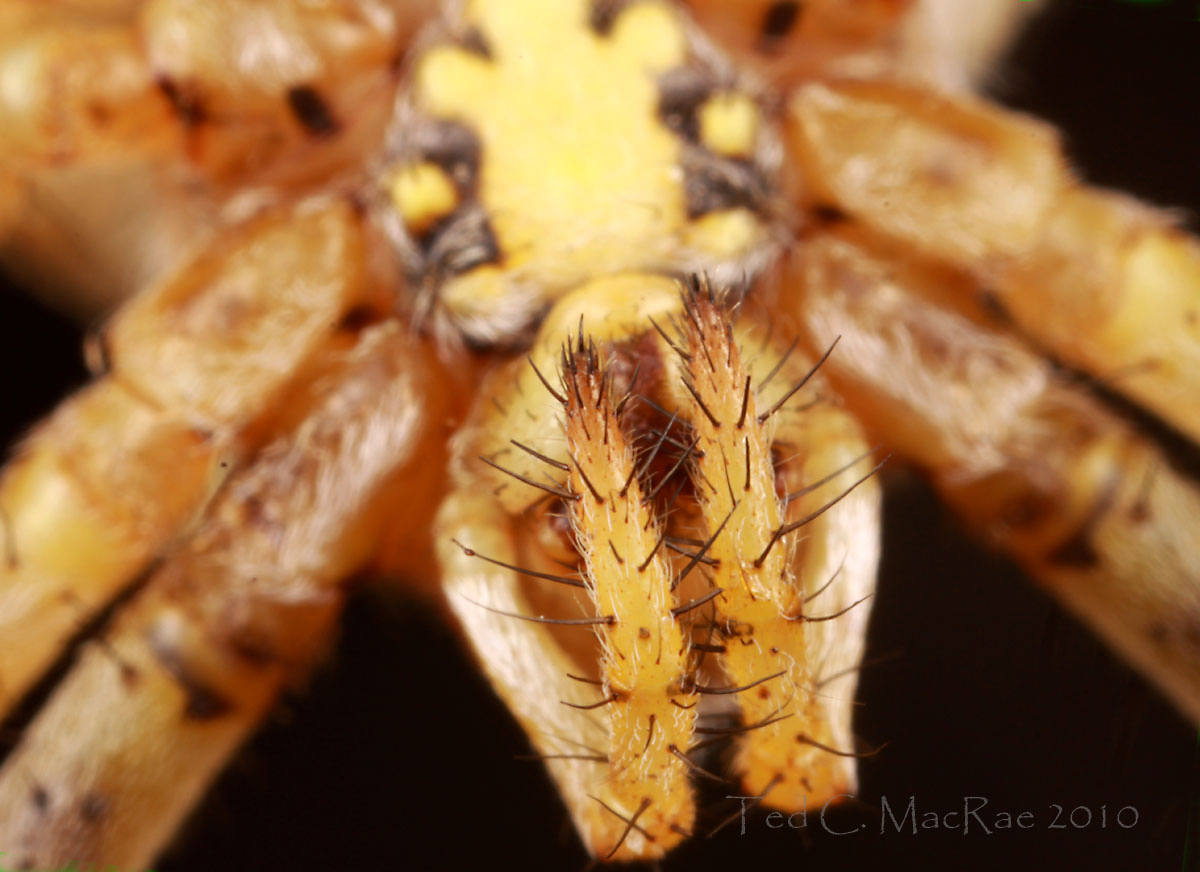
Here is another photo of the spider in the previous post with a closer view of its spiny pedipalps (mouth feeler thingys).  Troy Bartlett and BitB’s own James Trager got it right – the spider is, indeed, Argiope trifasciata, the banded garden spider (a.k.a. banded garden orbweaver, banded argiope, whitebacked garden spider, etc.).   I figured the genus would be easy, but the species might be a little tricky – at least for those in North America who might be tempted to conclude it was the larger A. aurantia (black and yellow garden spider, etc.).  The broken banding on the femora and generally lighter ventral coloration are usually enough to distinguish A. trifasciata from its more conspicuous congener.  Argiope trifasciata is also distinguished as one of the few truly cosmopolitan arthropod species, occurring naturally on all continents except Antarctica.

Both Troy and Dave Walter mentioned the conspicuous stabilimentum (heavy zig-zagging pattern) that Argiope spiders are perhaps best known for and that they often add to the center of their otherwise cryptic webs. Originally thought to possess a web-stabilizing function (hence the name), a variety of alternative explanations have since been proposed.  These include camouflage (to break up the body outline of the spider and make it less visible to predators), web protection (to make the web more visible to birds and prevent them from flying into and damaging it), prey luring (since it reflects ultraviolet light efficiently), thermal protection (by providing a shield against the sun), and a repository for excess silk.   An alternative hypothesis that I had not heard of but mentioned by Dave is that they serve as sponges for accumulating water for the spider to drink.  Webs with stabilimenta are more common and larger in exposed versus sheltered locations, and a recent study by Blackledge and Wenzel (1999) using A. aurantia found that webs with a stabilimentum suffered significantly less damage from birds (45% on average) than those without, but that they also caught fewer insects (34% on average).  The presence or absence of a stabilimentum, however, was not a significant factor in predation of the spiders by birds.  This implies not only a web protective function for the stabilimentum, but that there is an evolutionary trade-off between web protection and foraging success.  These authors concluded that variation in stabilimenta might be accounted for by a cost—benefit trade-off and that the decision by the spider to include a stabilimentum when building a web may be influenced by external factors such as prey density and web exposure.

Specific to A. trifasciata, a less well known but equally interesting aspect of its behavior is the use of web orientation for thermoregulation.   Tolbert (1979), in a study conducted in the southeastern US, found that web orientation was non-random during the hottest part of the summer, when spiders largely occupied east-west oriented webs with their silver/white dorsal surfaces facing south and their dark ventral surfaces facing north, and during October when the situation was reversed.  Orientation of the white/silver dorsal surface towards the sun presumably is done to help lower body temperatures, while orienting the ventral surface of the spider, which changes from silver to black as the spider reaches maturity, would maximize solar radiation for heat gain.  In contrast, Ramirez et al. (2003) found the species in coastal southern California never oriented their webs in a non-random fashion – rather, they always oriented them along an east-to-west axis with the mostly dark ventral surface of their abdomens facing south.  They suggested that dealing with a high heat load is not a significant problem in the predominantly cool environment of coastal southern California and that staying warm is the greater challenge for this mostly fall active species.

I’ll give 6 points to Troy for agreeing with me on everything, 4 to Dave for playing Devil’s advocate with the species and his unique alternative stabilimentum hypothesis, and 2 points to James for agreeing with Troy’s species ID. 🙂

Photo Details: Canon 50D w/ MP-E 65mm 1-5X macro lens (ISO 100, 1/250 sec, f/14), Canon MT-24EX flash w/ Sto-Fen + GFPuffer diffusers. Typical post-processing (levels, minor cropping, unsharp mask).

REFERENCES:

Blackledge, T. A. and J. W. Wenzel. 1999. Do stabilimenta in orb webs attract prey or defend spiders? Behavioral Ecology 10(4):372–376.

Ramirez, M. G., E. A. Wall and M. Medina. 2003. Web orientation of the banded garden spider Argiope trifasciata (Araneae, Araneidae) in a California coastal population. The Journal of Arachnology 31:405–411.

Tolbert, W. W.  1979. Thermal stress of the orb-weaving spider Argiope trifasciata (Araneae).  Oikos 32(3):386–392.

Copyright © Ted C. MacRae 2010
Flash solutions for the beautiful tiger beetle

Canon MP-E 65mm f/2.8 1-5X macro lens (f/13), Canon MT-24EX flash w/ concave diffuser.

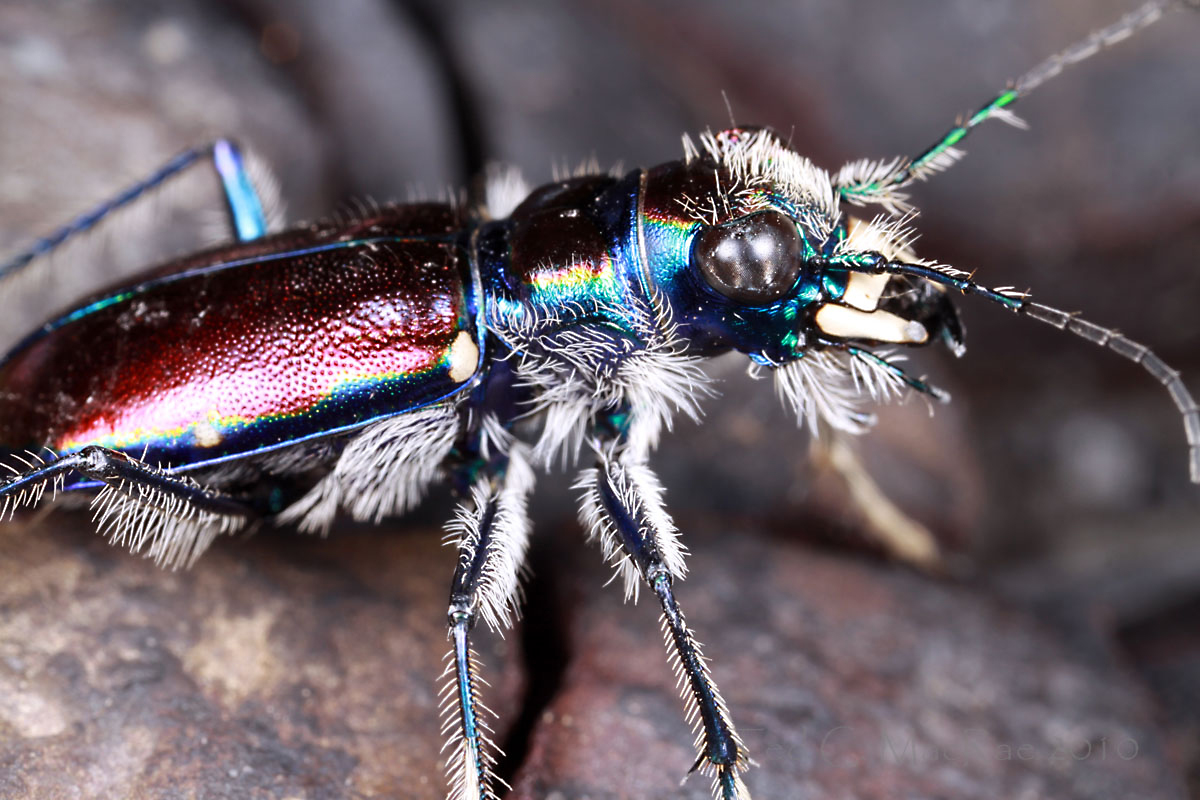
Recently I’ve been trying some different lighting and flash diffusion techniques with the Cicindela pulchra adults I brought back from South Dakota (see previous post).  While the beetles themselves are certainly among the most spectacular tiger beetles I’ve ever seen, I’ve been less than impressed with the photographs that I’ve managed to take of them.  Two factors have been largely responsible for this: 1) the smooth, shiny integument of the beetle reflecting the flash to create strong specular highlights, and 2) the colors, though brilliant, are also dark and difficult to bring out without further exacerbating the specular highlights.  Normally, the Sto-Fen+Puffer diffuser combination that I use does a pretty good job at diffusing the flash, but it just can’t handle these beetles.  To deal with this problem, I finally got around to trying out the do-it-yourself concave diffuser that Kurt at Up Close with Nature has been using with stunning results (similar to the tracing paper diffuser used so famously by Alex Wild at Myrmecos).  Photo 1 above and 2-3 below were taken with this diffuser on my Canon MP-E 65mm f/2.8 1-5X Macro Lens, and I’m rather pleased with these initial attempts.  I do need to figure out a better way to attach the diffuser to my Canon MT-24EX Macro Twin Lite Flash.

Canon MP-E 65mm f/2.8 1-5X macro lens (f/13), Canon MT-24EX flash w/ concave diffuser.

Canon MP-E 65mm f/2.8 1-5X macro lens (f/13), Canon MT-24EX flash w/ concave diffuser.

I’d have to say the lighting with this diffuser represents a considerable improvement over the Sto-Fen+Puffer diffusers using the same lens.  Compare especially Photo 3 above and 4 below – both taken with the MP-E 65mm lens at 1:1 and f/13 – Photo 3 was taken using the concave diffuser, while Photo 4 used the Sto-Fen+Puffer diffusers.

Canon MP-E 65mm f/2.8 1-5X macro lens (f/13), Canon MT-24EX flash w/ Sto-Fen+Puffer diffusers.

The problem with the concave diffuser is that it won’t work so well on my Canon EF 100mm f/2.8 Macro USM Lens due to its longer working distance.  I actually use this lens in the field as often as the MP-E 65mm lens, especially for the tiger beetles on which I focus (heh!) – not only do they rarely require more than 1:1 magnification, but they also rarely allow the ultra-close approach needed to use the 65mm lens.  The only solution is to find some way to get the flash heads closer to the subject to increase the apparent size of the light source, but so far I haven’t figured out a satisfactory way to do this.  Some photographers use the stalwart Canon Speedlite 580EX II Flash, equipped either with a do-it-yourself snoot diffuser or mounted on a bracket extender with a small softbox.  However, I am not a photographer, but rather an entomologist with a camera – I need to carry with me a net, vials, and in some cases a beating sheet and hatchet.  Both of the previously mentioned approaches for diffusing 100mm shots add far more bulk to the camera setup than I can accept.  I’ve been looking for extender brackets that will move the MT-24EX flash heads out closer to the subject to increase apparent light size and have found a few.  The Really Right Stuff B85-B Flash Bracket equipped with two FA-EX1 Flash Extenders and an extra Flash Mount looks like it would do the job quite well, but it is still bulkier (and vastly more expensive) than I would like.  The PhotoMed R2-C Dual Point Flash Bracket is a much less bulky and more reasonably priced option; however, the lack of any vertical adjustment capabilities is an insurmountable shortcoming.  Why Canon hasn’t themselves designed a lightweight, low-cost accessory for extending the MT-24EX flash heads out away from the lens is beyond me, and I’ve actually been toying with some ideas on how to do this myself using a couple of Kaiser Adjustable Flash Shoes.

Until I do figure out a solution, at least there is always the white box for any captive-held individuals (and yes, I have considered a small, collapsible white box to bring into the field – I’m not ready to resort to that just yet!):

Canon 100mm macro lens (f/16), Canon MT-24EX flash indirect in white box.

Photo Details: Canon 50D (ISO 100, 1/250 sec). Typical post-processing (levels, minor cropping, unsharp mask).

Copyright Ted C. MacRae 2010