Top Ten of 2008

For the first post of 2009, I begin with a look back at some of my favorite photos from 2008 (idea stolen from Alex Wild and others).  I initially hesitated to do a “best photos” post since I’m not really a photographer – just an entomologist with a camera.  Nevertheless, and with that caveat in mind, I offer ten photos that represent some of my favorites from this past year. To force some diversity in my picks, I’ve created “winning” categories (otherwise you might just see ten tiger beetles!). Click on the photos to see larger versions, and feel free to vote for your favorite. If so, what did you like about it? Was there a photo I didn’t pick that you liked better?  Enjoy!

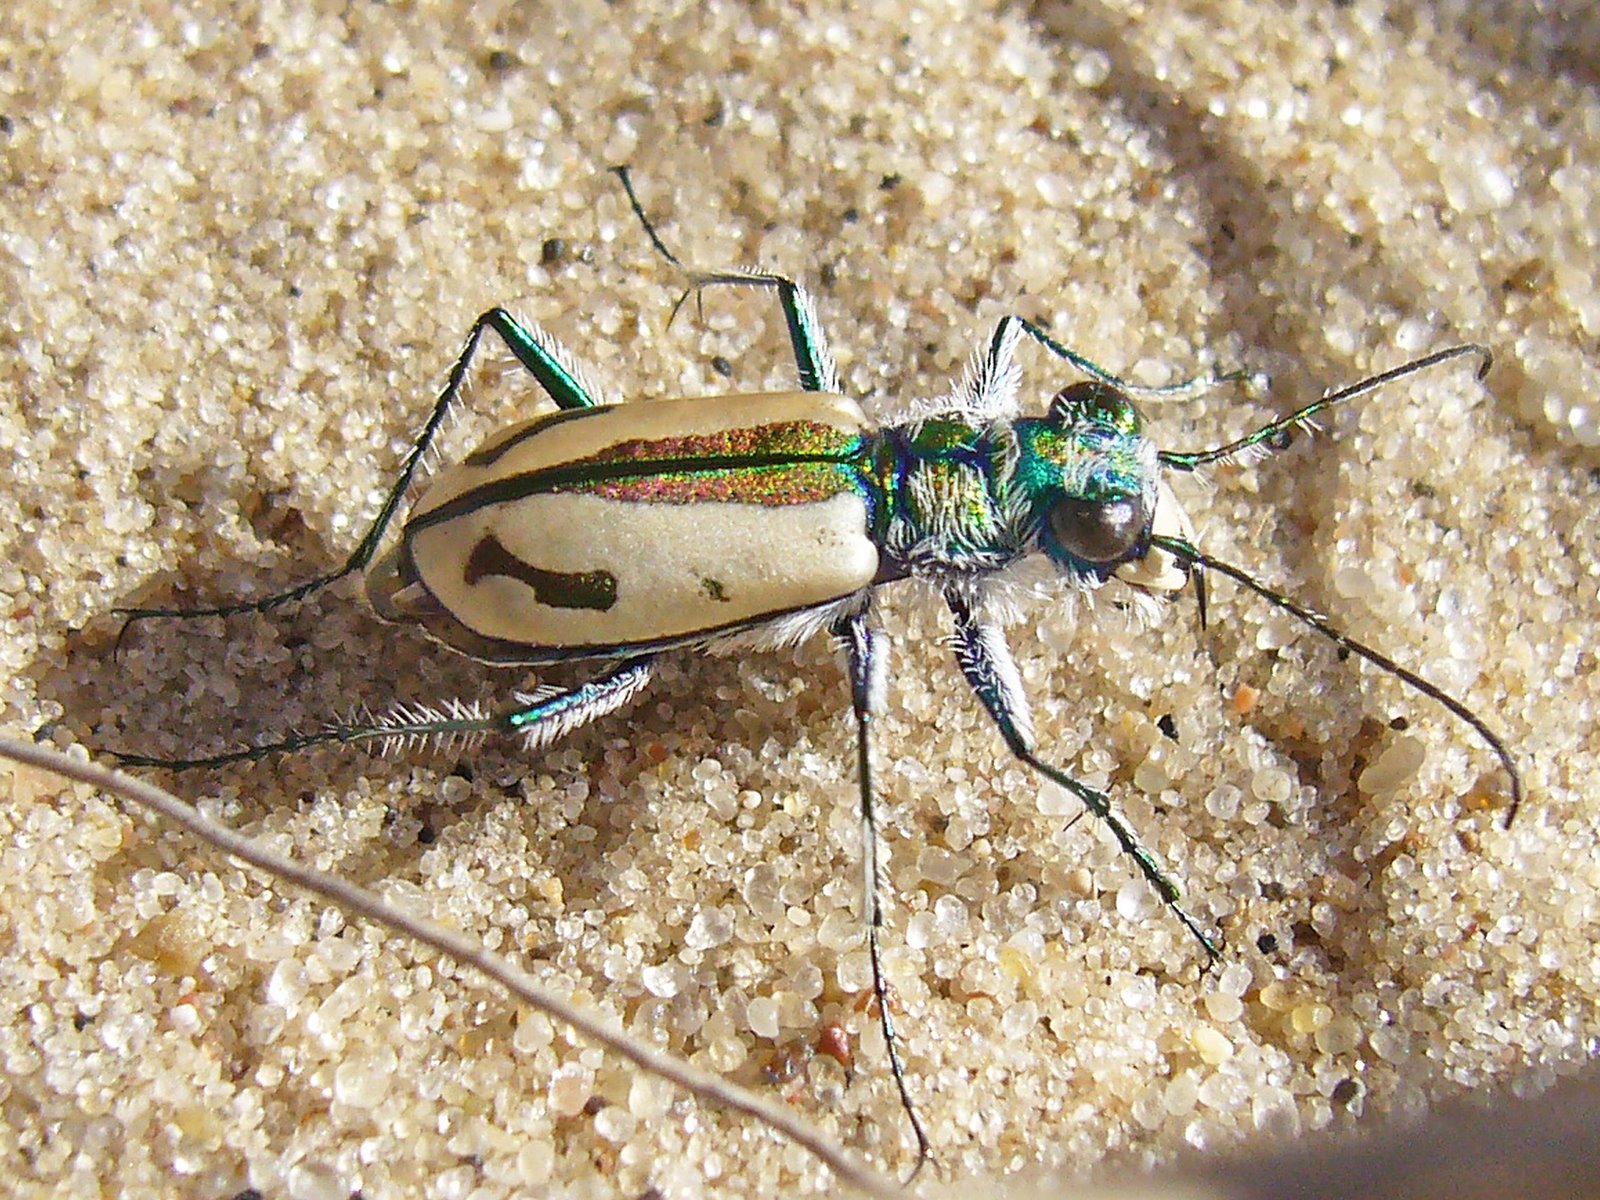
Best tiger beetle

Cicindela formosa generosa

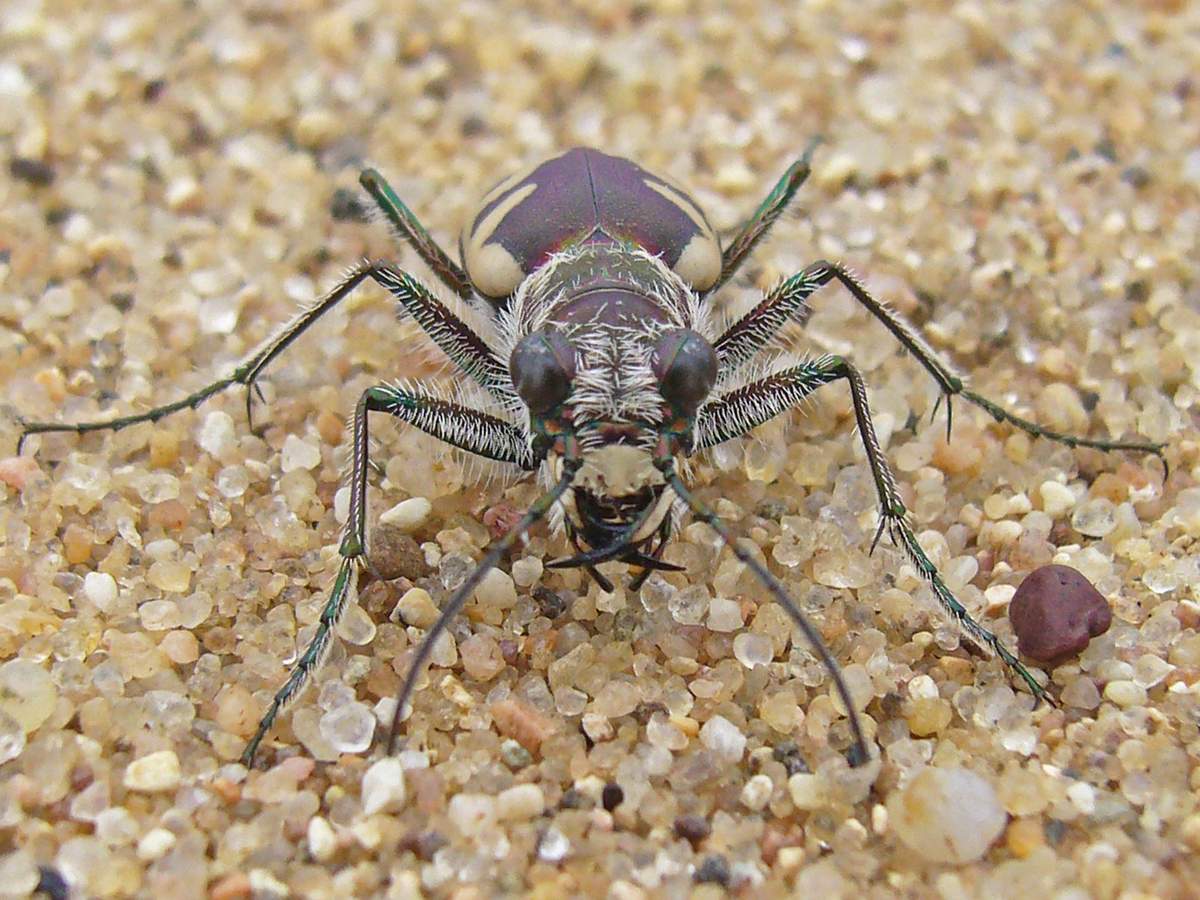
From “All the better to see you with, my dear!” (September 2008).  Picking a top tiger beetle photo was tough with so many to choose from.  Ultimately, I decided I really like these face-on shots, and of the several I’ve posted this one of Cicindela formosa generosa has the overall best composition, balance and symmetry.  I considered this one of Cicindela formosa formosa – with its half-cocked jaws, it probably has better personality.  However, the one above got the final nod because it is a true field shot of an unconfined, unmanipulated individual.

Best jewel beetle

Aegelia petelii

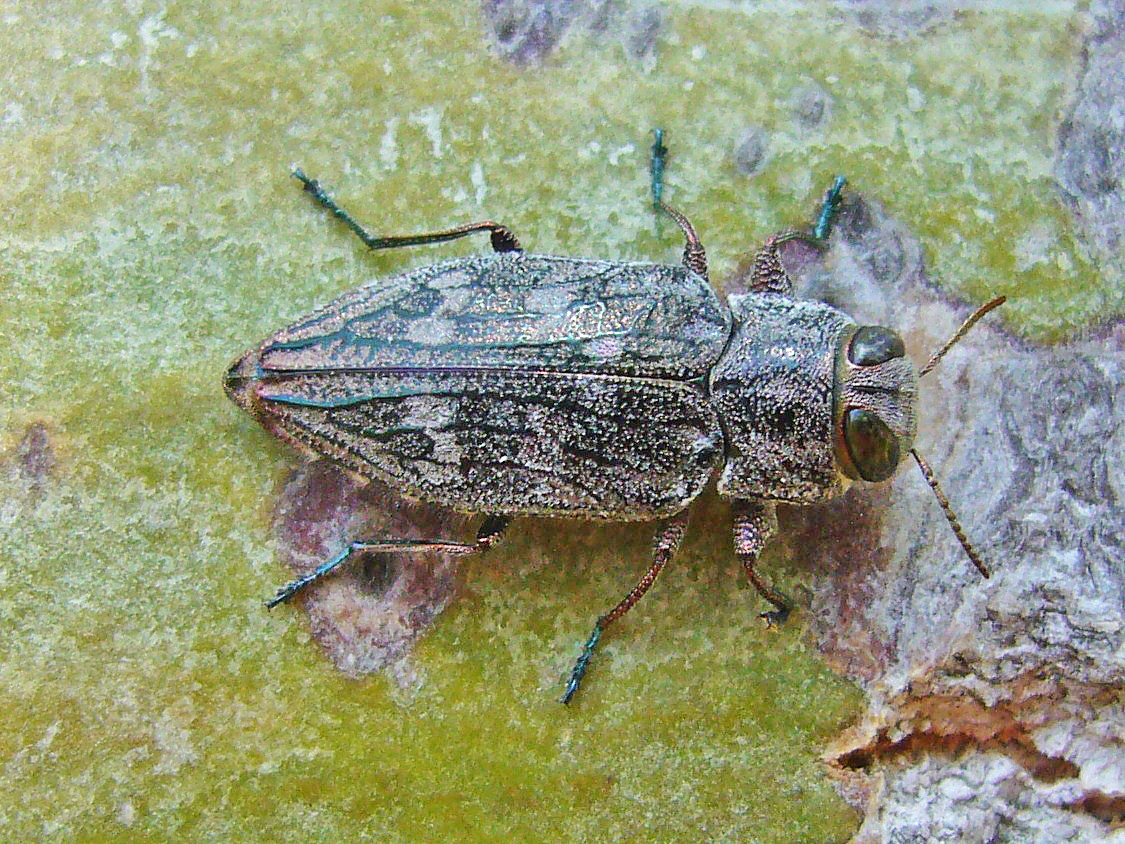
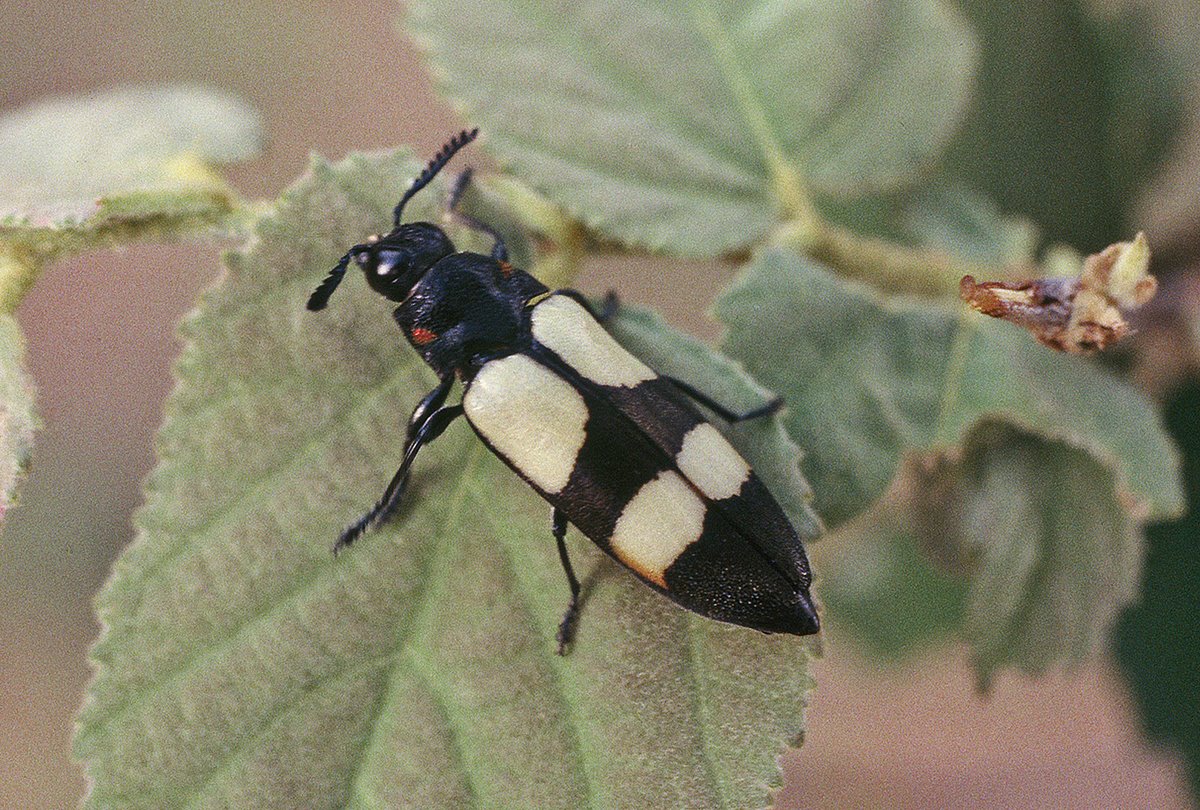
From Buppies in the bush(veld) (December 2008).  Although taken back in 1999, I just recently scanned and posted this photo of Agelia petelii from South Africa.  I like the bold, contrasting colors of the beetle combined with the soft colors of the host foliage.  Runners up included these photos of Evides pubiventris with its sumptuous iridescent green blending beautifully with the green background (but suffering slightly from shallow depth of field) and Chrysobothris femorata with its intricate surface sculpturing.

Best longhorned beetle

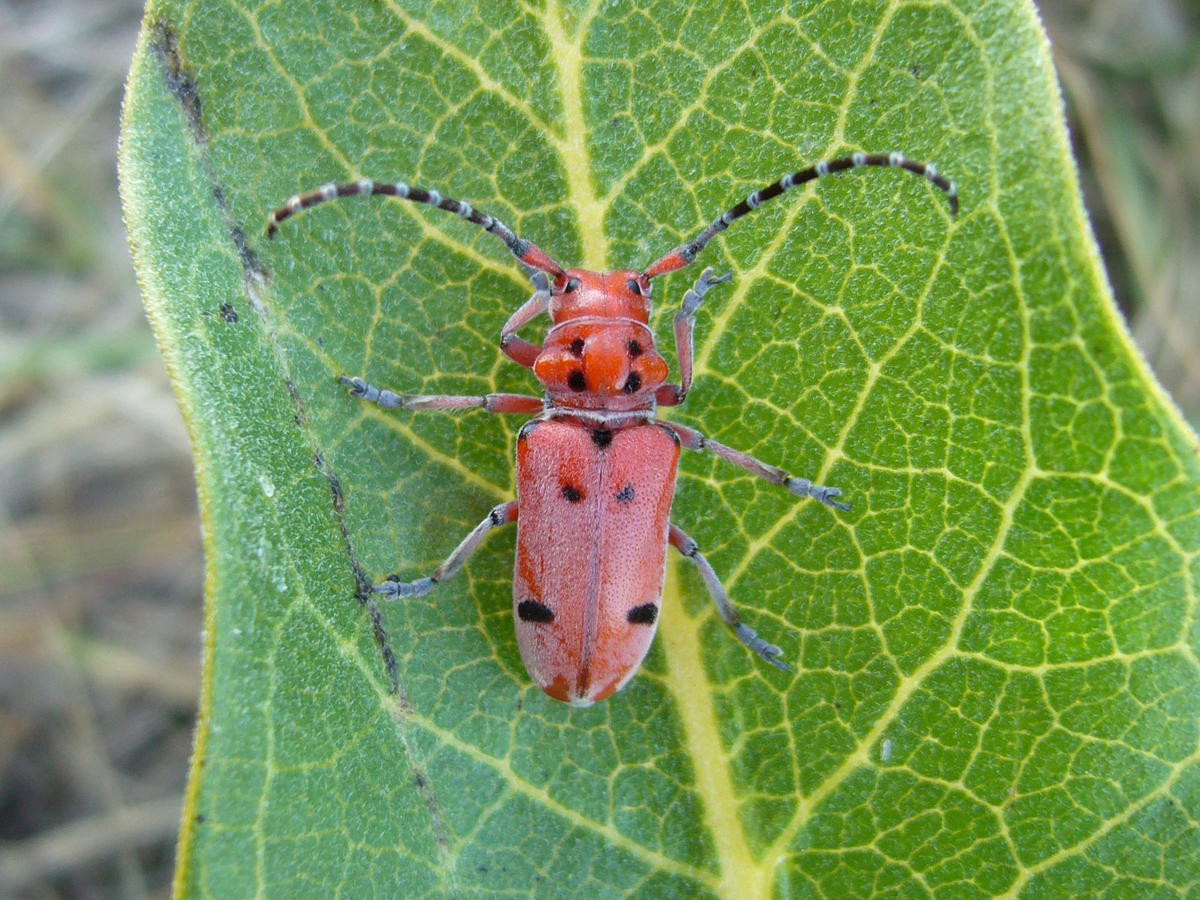
Tetraopes femoratus

From Rattled in the Black Hills (September 2008).  This was an easy choice – none of the other longhorned beetle photos that I posted during 2008 matched this photo of Tetraopes femoratus for clarity, composition, and the striking contrast between the red color of the beetle and the green color of the host plant.  I especially like the detailing of the body pubescence.

Best non-beetle insect

Proctacanthus milbertii

From Magnificently Monstrous Muscomorphs (November 2008).  I do like other insect besides beetles, and robber flies are hard to beat for their charisma.  This photo of Proctacanthus milbertii (which, as Chris Taylor pointed out, literally translates to “Milbert’s spiny butt”), has great composition and nice, complimentary colors.  I like contrast between the fine detail of the fly and the soft background.

Best non-insect arthropod

Argiope aurantia

From Happy Halloween! (October 2008). I didn’t have many non-insect arthropod photos to choose from, but this photo of a female Argiope aurantia (yellow garden spider) would be deserving of recognition no matter how many I had to choose from. I like the bold, contrasting colors and symmetry of the spider in front of the dappled background of this photo.

Best non-arthropod animal

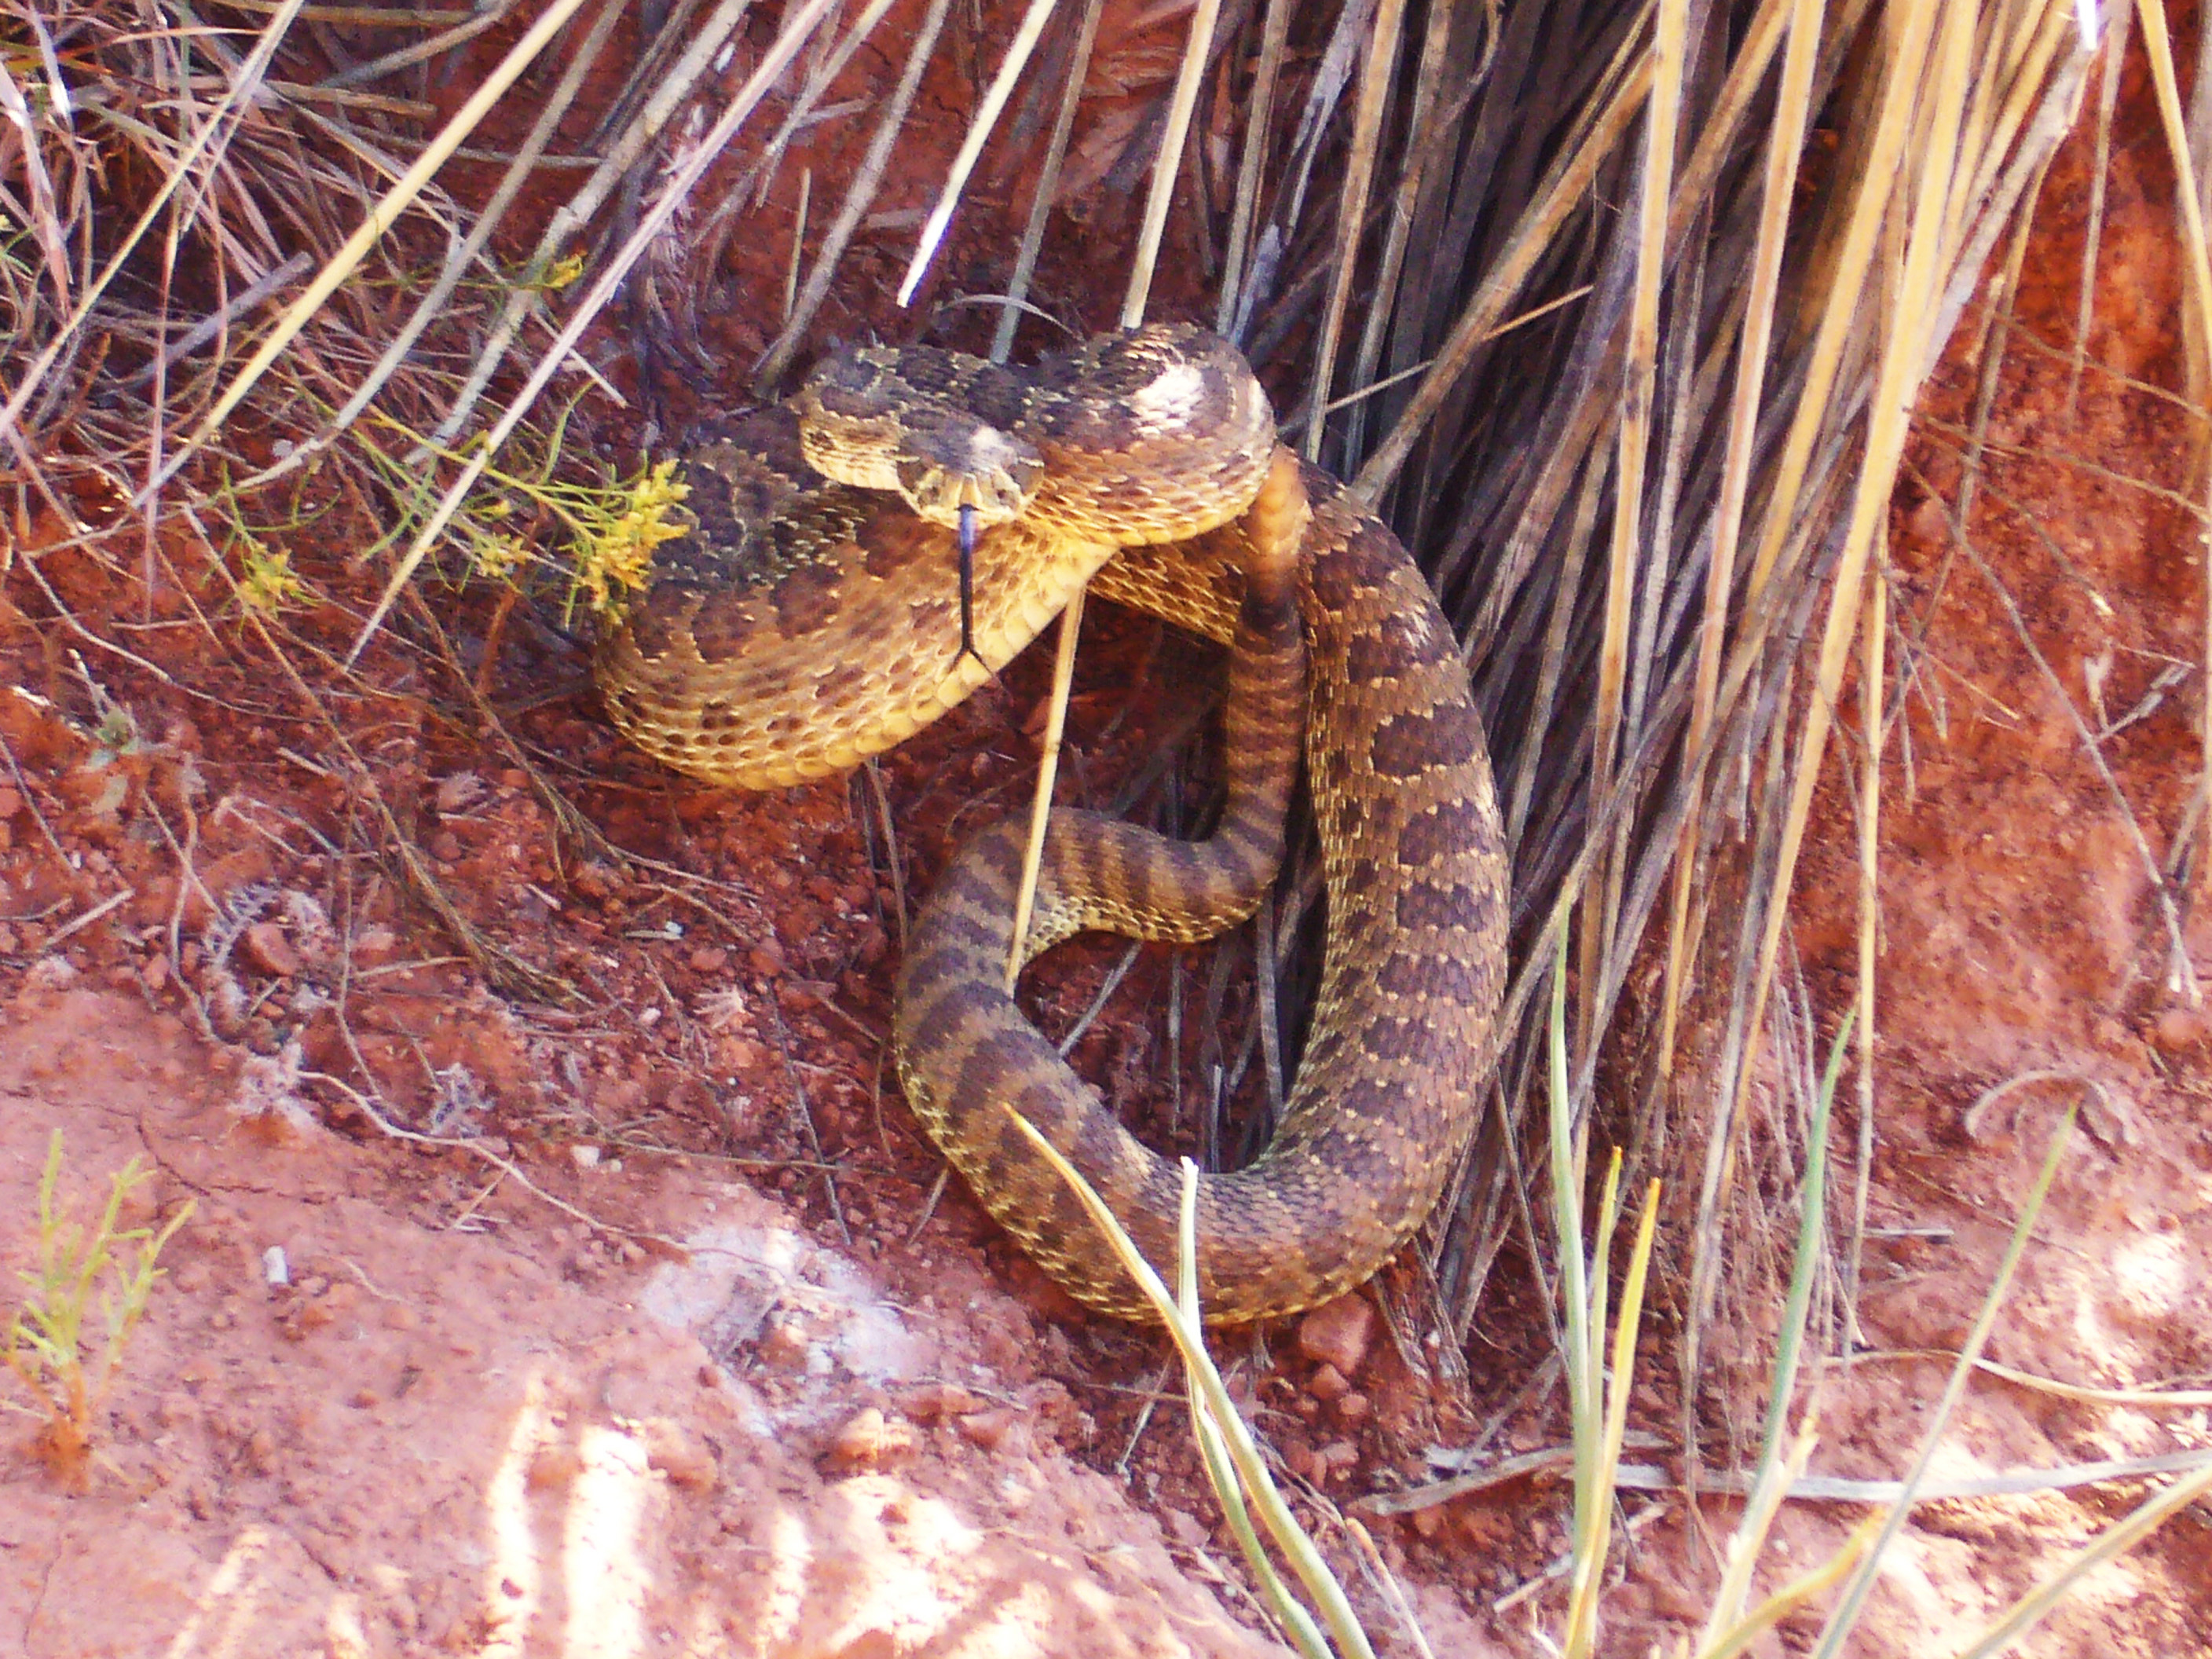
Prairie rattlesnake (Crotolus viridis)

Another one from Rattled in the Black Hills (September 2008).  This is admittedly not the best photo from a purely technical perspective – it’s a little out of focus, and the color is a bit off.  However, no photo could better convey the moment – confronted with a live, angry prairie rattlesnake (Crotalus viridis) (among the more aggressive species in the genus).  The forked tongue and rattle – blurred in motion – were icing on the cake.

Best wildflower

Victoria Glades

From Glades of Jefferson County (July 2008).  I had several wildflower closeups to choose from, but I kept coming back to this field shot of pale purple coneflower (Echincea simulata) and Missouri evening primrose (Oenethera macrocarpa).  The eastern redcedars (Juniperus virginiana) in the background are at once indicative of their preferred habitat (limestone/dolomite glades) and also testament to their threatening encroachment.

Best tree

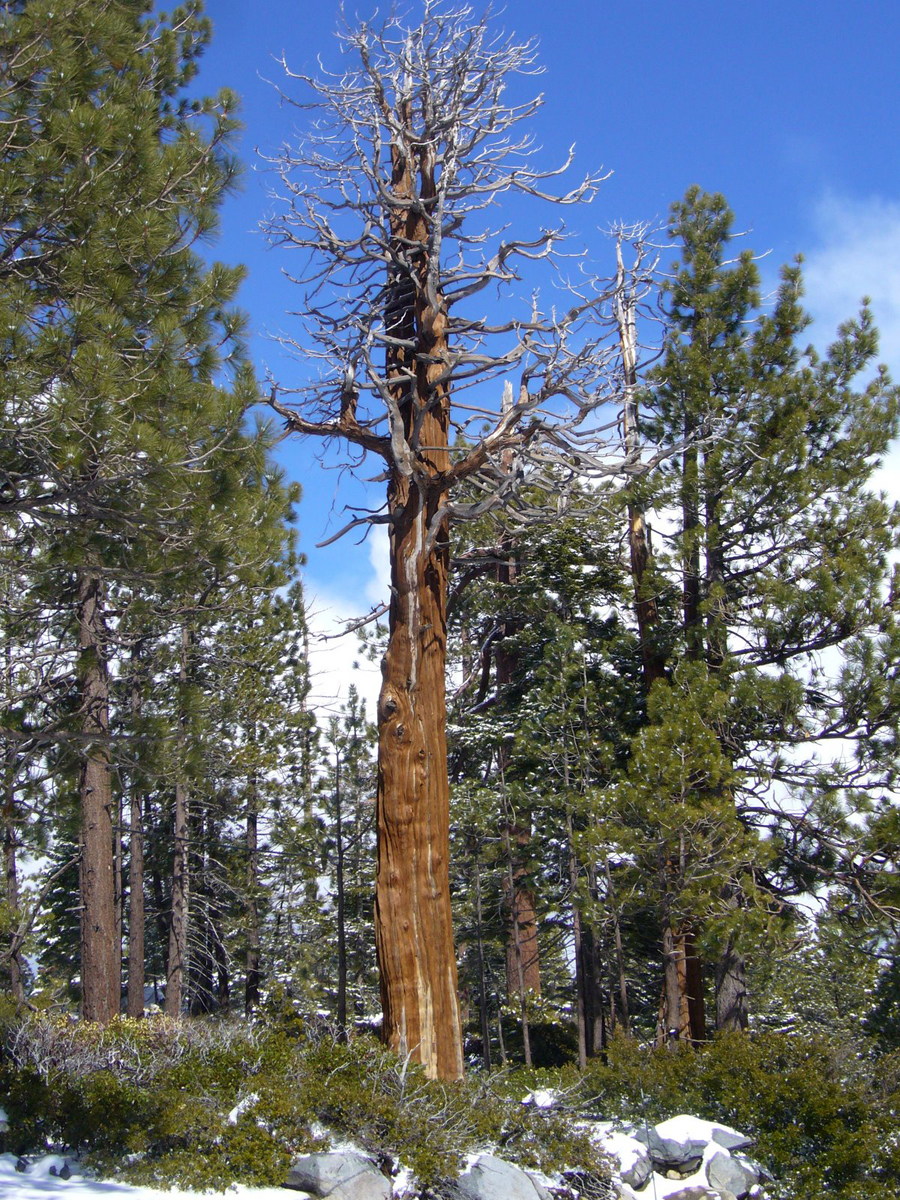
Calocedrus decurrens

From the very simply and aptly named Lake Tahoe, California (March 2008).  Incense cedar (Calocedrus decurrens), with its reddish, deeply furrowed bark and great height, is one of the most majestic of western conifers.  I was captivated by this tree – beautiful even in death and contrasting nicely with the surrounding green foliage.

Best rockscape

Pipestone National Monument, Old Stone Face

From Pipestone National Monument (April 2008).  “Old Stone Face” is one of Pipestone’s most recognizable geologic features, and the short angle of the sun on this early spring day provided nice detail to the cracks and fissures of the rock – almost appropriately adding a weathered “age” to this old man.

Best landscape

Emerald Isle, Lake Tahoe

Another one from Lake Tahoe, California (March 2008).  Few places on earth are more photogenic than Lake Tahoe, and this perspective overlooking Emerald Bay is among the finest views I’ve seen.  Brilliant blue skies and majestic snow covered mountains reflected perfectly from the still surface, with Fannette Island providing a perfect focal point for the photo.

Best miscellaneous

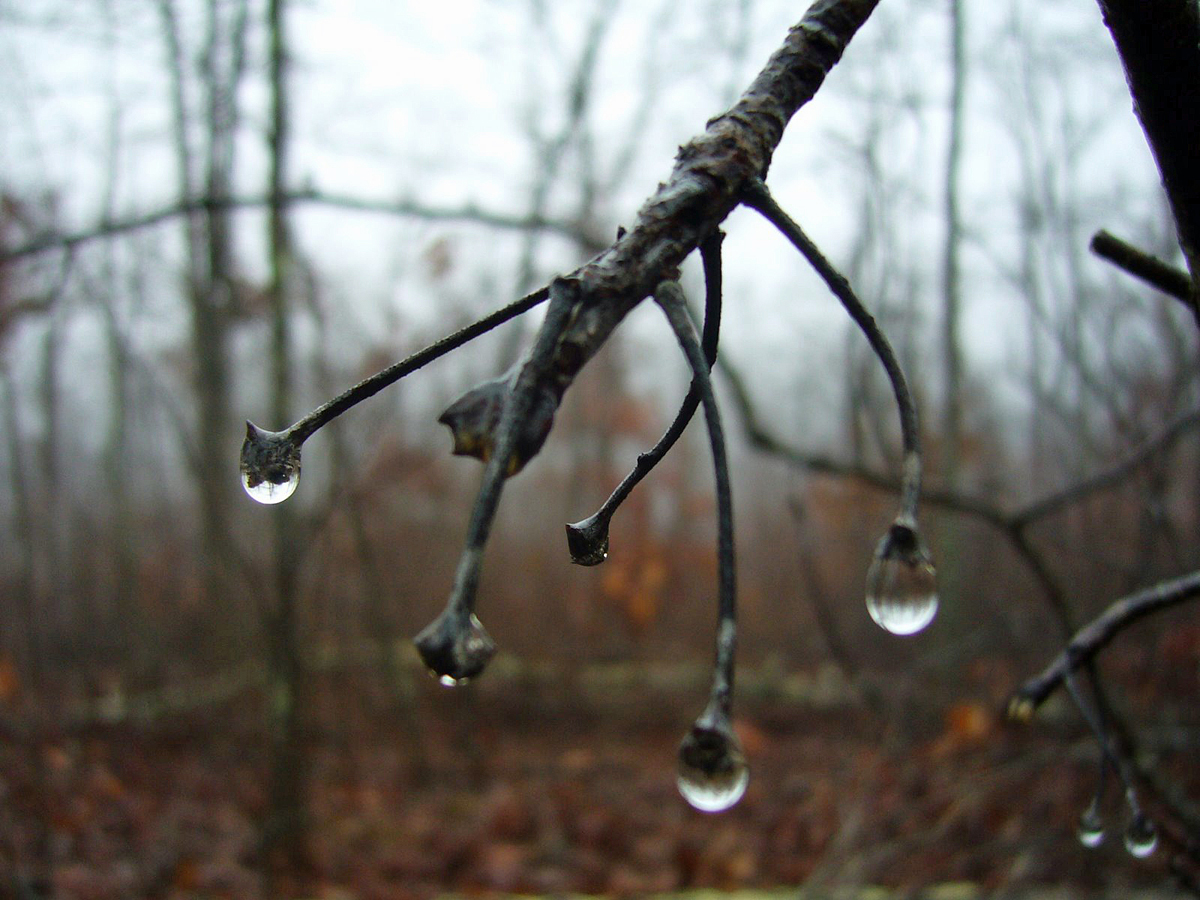
Water drops, Ozark Trail, Trace Creek SectionFrom Ozark Trail, lower Trace Creek Section (December 2007).  While technically not a 2008 photo, it’s close enough.  This was one of the first macro photographs I took with my camera, and it remains one of my favorites.  A chance occurence of an unlikely subject, created by cold temperatures and heavy moisture-laden air. I like the contrast between the water drops – sharp, round, and clear – with the vertical shapes of the leaf petioles and background trees.  Viewing the image full-sized reveals the reflection of the photographer in the leftmost water drop.

Subsequent edit: Okay, so after I put this post together, I realized I actually featured eleven photos – too much difficulty choosing, I guess. Let’s call it a baker’s ten.

Cicindela lengi vs. Cicindela formosa

Back to beetle blogging – I hope everyone enjoyed their holiday break as much as I. One of the tiger beetles that I most hoped to see on my trip to Nebraska and South Dakota last September was Cicindela lengi (blowout tiger beetle). This is another one of the several tiger beetle species confined to dry sand habitats in the central/northern Great Plains (Pearson et al. 2006). Its common name would suggest it prefers sand blowouts, the most barren of dry sand habitats and where the co-occurring C. limbata (sandy tiger beetle) can be found. In reality, it also can be found in slightly more vegetated habitats such as dune margins, sand flats, and sandy roadsides along with the much more common C. formosa (big sand tiger beetle) and C. scutellaris (festive tiger beetle). It can also be found occasionally on sand bars along rivers, where the aptly-named C. lepida (ghost tiger beetle) is likely to occur, and in the northern part of its range it even inhabits boreal coniferous forest along sandy roadsides.

Cicindela lengi lengiDespite its relatively loose habitat requirements, C. lengi is not a common species. In Nebraska it may be locally abundant (Spomer et al. 2008), and while planning my trip I was fortunate to get a specific locality from Steve Spomer and Matt Brust for one of these localized populations in far northwestern Nebraska. [Happily, that locality was very close to the locality where I would be looking for another priority species for the trip, C. nebraskana (prairie long-lipped tiger beetle)]. The site – a sandy roadside embankment – was characterized by a very fine-grained sand, which Matt Brust tells me the species appears to favor over the coarser-grained sands more typical of the Sandhills to the east. Success did not come easily – when no adults were seen at the site after two consecutive days of searching, I hedged my bets and extracted larvae that I hoped would represent this species for an attempt at rearing them out to adulthood in the laboratory. Persistence paid off, however – a hunch told me to make one more visit to the site after a couple days in the Black Hills, with two adults (and another C. nebraskana!) being my reward.

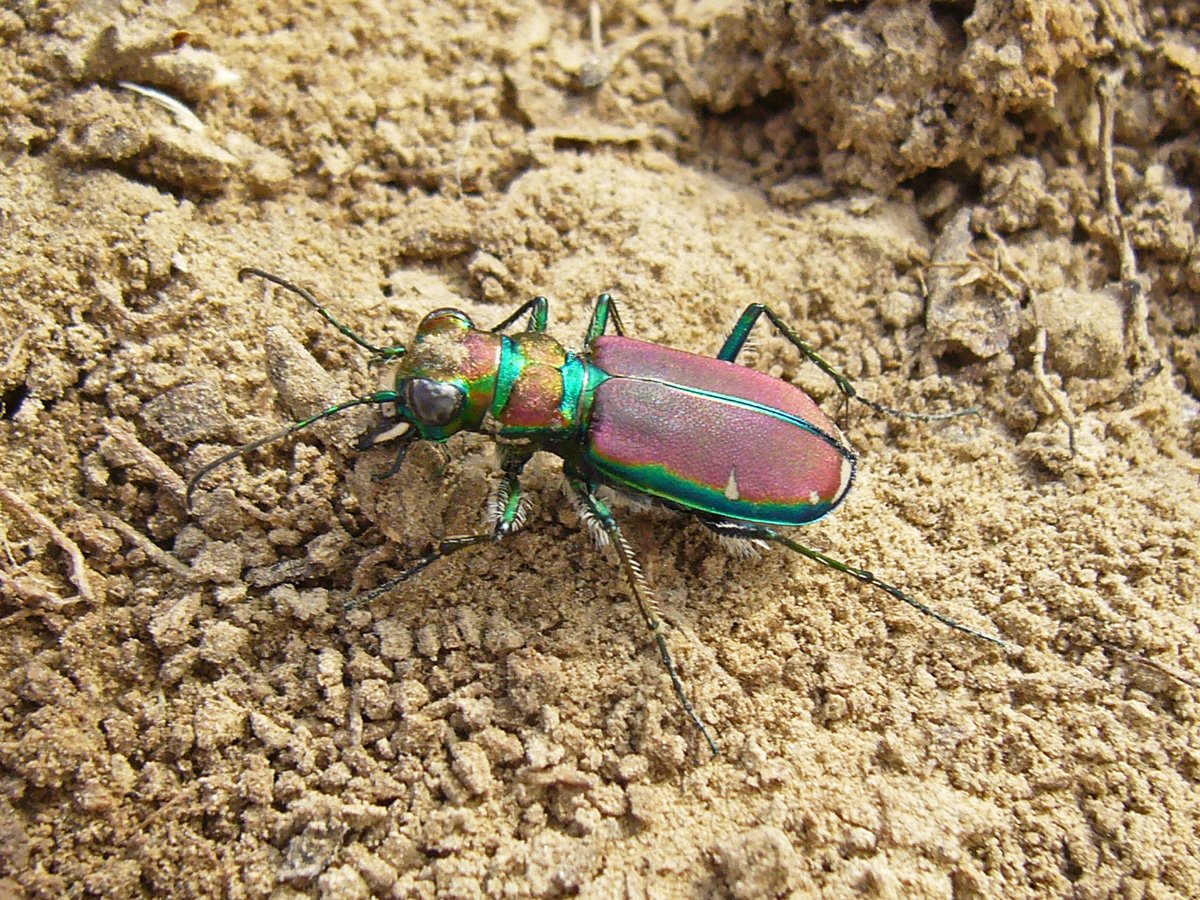
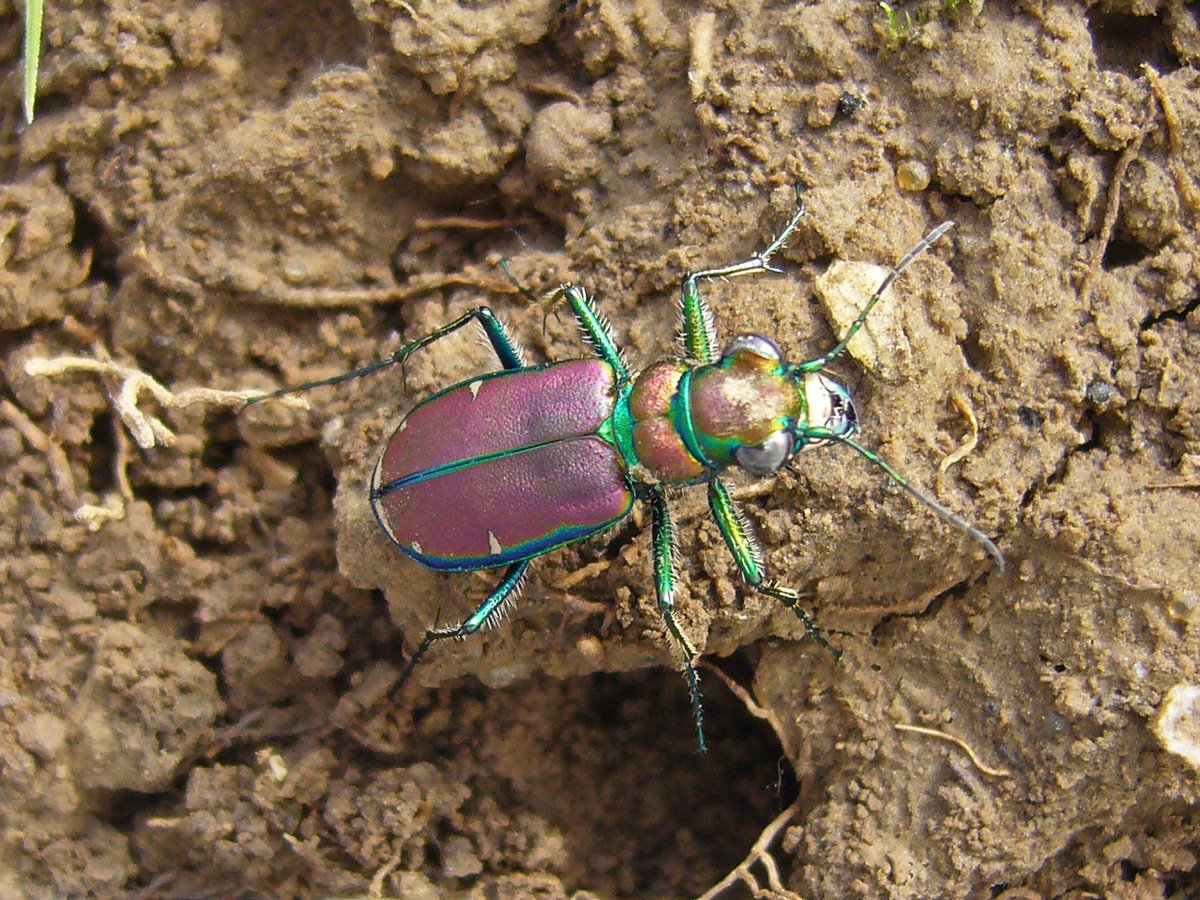
The individual shown in the above photo was an unexpected surprise. It was captured a day later in the Sandhills proper at a locality where I expected to see not this species, but C. limbata (which I did succeed in finding at a nearby locality – see “Cicindela limbata – epilogue“). When I first saw this individual, I thought it was the ever present C. formosa (pictured below), which it greatly resembles and which, along with C. scutellaris, occurs commonly in suitable sand habitats throughout the Sandhills. Cicindela formosa formosaSomething about the way it flew gave me pause, however, and after capturing and looking closely at it in my hand I realized what it was. Cicindela lengi is distinguished from C. formosa morphologically by its slightly narrower form and longer, narrower labrum, but the quickest field identifier is the obliquely straight humeral marking (“C”-shaped in C. formosa). There are subtle behavioral differences also – both species are alert and quick to fly, but C. lengi lands quickly after a short flight, whereas C. formosa flies further and tends to land with a comical bounce and tumble or two across the sand. Cicindela lengi and C. formosa are not closely related despite their similar appearance – the former is assigned to subgenus Cicindela (Tribonia), while the latter is assigned to the nominate subgenus. The individual pictured above represents the nominate C. lengi lengi – populations north of Nebraska and Colorado exhibit a distinct coppery underside to the thorax and are assigned to subspecies C. lengi versuta, while populations in the southwestern part of its range show broadly coalesced elytral maculations and are assigned to subspecies C. lengi jordai.

REFERENCES:

Pearson, D. L., C. B. Knisley and C. J. Kazilek. 2006. A Field Guide to the Tiger Beetles of the United States and Canada. Oxford University Press, New York, 227 pp.

Spomer, S. M., M. L. Brust, D. C. Backlund and S. Weins. 2008. Tiger beetles of South Dakota & Nebraska. University of Nebraska-Lincoln Special Publication, 60 pp.

You messin’ with me?

Cicindela formosa formosa

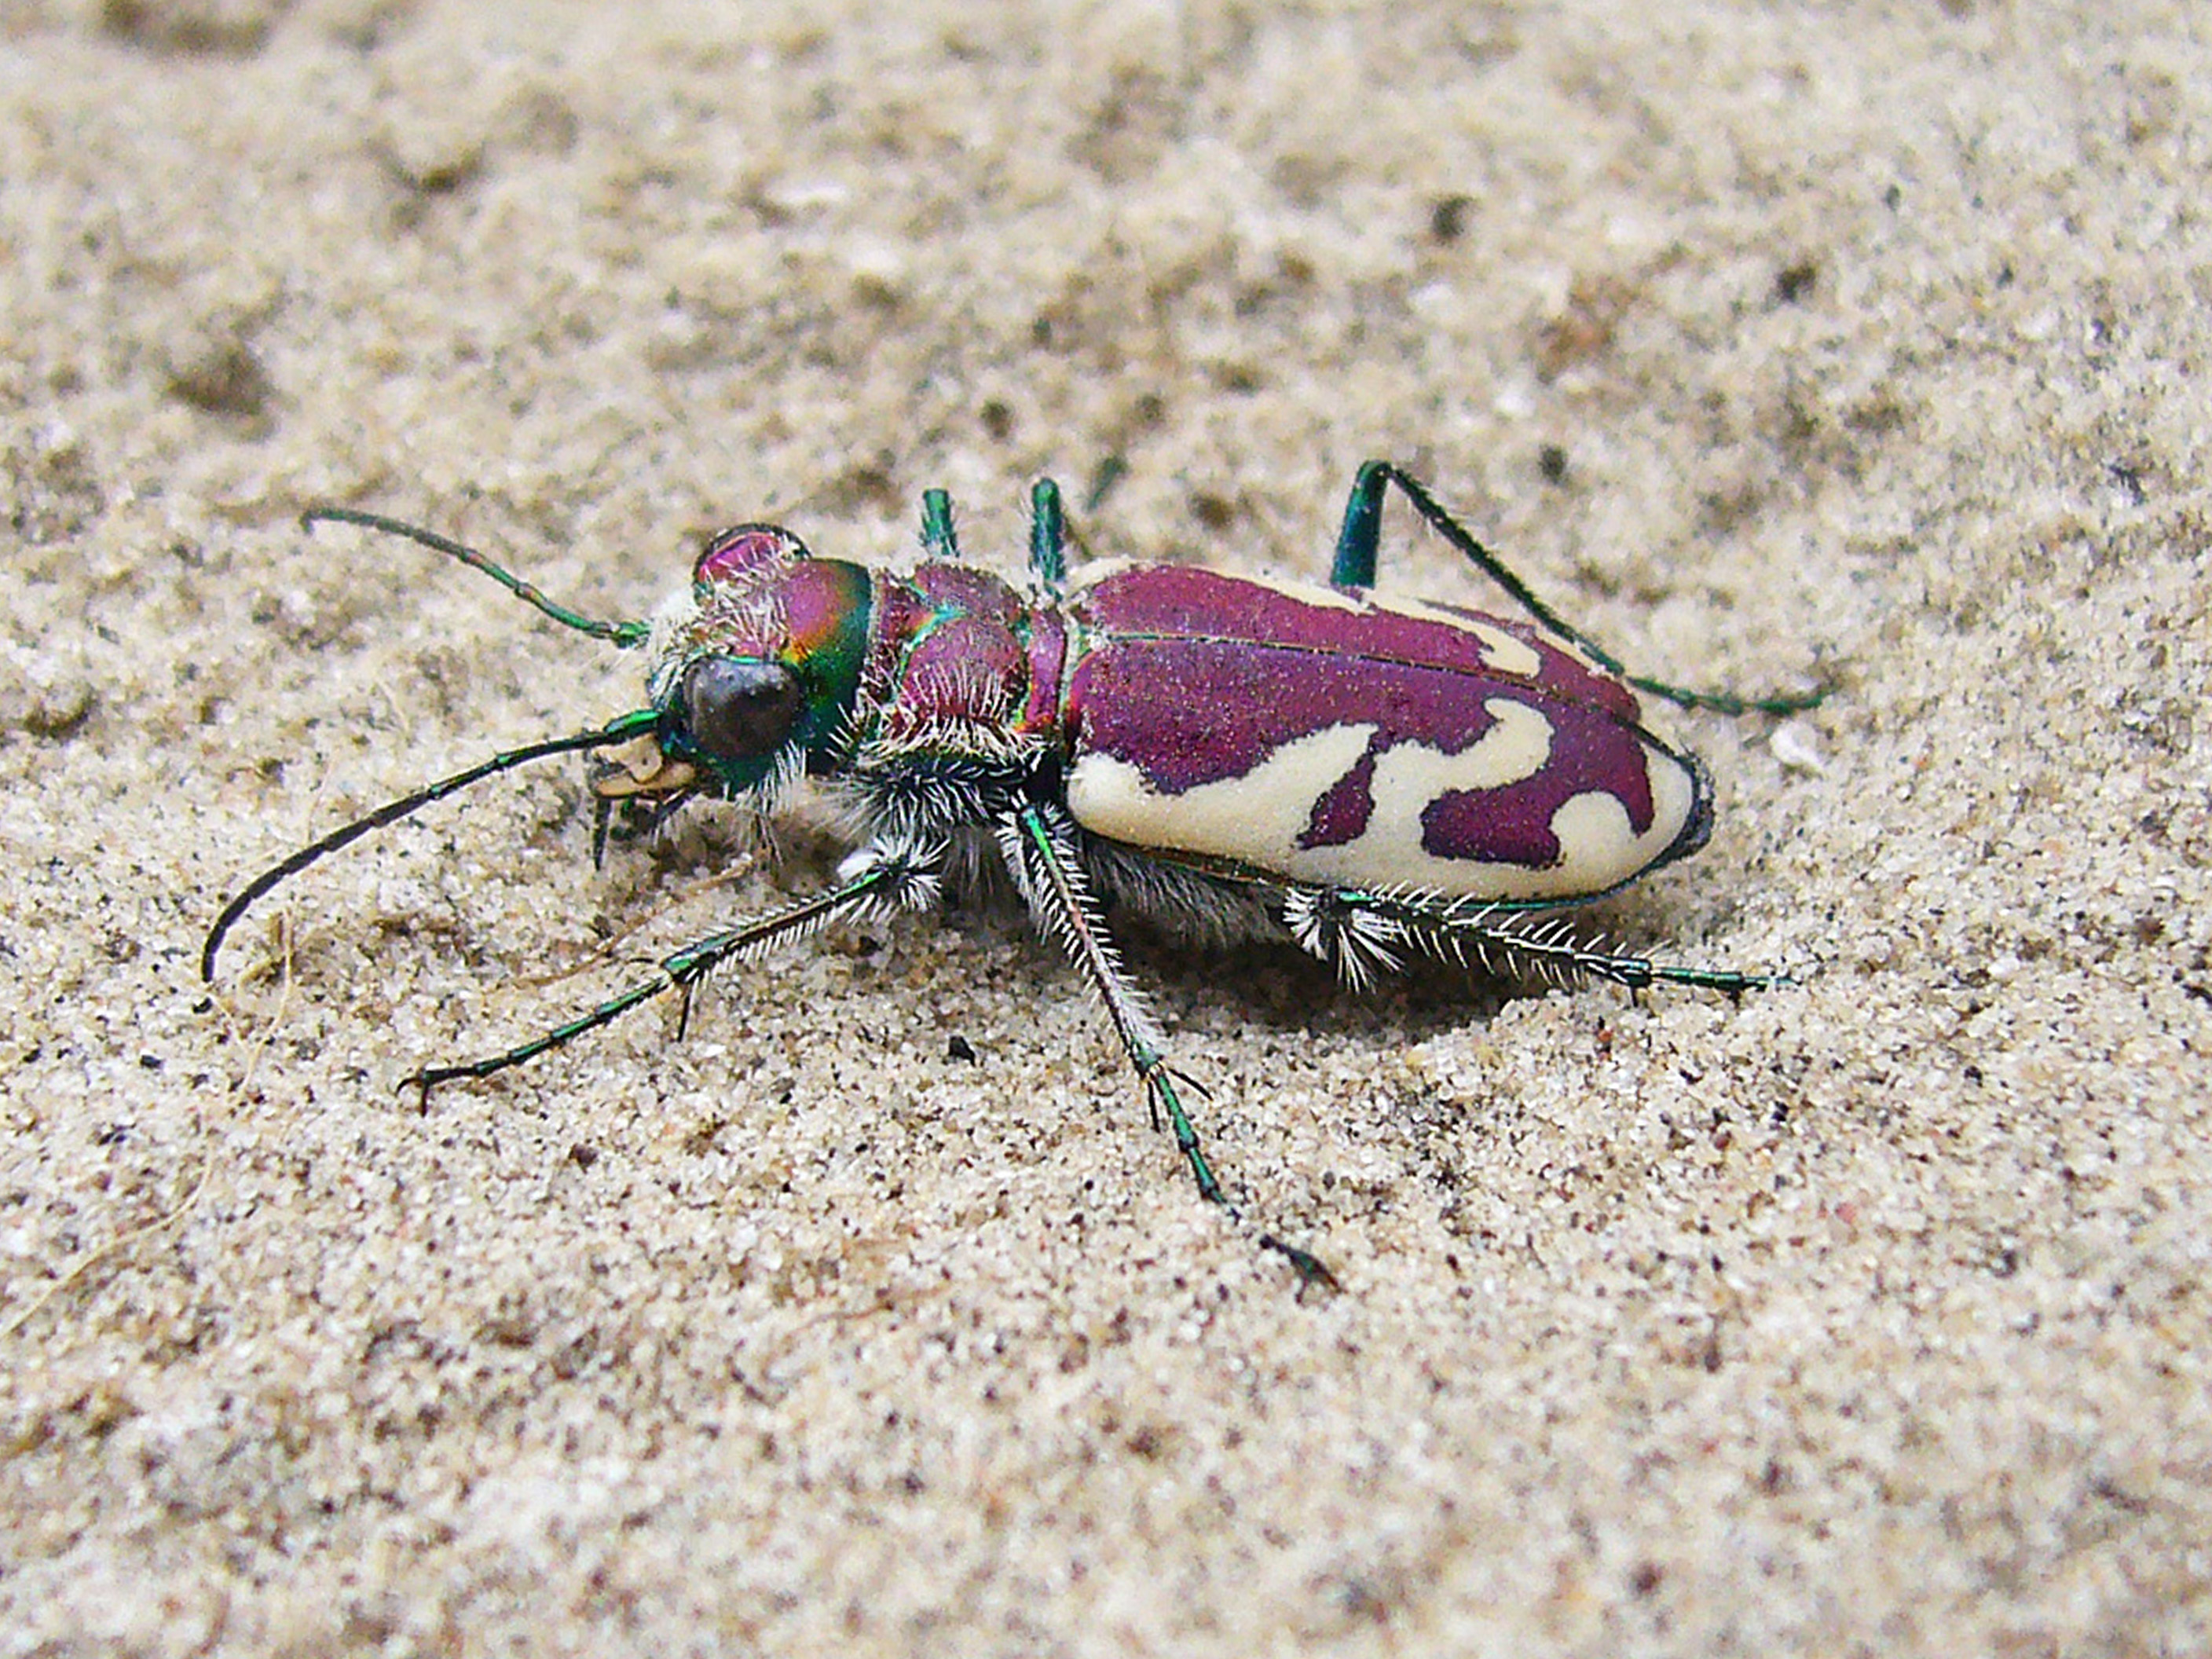
This is another one of the tiger beetles I brought back alive from the Sandhills of western Nebraska since I was unable to get any good photographs of this species in the field.  If this photo looks familiar, you may recall this headshot of another individual, representing the eastern subspecies (Cicindela formosa generosa), that I took back in September in southeast Missouri.  Compare the two photos to see the distinctly reddish dorsal coloration of nominotypical C. formosa versus the darkened coloration of C. formosa generosa.  Nominotypical C. formosa also has a much more violaceous ventral coloration.

If this guy looks a little angry, it’s because he is! I had prodded and poked him for some time by the time this photo was taken, trying to coax/force him away from the edge of terrarium in which I had him confined.  Every time I thought I had him sitting still in a good position, he would run suddenly and make a beeline to the edge – a most unphotogenic place.  He even reached up a few times, seemingly out of shear frustration, and bit at my finger while I tried to push him back away from the terrarium wall (talk about biting the hand that feeds you!).  Finally I got him sitting still in the middle of the terrarium – his half-cocked mandibles suggesting exhaustion or rage, or maybe both.

Like the Cicindela limbata individual from the same locality that I brought back alive for photographs, this little beast lived for 10 weeks in his terrarium before, ahem… donating his body to science.   Also like C. limbata, he amusingly reached up and grabbed caterpillars directly from the forceps almost every time one was offered.  I think my colleagues in the lab enjoyed feeding time as much as the tiger beetle!

Cicindela limbata – epilogue

In my Lucky 13 post, I featured Cicindela limbata (sandy tiger beetle) from north of Grand Island, near the easternmost edge of the Nebraska Sandhills. This species is restricted to dry sand blow out and dune habitats away from water, thus its distribution in Nebraska largely coincides with that of the Sandhills themselves. Nebraska populations are assigned to the nominate subspecies, which is characterized by extensively developed white maculations on the elytra, Nebraska, Grant Co., nr. Hyannis, 3.4 mi S Hwy 2 on Hwy 61, 26.ix.2008, coll. T.C.MacRaewith the sutural area and small discal markings metallic green or blue. The whitish areas on the elytra and dense pilosity on the undersurface, along with their habit of digging into the sand during the midday hours, are obvious adaptations for reflecting heat and avoiding the high temperatures that occur in their white sand habitats. In the more eastern areas of the Sandhills, the green sutural areas of the elytra are suffused with a reddish cast (see this photo in Lucky 13), while in populations further to the west no such reddish suffusion is seen. The individual featured in these two photos was found in the western Sandhills (near Hyannis) and is one of the individuals that I dug from their midday burrows (see Sand Hills Success). Had I not been clued into this behavior when I visited this site, I would have left with only the single individual that was seen at the surface. That individual was captured immediately, and further searching for active adults to take photographs of were unsuccessful – until I started digging, that is. Unfortunately, adults that have just been caught or dug out of their burrows aren’t the most cooperative photography subjects, so one of them was kept alive and placed in a terrarium upon my return to St. Louis. (These photos were taken about a week after I returned, and the individual lived for another seven weeks on a diet of 3rd instar fall armyworm and black cutworm larvae. I eventually trained it to grab larvae directly from the forceps – very entertaining indeed! Also, while these photos from the terrarium confines are adequate for illustrating the species, I think they still lack that undefinable spark that is caputured in true field photographs with unmanipulated individuals – compare to this photo).

Cicindela limbata, with its five recognized subspecies1, has one of the more interesting distributions of North American species (see Pearson et al. 2006). In the main area of distribution, the southernmost populations, distributed through most of Nebraska and adjacent areas of Wyoming and South Dakota, are considered nominotypical. A distributional gap to the north separates these populations from Nebraska, Grant Co., nr. Hyannis, 3.4 mi S Hwy 2 on Hwy 61, 26.ix.2008, coll. T.C.MacRaesubspecies nympha, which occurs in sand habitats of northern Montana and North Dakota and further northward into the Canadian Prairie Provinces. Individuals from these populations exhibit even greater development of the white maculations but darker intervening areas. Another distributional gap separates nympha from subspecies hyperborea, which (as its name suggests) occurs even further north in open sand habitats in the pine and poplar forests of northern Alberta and Saskatchewan and adjacent areas of the Northwest Territories. Subspecies hyperborea is characterized by its greatly reduced white maculations (thus, exhibiting expanded dark areas) and overall smaller size, both of which may be regarded as heat conservation adaptations for the far boreal climate in which it lives.

1 Excluding the federally endangered Cicindela albissima (Coral Pink Sand Dunes tiger beetle), which was recently elevated to species status based on mitochondrial DNA evidence (Morgan et al. 2000).

The fragmented nature of the main limbata population in the upper Great Plains and into the boreal forests is, in itself, interesting enough. Even more interesting, however, are the existence of two small and highly disjunct populations far removed from the main limbata population. One of these is known from Labrador – almost 3,000 miles to the east! Originally referred to subspecies hyperborea, this population was theorized to possibly represent an accidental introduction since individuals appeared to be restricted to open sand habitats within 70 km of the Goose Bay airport (Larson 1986, Pearson et al. 2006). However, careful examination of individuals from this population revealed subspecific differences in maculation (intermediate between hyperborea and nominotypical limbata), lending support to the hypothesis that it is a naturally occurring population and resulting in its description as a distinct subspecies, labradorensis (Johnson 1990). Recent analysis of mitochondrial DNA sequences provided additional support for this subspecies as a distinct entity (Knisley et al. 2008), and newly published field observations by tiger beetle afficionados Dave Brzoska and John Stamatov (2008) conducted 19 years after the initial discovery of the population suggest it is well established in suitable habitats much more distant from Goose Bay than originally reported. This accumulation of evidence seems to increasingly support a historical isolation rather than accidental introduction hypothesis. The fifth and final subspecies is an even more recently discovered and equally disjunct population in the Nogahabara Dunes of northwestern Alaska (Pearson et al. 2006). Although individuals from this population resemble subspecies nympha, morphological and mitochondrial DNA sequence analyses support its status as a distinct subspecies, designated nogahabarensis (Knisley et al. 2008). Such an unusual and fragmented distribution for Cicindela limbata and its subspecies is likely the result of historical changes in climate that have caused expansions and contractions of open sand habitats due to fluctuations in available moisture. The current geographical subspecies may have originated at the end of the mid-Holocene hypsithermal (or Holocene Climatic Optimum) some 5,000 years ago, when previously expansive open sand habitats would have begun shrinking and fragmenting as a result of declining temperatures and increasing moisture regimes.

REFERENCES

Brzoska, D. W. and J. Stamatov. 2008. A trip to Goose Bay, Labrador, Canada. Cicindela 40(3):47-52.

Johnson, W. 1990. A new subspecies of Cicindela limbata Say from Labrador (Coleoptera: Cicindelidae). Le Naturaliste Canadien 116(4) [dated 1989]:261-266.

Larson, D. J. 1986. The tiger beetle, Cicindela limbata hyperborea LeConte, in Goose Bay, Labrador (Coleoptera: Cicindelidae). The Coleopterists Bulletin 40(3):249-250.

Knisley, C. B., M. R. Woodcock and A. Vogler. 2008. A new subspecies of Cicindela limbata (Coleoptera: Cicindelidae) from Alaska and further review of the maritima group by using mitochondrial DNA analysis. Annals of the Entomological Society of America 101(2):277-288.

Morgan, M., C. B. Knisley and A. Vogler. 2000. New taxonomic status of the endangered tiger beetle Cicindela limbata albissima (Coleoptera: Cicindelidae): evidence from mtDNA. Annals of the Entomological Society of America 93(5):1108-1115.

Pearson, D. L., C. B. Knisley and C. J. Kazilek. 2006. A Field Guide to the Tiger Beetles of the United States and Canada. Oxford University Press, New York, 227 pp.

“My favorite bettle”

Today’s essay is by guest blogger (and perhaps future entomologist), Madison MacRae. Currently a 3rd grade student at Pond Elementary School, Madison’s interests include ice skating, tetherball, basketball, piano, dancing, singing, and hiking/bug collecting with her dad. Next year they will be something else. Madison would like to be a grade school teacher when she grows up. She would also like to be a nurse… and a fire fighter… and a football player. This is Madison’s second guest contribution to Beetles In The Bush, the first appearing on February 6, 2008 where she discussed the job responsibilities of a professional entomologist. For today’s contribution, Madison will be discussing one of the insects she saw on a visit to Missouri’s sand prairies back in early September [Ed. note: the insect in question appears to be an intergrade population of Cicindela scutellaris, characterized by their green coloration (unicolor influence) with variable maculation (lecontei influence)]. The original article was submitted as school work (with no prompting or prior knowledge by her dad!) and is reprinted here by the kind permission of its author.

MacRae, M. I.  2008.  My favorite bettle.  Privately published, 1 p., 1 color pl.

Cicindela scutellaris lecontei x scutellaris unicolor intergrades in southeast Missouri

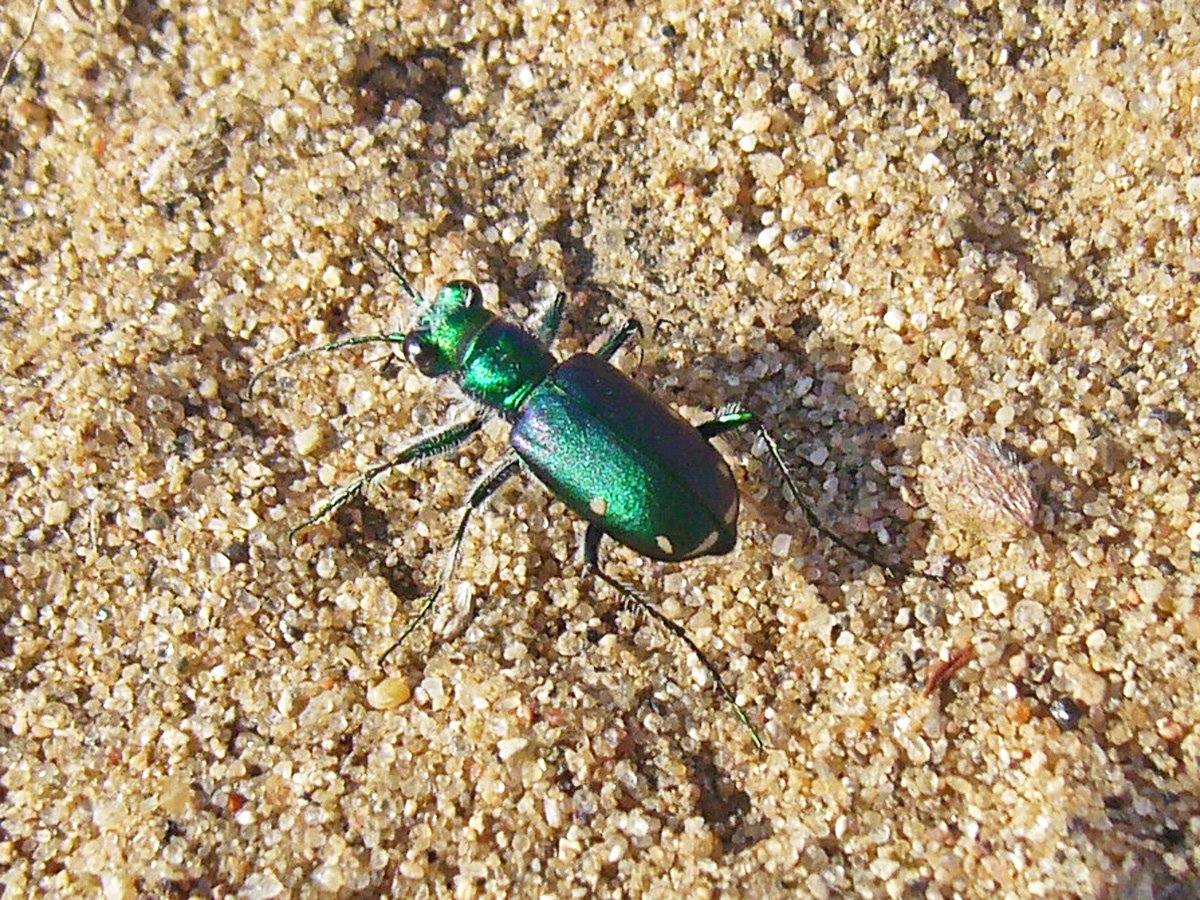
An individual from Sand Prairie Conservation Area.  Note the uniform blue-gray coloration and complete lack of maculations, making this individual indistinguishable from true unicolor.Cicindela scutellaris (festive tiger beetle) is widely distributed in the U.S., having been recorded from most areas east of the Rocky Mountains except Appalachia, the lower Mississippi River delta, and south Florida. Within this range, the species occupies deep, dry sand habitats without standing water. It is often found in the company of Cicindela formosa (big sand tiger beetle), whose range largely coincides with that of C. scutellaris (except the southeastern Coastal Plain). More than any other North American Cicindela, populations of this species show extraordinary variability in color across its range of distribution. Seven geographically recognizable subspecies are generally accepted, with considerable variation evident within some of these and along zones of contact between them.

An individual from further south on the Sikeston Ridge (~20 mi S of Sand Prairie Conservation Area).  Note the generally blue-green coloration as in unicolor, but it also exhibits fairly well developed maculations and a suffusion of maroon color on the elytra - distinct influences from subspecies lecontei.The greatest portion of the species’ range is occupied by nominotypical populations in the Great Plains and subspecies lecontei in the Midwest and northeast. Similar to what I’ve noted in previous posts for other species, a broad zone of intergradation between these two subspecies occurs along the upper Missouri River. Other subspecies occupy more limited ranges along the upper Atlantic Coast (rugifrons), southeastern Coastal Plain (unicolor), eastern Texas and adjacent areas of northwestern Louisiana and southwestern Arkansas (rugata), and north-central Texas (flavoviridis), and the highly restricted and disjunct yampae is found only in a small area of northwestern Colorado. Populations in the upper Midwest and Canadian prairie are sometimes regarded as distinct from lecontei (designated as subspecies criddlei) due to their broadly coalesced marginal elyral maculations, and an apparently disjunct population of small, blue individuals in south Texas may also be regarded as subspecifically distinct.

Another individual from Sand Prairie Conservation Area.  It is similar to the unicolor-type individual in Photo 1 but also exhibits small maculations derived from its lecontei influence.Although Missouri lies well within the boundaries of its range, this species has been found in only three widely-separated parts of the state – near the Missouri River in the northwest part of the state, near the Mississippi River in the extreme northeast corner, and in the southeastern lowlands (formally known as the Mississippi River Alluvial Basin). The two northern Missouri populations are assignable to and typical of lecontei, with their uniform dull maroon to olive green coloration and continuous to near-continuous ivory-colored border around the outer edge of the elytra. Additional dry sand habitats occur along the lower Missouri River in central and east-central Missouri and along some of the larger rivers that drain the Ozark Highlands; however, this species has not been located in these habitats despite their apparent suitability and occurrence of C. formosa with which it frequently co-occurs. The reasons for this distributional gap between the northern and southern populations – some 400 miles in width – remain a mystery. The southeastern Missouri population is not clearly assignable to any subspecies, apparently representing an intergrade between lecontei to the north and unicolor to the south. Accordingly, individuals from this area are known by the unwieldy appellative “Cicindela scutellaris lecontei x scutellaris unicolor intergrade.” Pearson et al. (2005) states that intergrades between lecontei and unicolor are evident only in northern “Missouri” (an obvious error for Mississippi) and Tennessee. Thus, the existence of intergrades in southeastern Missouri suggests that the zone of intergradation extends further north than previously realized.

A second individual from ~20 mi S of Sand Prairie Conservation Area.  Similar to the individual in Photo 2 except with smaller maculations.  Note the gorgeous suffusion of maroon, especially on head and pronotum - a spectacular individual.Prior to this season, I had located two main population centers in the southeastern lowlands – one at Holly Ridge Conservation Area in Stoddard County, and another at Sand Pond Conservation Area in Ripley County. Holly Ridge is located on Crowley’s Ridge – an erosional remnant of Tertiary sand and aggregate sediments left behind by the late Pleistocene glacial meltwaters whose scouring action formed the surrounding lowlands, while the sandy sediments at Sand Pond were deposited west of Crowley’s Ridge along the southeastern escarpment of the Ozark Highlands during that same period. These erosional and depositional events created the deep, dry sand habitats that Cicindela scutellaris requires. I had known also about the Sikeston Sand Ridge further to the east – another erosional remnant of Tertiary sands deposited by the ancient Ohio River – but had not explored it closely until this season when I initiated my surveys at Sand Prairie Conservation Area. I expected Cicindela scutellaris might occur here, and in my first fall visit in early September I found two individuals in the sand barrens (alongside Cicindela formosa). Another individual was seen here in early October, but more robust populations were observed at a small, high-quality sand prairie remnant (last photo) further to the south along the Sikeston Ridge, and around eroded sand barrens behind private residences still further to the south. Clearly, the species is well-established in the southeastern lowlands wherever open dry sand habitats can be found.

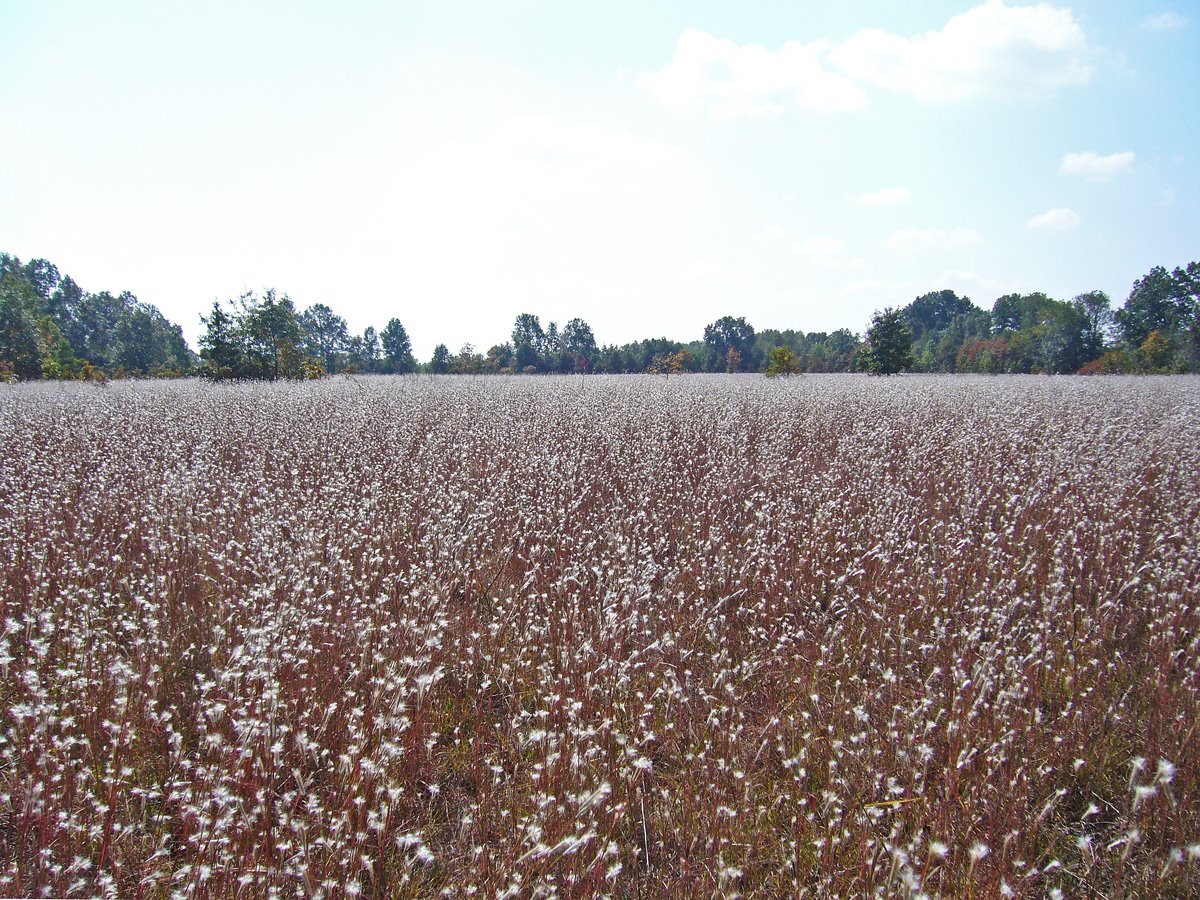
Sand prairie habitat for Cicindela scutellaris in southeast Missouri.  Note the well-spaced clumps of grass, in this case splitbeard bluestem.The individuals shown here exemplify the range of variation exhibited by Cicindela scutellaris populations in southeast Missouri. They greatly resemble subspecies unicolor by their uniform shiny blue-green coloration. Indeed, the individual in the first photo might well be classified as such due to the complete absence of white maculations along the elytral border. Most individuals, however, show varying development of such maculations, ranging from small disconneted spots to the more developed apical “C”-shaped mark – clearly an influence from subspecies lecontei. Another apparent lecontei influence is the suffusion of wine-red or maroon coloration that can be seen on the head, pronotum, and elytra of the individuals in photos 2 and 4. These characters make this population divergent from the typically monochromic unicolor (as its name suggests). Because of their bright green coloration and white maculations, individuals in this population greatly resemble subspecies rugifrons, but that subspecies is limited to the northern Atlantic seaboard. They also resemble the common and widespread Cicindela sexguttata (six-spotted tiger beetle) but can be distinguished from that species by the more noticeably domed profile of the elytra, rounded rather than tapered elytral apex, and dark labrum of the female (both sexes of C. sexguttata have a white labrum).

There is one additional sand ridge in Missouri’s southeastern lowlands – the Malden Ridge. This sand ridge occurs south of Crowley’s Ridge and is much smaller than the Sikeston Ridge. No significant remnant habitats remain on the Malden Ridge, but it is possible that sufficient areas of open sand remain that might support populations of C. scutellaris. Determining whether this is true will require some time studying Google Earth and even more time on the ground to search them out. If they do exist, however, it will be interesting to see what level of influence by lecontei is exhibited in this most southerly of Missouri populations. Only spring will tell!

A sand prairie autumn

Splitbeard bluestem seed headsAsk any astronomer when autumn begins, and they will likely tell you it begins at the autumnal equinox – when shortening days and lengthening nights become equal as the sun crosses over the celestial equator. According to them, fall began this year on September 22 – at 11:44:18 A.M. EDT, to be precise. I agree that autumn begins at a precise moment, but it is not at the equinox. Rather, it is that unpredictable moment when a sudden crispness in the air is felt, when the sky somehow seems bluer and shadows seem sharper, and hints of yellow – ever so subtle – start to appear in the landscape. Butterfly pea blossomIn Missouri, with its middle latitudes, this usually happens a few weeks before the equinox, as August is waning into September. It is a moment that goes unnoticed by many, especially those whose lives and livelihoods have lost all connection with the natural world. To plants and animals, however, it is a clear signal – a signal to begin making preparations for the long cold months of winter that lie ahead. Plants that have not yet flowered begin to do so in earnest, while those that have shift energy reserves into developing seeds. Animals take advantage of their final opportunities to feed before enduring the scarcities of winter, digging in to sleep through them, or abandoning altogether and migrating to warmer climes. Insects begin hastily provisioning nests for their broods or laying eggs – tiny capsules of life that survive the harsh winter before hatching in spring and beginning the cycle anew.
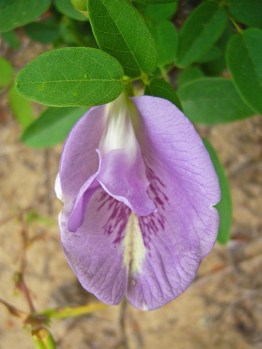
Sand prairie in early September.Sand prairie in early October.  Note abundance of splitbeard bluestem seed heads.Across much of Missouri, in the Ozark Highlands and in riparian ribbons dissecting the northern Plains, autumn brings an increasingly intense display of reds, purples, oranges, and yellows, as the leaves of deciduous hardwoods begin breaking down their chlorophyll to unmask underlying anthocyanins and other pigments. Small southern jointweedIn Missouri’s remnant prairies, seas of verdant green morph to muted shades of amber, tawny, and beige. This subtle transformation is even more spectacular in the critically imperiled sand prairies of the Southeast Lowlands, where stands of splitbeard bluestem (Andropogon ternaries – above) turn a rich russet color while fluffy, white seed heads (1st paragraph, 1st photo) appear along the length of each stem, evoking images of shooting fireworks. Small southern jointweed (Polygonella americana – right) finds a home at the northern extent of its distribution in these prairie remnants and in similar habitats in nearby Crowley’s Ridge, blooming in profusion once the cooler nights arrive. Butterfly pea (Clitoria mariana – 1st paragraph, 2nd photo) blooms add a gorgeous splash of soft purple in contrast to the muted colors of the plants around them.
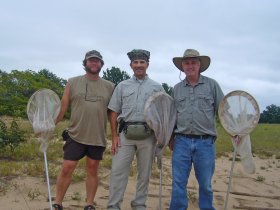
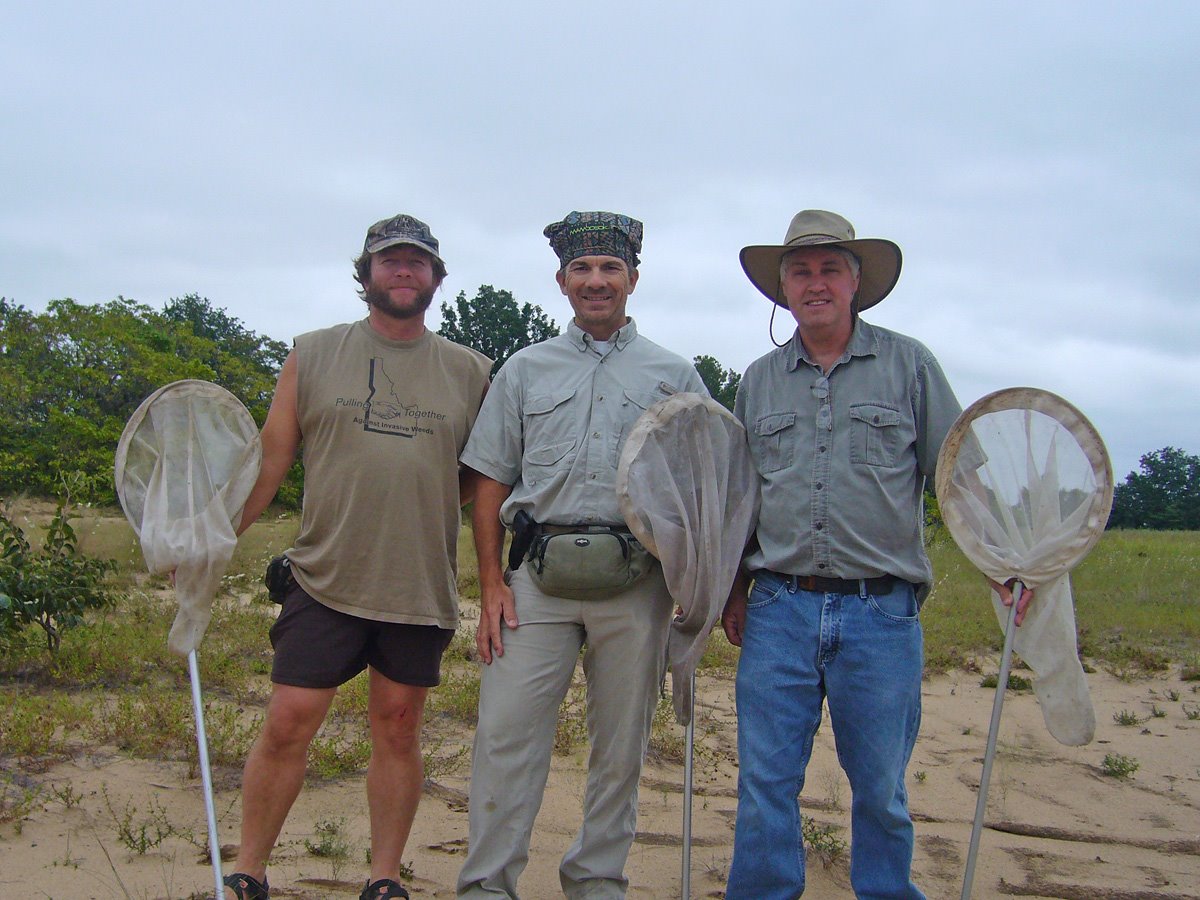
Kent Fothergill, Ted MacRae, and Rich ThomaAfter first becoming acquainted with Missouri’s sand prairies this past summer, I knew a fall trip (or two) would be in order. The extensive deep, dry sand barrens were ideal habitat for sand-loving insects, including certain spring/fall species of tiger beetles that would not be active during the summer months. The cooler nights and crisp air of early fall make insect collecting extraordinarily pleasurable, so it took little effort to convince friends and colleagues Kent and Rich to join me on another excursion to these extraordinary remnant habitats, along with my (then 8 yr-old) daughter Madison (who would likely characterize this as “tallgrass” prairie). Madison MacRae, age 9 (almost)I was, as ever, on the lookout for tiger beetles; however, temperatures were cool, skies were overcast, and the fall season was just beginning, greatly limiting tiger beetle activity during this first fall visit. We did see one Cicindela formosa (big sand tiger beetle), which cooperated fully for a nice series of photographs. We also found single specimens of the annoyingly ubiquitous C. punctulata (punctured tiger beetle) and a curiously out-of-place C. duodecimguttata (12-spotted tiger beetle), which must have flown some distance from the nearest dark, muddy streambank that it surely prefers. Of greatest interest, we found two specimens of C. scutellaris (festive tiger beetle), which in this part of Missouri is represented by a population presenting a curious mix of influences from two different subspecies (more on this in a later post…). Despite the scarcity of tiger beetles, other insects were present in great diversity, some of which I share with you here.

Ululodes macleayanusThis bizarre creature, sitting on the stem of plains snakecotton (Froelichia floridana), is actually a neuropteran insect called an owlfly (family Ascalaphidae). Looking like a cross between a dragonfly and a butterfly due to its overly large eyes and many-veined wings but with long, clubbed antennae, this individual is demonstrating the cryptic resting posture they often assume with the abdomen projecting from the perch and resembling a twig. The divided eyes identify this individual as belonging to the genus Ululodes, and Dr. John D. Oswald (Texas A&M University) has kindly identified the species as U. macleayanus. As is true of many groups of insects, their taxonomy is far from completely understood. Larvae of these basal holometabolans are predaceous, lying on the ground with their large trap-jaws held wide open and often camouflaging themselves with sand and debris while waiting for prey. The slightest contact with the jaws springs them shut, and within a few minutes the prey is paralyzed and can be sucked dry at the larva’s leisure.

Ant lion, possibly in the genus Myrmeleon.Another family of neuropteran insects closely related to owlflies are antlions (family Myrmeleontidae, sometimes misspelled “Myrmeleonidae”). This individual (resting lower down on the very same F. floridana stem) may be in the genus Myrmeleon, but my wanting expertise doesn’t allow a more conclusive identification [edit 4/12/09 – John D. Oswald has identified the species as Myrmeleon immaculatus]. Strictly speaking, the term “antlion” applies to the larval form of the members of this family, all of whom create pits in sandy soils to trap ants and other small insects, thus, it’s occurrence in the sand prairie is not surprising. Larvae lie in wait beneath the sand at the bottom of the pit, flipping sand on the hapless prey to prevent it from escaping until they can impale it with their large, sickle-shaped jaws, inject digestive enzymes that ‘pre-digest’ the prey’s tissues, and suck out the liquifying contents. Finding larvae is not easy – even when pits are located and dug up, the larvae lie motionless and are often covered with a layer of sand that makes them almost impossible to detect. I’ve tried digging up pits several times and have failed as yet to find one. Larvae are also sometimes referred to as “doodlebugs” in reference to the winding, spiralling trails that the larvae leave in the sand while searching for a good trap location – these trails look like someone has doodled in the sand.

Bembix americanaThis digger wasp, Bembix americana (ID confirmed by Matthias Buck), was common on the barren sand exposures, where they dig burrows into the loose sand. Formerly included in the family Sphecidae (containing the better-known “cicada killer”), members of this group are now placed in their own family (Crabronidae). Adult females provision their nest with flies, which they catch and sting to paralyze before dragging it down into the burrow. As is common with the social hymenoptera such as bees and paper wasps, these solitary wasps engage in active parental care by providing greater number of prey as the larva grows. As many as twenty flies might be needed for a single larva. I found the burrows of these wasps at first difficult to distinguish from those created by adults of the tiger beetles I so desired, but eventually learned to distinguish them by their rounder shape and coarser, “pile” rather than “fanned” diggings (see this post for more on this subject).

Stichopogon trifasciatusRobber flies (family Asilidae) are a favorite group of mine (or, at least, as favorite as a non-coleopteran group can be). This small species, Stichopogon trifasciatus (ID confirmed by Herschel Raney), was also common on the barren sandy surface. The specific epithet refers to the three bands of alternating light and dark bands on the abdomen. Many species in this family are broadly distributed but have fairly restrictive ecological requirements, resulting in rather localized occurrences within their distribution. Stichopogon trifasciatus occurs throughout North America and south into the Neotropics wherever barren, sandy or gravely areas near water can be found. Adults are deadly predators, swooping down on spiders, flies and other small insects and “stabbing” them with their stout beak.

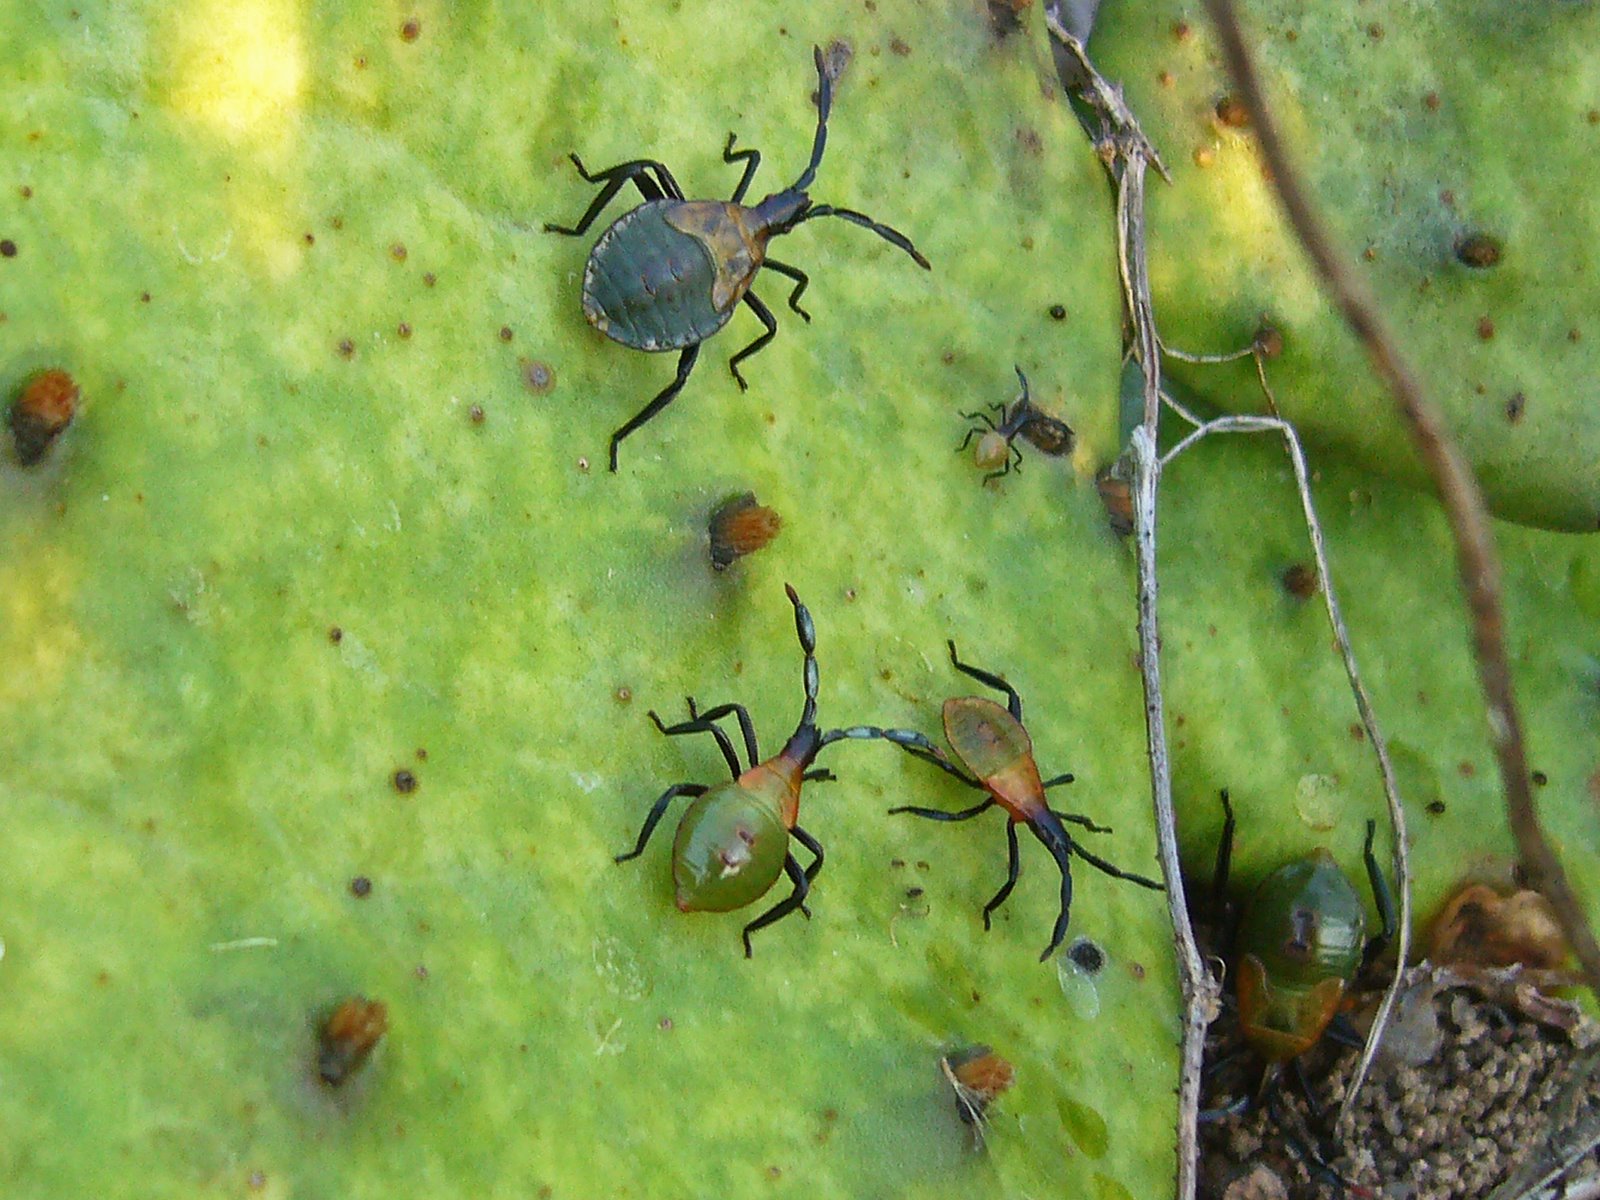
Chelinidea vittigerPrickly pear cactus (Opuntia humifusa) grows abundantly in the sandy soil amongst the clumps of bluestem, and on the pads were these nymphs of Chelinidea vittiger (cactus bug, family Coreidae). This wide-ranging species occurs across the U.S. and southward to northern Mexico wherever prickly pear hosts can be found. This species can either be considered a beneficial or a pest, depending upon perspective. On the one hand, it serves as a minor component in a pest complex that prevents prickly pear from aggressively overtaking rangelands in North America; however, prickly pear is used by ranchers as emergency forage, and fruits and spineless pads are also sometimes harvested for produce. In Missouri, O. humifusa is a non-aggressive component of glades, prairies, and sand and gravel washes, making C. vittiger an interesting member of the states natural diversity.
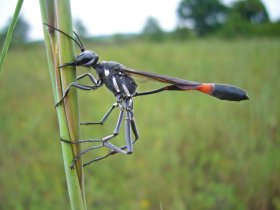
Ammophila sp., possibly A. proceraThis wasp in the genus Ammophila (perhaps A. procera as suggested by Herschel Raney) was found clinging by its jaws to a bluestem stem in the cool morning, where it presumably spent the night. One of the true sphecid (or “thread-waist”) wasps, A. procera is a widespread and common species in eastern North America. One of the largest members of the genus, its distinctive, bold silver dashes on the thorax distinguish it from most other sympatric congeners. Similar to the habits of most other aculeate wasp groups, this species captures and paralyzes sawfly or lepidopteran caterpillars to serve as food for its developing brood. Females dig burrows and lay eggs on the paralyzed hosts with which the nests have been provisioned. Adults are also found commonly on flowers, presumably to feed on nectar and/or pollen.

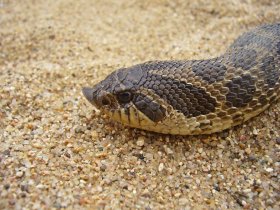
Dusty hog-nosed snakeRich is a bit of herpatologist, so when he brought this hog-nosed snake to our attention we all had a good time pestering it to try to get it to turn upside down and play dead. I had never seen a hog-nosed snake before but knew of its habit of rolling over and opening its mouth with its tongue hanging out when disturbed, even flopping right back over when turned rightside up or staying limp when picked up. We succeeded in getting it to emit its foul musky smell, but much to our disappointment it never did play dead, instead using its shovel-shaped snout to dig into the sand. Dusty hog-nosed snake - head closeupWe had assumed this was the common and widespread eastern hog-nosed snake (Heterodon platirhinos); however, in our attempts to turn it over I noticed its black and orange checker patterned belly. I later learned this to be characteristic of the dusky hog-nosed snake (H. nasicus gloydi), only recently discovered in the sand prairies of southeast Missouri and regarded as critically imperiled in the state due to the near complete destruction of such habitats. Disjunct from the main population further west, its continued survival in Missouri depends upon the survival of these small sand prairie remnants in the Southeast Lowlands.
It’s a girl!

I’ve been interested in collecting insects since I was 10 years old, and my current collection dates back to spring semester 1978 when, after finally declaring a major, I kicked off my life as an entomologist with Entomology 101. I did my graduate work on the now-defunct Homoptera (I just can’t call them hemipterans), using laboratory rearing to figure out life history details of several species of leafhoppers. Although my allegiance would soon switch to beetles (where it has remained ever since), my interest in rearing insects would persist. It wasn’t long before I began rearing wood boring beetles as a way of studying their distributions and host plant associations. I’ve reared beetles from literally hundreds of batches of wood – buprestids, cerambycids, bostrichids, clerids, ostomids, you name it – if it breeds in wood, I’ve reared it. Not to mention the parasitic hymenopterans and even predaceous asilids associated with them. Rearing has been part of my professional life as well. In the early part of my career in industry, I supervised an insectary that maintained laboratory colonies of nearly two dozen arthropod species to support research. We reared moths, beetles, flies, roaches, aphids – even mites and nematodes. However, despite having reared hundreds of species of insects, I had never reared a tiger beetle – until now!

This little gal – a gorgeous individual representing Cicindela limbalis (common claybank tiger beetle) – was waiting for me when I returned from my recent trip to western Nebraska and South Dakota. I had collected her as a 3rd instar larva from her burrow atop a steep clay bank in western Missouri, where my colleague and I were conducting our survey for Cicindela pruinina (now Dromochorus pruininus). I had entertained the hope that it might prove to be that species, but the abundance of larval burrows within this patch of habitat – where C. pruinina had not been seen – and the fact that they contained mostly 3rd instars suggested it would prove to be one of the spring-fall clay associated species. After fishing her from her burrow, I filled an empty Starbuck’s Frappucinno bottle (there is, apparently, only one place in the Ozarks where availability of good coffee obviates the need to resort to a cold, sugary, “coffee-flavored” drink in the morning) with native clay and dropped her in, where she immediately proceeded to dig a new burrow. She was thoughtful enough to dig her burrow right down along the glass so that I could keep an eye on her over the next several weeks, occasionally dropping in a fat fall armyworm larva and watching it meet its gruesome yet mercifully quick death. A few weeks before my trip, she sealed up her burrow and disappeared from view. Curious (and impatient), I emptied the soil from the bottle and found her down at the bottom, quiescent but apparently healthy. I put the soil back into the bottle and dropped her in, and she immediately dug a new burrow, sealed it up, and disappeared from view once again. My curiosity satisfied, I had an easier time leaving her alone after that, and when I returned from my trip, there she was.

Cicindela limbalis occurs throughout Missouri on eroded or sparsely vegetated clay soils, although it is less common in the southern Ozark Highlands – being largely replaced by Cicindela splendida (splendid tiger beetle). I’ve most often encountered C. limbalis on roadside embankments, along 2-tracks through open forest and woodland, and in glade habitats. This individual shows the greatly reduced elytral maculations that are typical of populations found throughout most of Missouri – only in the extreme northern tier of counties is the full pattern of maculation expressed (as exemplified by this individual from central Nebraska). At one time, this reduced maculation was the basis for recognition as a separate subspecies (C. limbalis transversa); however, no distinct geographical forms are currently recognized for this species (unusual in cicindelid taxonomy). Regardless of her taxonomic identity, I’m enjoying watching my new pet – she now occupies a larger, roomier terrarium filled with native clay, into which she has dug a burrow and spends most of her time sitting at its entrance. As she did when she was a 3rd instar, she enjoys a fat fall armyworm larva for lunch every few days. She will eventually take up permanent residence in a neat row inside a wooden, glass-topped box, but for now I’m going to do everything I can to delay that fate. Of all the many thousands of insects that I’ve reared over the years, she is my favorite.